NAD+ & NMN for Longevity and Sirtuin Activation
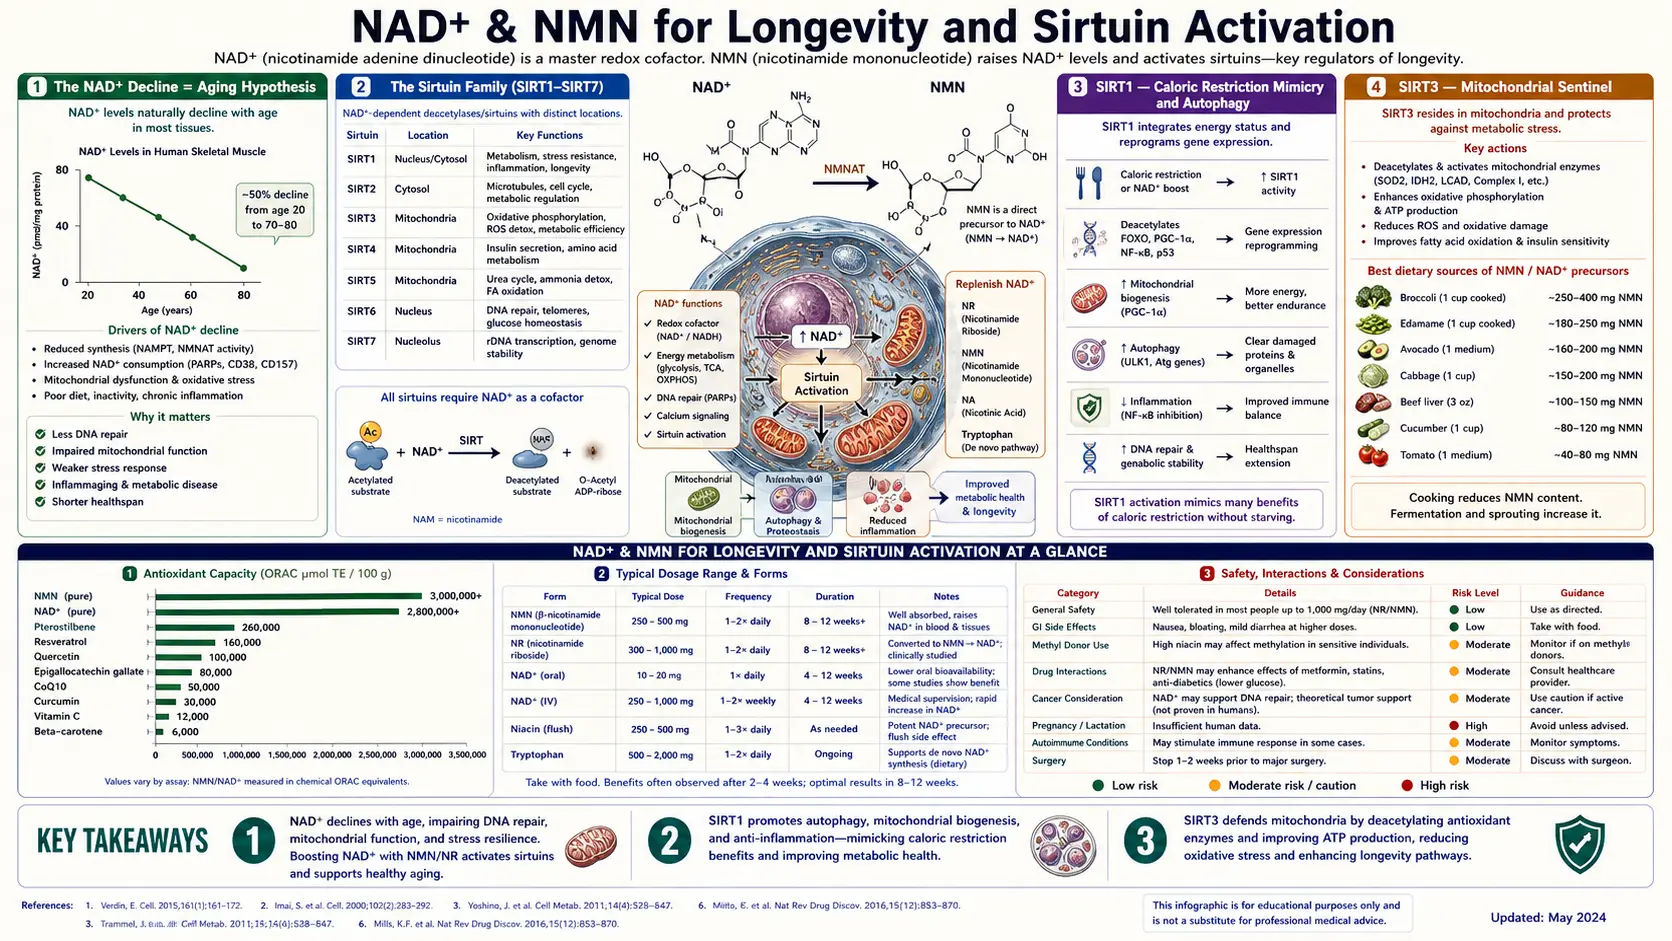
NAD+ precursors are among the most studied candidate "longevity supplements," and they are tied to a specific biological theory of aging. Laboratories including David Sinclair's at Harvard Medical School linked NAD+ availability to the sirtuin family of enzymes, and the resulting model — declining NAD+ limits sirtuins, which in turn allows epigenetic decay and mitochondrial dysfunction to accumulate — is the main framework used to explain why NAD+ precursors are studied for aging. It rests mostly on cell and mouse work. This deep-dive walks through the seven mammalian sirtuins, the SIRT1/SIRT3/SIRT6 axis most studied in aging research, the mouse lifespan results, the Sinclair Information Theory of Aging, the Brenner vs Sinclair NR-vs-NMN debate, and what is and is not shown in humans.
Table of Contents
- The NAD+ Decline = Aging Hypothesis
- The Sirtuin Family (SIRT1–SIRT7)
- SIRT1 — Caloric Restriction Mimicry and Autophagy
- SIRT3 — Mitochondrial Sentinel
- SIRT6 — Telomeres, DNA Repair, and Lifespan
- The David Sinclair Lab Program
- The Information Theory of Aging
- The Brenner vs Sinclair NR-vs-NMN Debate
- What Is and Is Not Proven in Humans
- Combinations Discussed for Sirtuin Activation
- Safety Findings and Open Questions
- Key Research Papers
- Connections
The NAD+ Decline = Aging Hypothesis
The central premise of NAD+-centric longevity science is that NAD+ falls with age and that the fall matters. The evidence differs by species, tissue and measurement. In aged mice, isotope tracing across tissues found a median decrease of about 30%, with NAD+ production maintained; the authors called the decline with normal aging "relatively subtle" (McReynolds and colleagues, 2021). In human tissues, lower NAD+ with age has been reported in skin (Massudi and colleagues, 2012), brain (Zhu and colleagues, 2015) and skeletal muscle (Janssens and colleagues, 2022). Human blood data are mixed: one study found lower plasma NAD+ with age, a study of 1,518 people found a decline in men but not women, and a 2026 study of seven cohorts found whole-blood NAD+ "remarkably stable with age" (Trętowicz and colleagues, 2026). A frequently quoted figure of a 50% fall by middle age was not found as a measured human result. Lower NAD+ has been linked to mitochondrial dysfunction, genomic instability, cellular senescence, inflammation and impaired stem-cell function, mainly in animal and cell studies.
The hypothesis is that this NAD+ decline is not just a marker of aging but a cause of it. The reasoning runs as follows:
- Sirtuins, PARPs, and CD38 all consume NAD+ as a substrate.
- As DNA damage accumulates with age, PARPs consume more NAD+ to flag and repair breaks.
- As inflammaging develops, CD38 on inflammatory immune cells rises in mice, consuming more NAD+; in mouse experiments CD38 was required for the age-related decline (Camacho-Pereira and colleagues, 2016).
- The salvage enzyme NAMPT has been reported to fall in some aged mouse tissues, reducing supply.
- The net result, in this model, is a smaller pool of NAD+ available to the sirtuins.
- Sirtuins, short of substrate, maintain their epigenetic, metabolic, and DNA-repair functions less well.
- Cellular function degrades, contributing to the visible phenotype of aging.
If the chain is correct, restoring NAD+ would support sirtuin function and could slow aspects of biological aging. In this framing, NMN and NR are studied not as vitamin replacement but as substrate replenishment for enzymes whose substrate is proposed to become limiting.
The hypothesis rests mainly on mouse data. The final step — that boosting NAD+ in humans extends healthspan or lifespan — has not been shown. Short human trials consistently show that NMN and NR raise NAD+ or its metabolites in blood; effects on clinical outcomes have been small, mixed or absent, and no study has measured lifespan in people taking NMN or NR.
The Sirtuin Family (SIRT1–SIRT7)
Mammals have seven sirtuins, named SIRT1 through SIRT7. All seven require NAD+ as a stoichiometric cofactor — one NAD+ molecule is consumed for each deacetylation reaction. They differ in subcellular location and substrate preference, which determines their specific roles in cellular biology.
| Sirtuin | Location | Primary Activities |
|---|---|---|
| SIRT1 | Nucleus, cytoplasm | Deacetylates p53, FOXO, PGC-1α, NF-kB; promotes autophagy; mediates caloric restriction |
| SIRT2 | Cytoplasm | Tubulin deacetylase; cell-cycle control; oligodendrocyte function |
| SIRT3 | Mitochondrial matrix | Master mitochondrial deacetylase; regulates electron transport, antioxidant defenses, fatty acid oxidation |
| SIRT4 | Mitochondrial matrix | ADP-ribosyltransferase rather than deacetylase; regulates glutamate dehydrogenase |
| SIRT5 | Mitochondrial matrix | Demalonylates, desuccinylates, deglutarylates rather than classic deacetylation |
| SIRT6 | Nucleus, chromatin | DNA double-strand break repair, telomere maintenance, glucose metabolism regulation |
| SIRT7 | Nucleolus | Ribosomal DNA stability, transcription regulation |
For longevity purposes, the three that matter most are SIRT1 (the master metabolic sensor), SIRT3 (the mitochondrial protector), and SIRT6 (the chromatin guardian). The next three sections examine each in detail.
SIRT1 — Caloric Restriction Mimicry and Autophagy
SIRT1 is the mammalian counterpart of yeast Sir2, which Leonard Guarente's laboratory at MIT linked to yeast aging in the 1990s. Sirtuins were proposed as a molecular explanation for why caloric restriction extends lifespan in yeast and other organisms: in this model, caloric restriction raises the cellular NAD+/NADH ratio, activating SIRT1, which then deacetylates many downstream targets. How much of caloric restriction's effect in mammals runs through sirtuins is still debated.
Key SIRT1 substrates and their downstream effects:
- p53 — SIRT1 deacetylates p53 at lysine 382, reducing its pro-apoptotic activity and shifting cells toward survival rather than death under stress. This is part of how caloric restriction protects against age-related cell loss.
- FOXO transcription factors — SIRT1 deacetylation of FOXO1, FOXO3, and FOXO4 promotes their stress-resistance and antioxidant gene programs, including superoxide dismutase 2 (SOD2) and catalase. This is a major reason SIRT1 activation enhances cellular resilience.
- PGC-1α — SIRT1 deacetylates and activates PGC-1α, the master regulator of mitochondrial biogenesis. The result is more mitochondria per cell, better-organized respiratory chains, and improved oxidative metabolism — the same phenotype induced by exercise.
- NF-kB — SIRT1 deacetylates the p65 subunit of NF-kB, reducing inflammatory gene transcription. This is the molecular basis for SIRT1's anti-inflammaging effects.
- ATG proteins and LC3 — SIRT1 promotes the assembly of the autophagy machinery, enabling cells to clear damaged proteins and organelles.
The proposed link to NAD+ supplementation is that SIRT1 activity depends on NAD+ availability, so raising the NAD+ pool with NMN or NR could enhance SIRT1 function and produce caloric-restriction-like effects. This is the basis for describing NMN as a "caloric restriction mimetic"; it has not been shown in people. In mice, moderate whole-body SIRT1 overexpression produced healthier aging and fewer spontaneous cancers but did not extend lifespan (Herranz and colleagues, 2010), while SIRT1 overexpression limited to the brain did extend lifespan in both sexes (Satoh and colleagues, 2013).
SIRT3 — Mitochondrial Sentinel
SIRT3 lives in the mitochondrial matrix and is the main deacetylase for a large number of mitochondrial proteins. Its substrates include:
- Long-chain acyl-CoA dehydrogenase (LCAD) — SIRT3 deacetylates LCAD, enabling efficient fatty acid oxidation. SIRT3 knockout mice cannot oxidize long-chain fatty acids properly and develop fatty liver under fasting.
- Manganese superoxide dismutase (MnSOD/SOD2) — SIRT3 deacetylates SOD2, activating the principal mitochondrial antioxidant defense. Reduced SIRT3 activity (as in aged tissues) leaves mitochondrial superoxide unchecked.
- Complex I and Complex II subunits — SIRT3 deacetylates respiratory chain subunits, supporting normal electron flow and ATP production.
- Isocitrate dehydrogenase 2 (IDH2) — SIRT3 deacetylation of IDH2 supports NADPH regeneration, which is required for glutathione recycling.
In mice, CD38, the NAD+ consumer that rises with age, was required for the age-related NAD+ decline and for mitochondrial dysfunction through a SIRT3-dependent mechanism (Camacho-Pereira and colleagues, 2016); a 2023 study by some of the same researchers reported that CD38 may not dictate NAD+ levels in brain mitochondria of aged mice. NAD+ repletion is proposed to act on this pathway by giving SIRT3 more substrate. In 12 older men, NR raised the muscle NAD+ metabolome but did not change mitochondrial bioenergetics (Elhassan and colleagues, 2019).
SIRT6 — Telomeres, DNA Repair, and Lifespan
SIRT6 is the sirtuin with the clearest mouse lifespan data. Mice engineered to overexpress SIRT6 lived longer — males only in a 2012 study (Kanfi and colleagues), and both sexes in a 2021 study on a different genetic background (Roichman and colleagues) — and SIRT6 knockout mice die prematurely with a phenotype resembling accelerated aging (Mostoslavsky and colleagues, 2006).
SIRT6 has three principal functions:
- Telomere chromatin maintenance — SIRT6 deacetylates histone H3 at lysine 9 (H3K9ac) and lysine 56 (H3K56ac) at telomeric chromatin, supporting the compact heterochromatin structure that protects chromosome ends. Without SIRT6, telomeric chromatin destabilizes and chromosomal ends become dysfunctional.
- DNA double-strand break repair via homologous recombination — SIRT6 is recruited to DNA breaks and facilitates the homologous recombination pathway, which is the higher-fidelity repair mechanism. Reduced SIRT6 activity shifts repair toward the more error-prone non-homologous end joining pathway, producing accumulating mutations.
- Glucose metabolism regulation — SIRT6 represses glycolytic genes via deacetylation of H3K9 at glycolysis-related promoters, biasing metabolism toward oxidative phosphorylation. Loss of SIRT6 produces a Warburg-like shift toward glycolysis, which is metabolically associated with both cancer and aging.
SIRT6 activity, like SIRT1 and SIRT3 activity, is NAD+-dependent. Researchers propose that restoring NAD+ levels in aged tissues with NMN or NR could support SIRT6 alongside the other sirtuins; this has not been measured in people. The telomere and DNA repair effects in particular are the mechanistic basis for the "NAD+ extends healthspan" framing in mouse studies.
The David Sinclair Lab Program
David Sinclair is a Professor of Genetics at Harvard Medical School and one of the scientists most associated with the case for NAD+-based interventions. His research arc moves through three phases:
Phase 1: The Sir2 / SIRT1 discovery (1995–2003)
Sinclair completed his Ph.D. in Molecular Genetics at the University of New South Wales in 1995, then joined Leonard Guarente's lab at MIT as a postdoctoral fellow. There he co-discovered a cause of yeast aging tied to genomic instability at the ribosomal DNA locus — extrachromosomal rDNA circles (Sinclair and Guarente, 1997) — and worked on Sir2 (the yeast sirtuin) as a regulator of that process. He founded his own lab at Harvard Medical School in 1999 and extended the Sir2 work into mammalian SIRT1.
Phase 2: Resveratrol and the STAC search (2003–2013)
In 2003, Sinclair's group reported that resveratrol and related molecules activated sirtuins and extended the lifespan of yeast by 70% (Howitz and colleagues, 2003), which launched a search for sirtuin-activating compounds (STACs). The mammalian results since then are mixed. Resveratrol improved health measures in mice but did not extend lifespan on a standard diet (Pearson and colleagues, 2008), and the US National Institute on Aging's Interventions Testing Program found no lifespan effect (Miller and colleagues, 2011). A 2010 study found that resveratrol and several synthetic "sirtuin activators" activated SIRT1 only with an artificial fluorescent test substrate, not with native substrates (Pacholec and colleagues, 2010); Sinclair's group later reported that activation depends on particular substrate features (Hubbard and colleagues, 2013). The synthetic activator SRT2104 extended mean and maximal lifespan of male mice on a standard diet (Mercken and colleagues, 2014). Sinclair co-founded a company built around this work, which a large pharmaceutical company bought in 2008.
Phase 3: NAD+ precursors and epigenetic reprogramming (2013–present)
Sinclair's lab then turned to NAD+ itself. A 2013 paper from his group (Gomes and colleagues, Cell) found that aging mice lost mitochondrially encoded respiratory-chain subunits through a decline in nuclear NAD+, and that raising NAD+ with NMN in old mice for one week restored mitochondrial function in muscle to that of young mice, in a SIRT1-dependent manner. Mills and colleagues (2016, Imai laboratory at Washington University) found that 12 months of NMN in normal mice suppressed age-related weight gain and improved energy metabolism, physical activity, insulin sensitivity, lipids and eye function; the study did not report a lifespan result and was not designed as a lifespan study. Sinclair's lab has more recently focused on cellular reprogramming as a more direct intervention against the epigenetic noise that he proposes drives aging, while continuing to publish on NAD+ biology.
Sinclair has publicly favoured NMN over NR, in part because his own lab's data are NMN-centric, and has said in interviews that he takes about 1 g of NMN daily along with other compounds. His public commentary has been a major driver of consumer interest in NMN; how to read that interest is part of the Brenner debate below.
The Information Theory of Aging
In his 2019 book Lifespan and a series of subsequent papers, Sinclair proposed a unifying framework he calls the Information Theory of Aging. The core idea: aging is fundamentally a loss of epigenetic information, not genetic information. Cells lose the ability to read their own DNA correctly because the epigenetic marks that tell each cell which genes to express become progressively scrambled over time.
The mechanism proposed is that DNA double-strand breaks — which occur thousands of times per cell per day from normal metabolism, radiation, and chemical stress — recruit sirtuins (particularly SIRT1) away from their normal epigenetic maintenance duties to participate in emergency repair. Each repair episode subtly perturbs the local chromatin state and leaves a small amount of epigenetic noise behind. Over decades, this accumulating noise progressively degrades cellular identity, leading to functional decline.
The implications for NAD+ supplementation under this model:
- In the model, NAD+ supplementation would reduce the "tax" that DNA damage imposes on sirtuin availability, allowing sirtuins to maintain their epigenetic maintenance functions more effectively.
- In the model, NAD+ supplementation would support SIRT6, which directs DNA repair toward the higher-fidelity homologous recombination pathway, reducing the rate of epigenetic perturbation per repair event.
- Cellular reprogramming with the Yamanaka transcription factors (OSK, omitting cMyc) may directly reverse epigenetic noise, restoring a more youthful epigenetic state — this is now the main focus of Sinclair's laboratory.
A 2023 mouse study from the laboratory, which induced DNA breaks to test the idea, is the main experimental paper behind it (Yang and colleagues, 2023). The theory is not universally accepted; competing frameworks emphasize mitochondrial decline, telomere attrition, senescent cell accumulation, or stem cell exhaustion as the primary drivers. It remains a hypothesis supported by laboratory and animal work; it has not been tested as a treatment in people.
The Brenner vs Sinclair NR-vs-NMN Debate
Charles Brenner, the biochemist whose laboratory described NR as an NAD+ precursor in 2004 (Bieganowski and Brenner, 2004), has been the most prominent scientific critic of the NMN-over-NR framing; he has served as chief scientific adviser to a company that sells NR. The Brenner critique has several components:
- Absorption and cell entry — Brenner argues that NMN, a charged phosphorylated molecule, does not enter cells intact and is first converted outside cells to NR, so that oral NMN and oral NR end up doing the same thing biochemically. A 2019 mouse study reported that the gene Slc12a8 encodes an NMN transporter highly expressed in the small intestine (Grozio and colleagues, 2019); Schmidt and Brenner replied that the evidence did not show this (2019). A 2025 mouse study found that only a small portion of oral NMN and NR was directly absorbed; most was converted by gut bacteria to nicotinic acid, which then fed NAD+ synthesis, mainly in the liver (Yaku and colleagues, 2025).
- Methylation cofactor demand — when NAD+ is used by sirtuins, PARPs and CD38, nicotinamide is released, and much of it is methylated by the enzyme NNMT before excretion. Some writers argue that high-dose NMN or NR could therefore draw down the body's methyl-donor pool, and propose a methyl donor such as TMG (trimethylglycine). This is a theoretical concern; it has not been measured in the NMN trials found for this page. In a 4-week trial of NR at 3,000 mg a day in 20 people with Parkinson's disease, serum homocysteine rose slightly at first while the methyl-donor pool stayed intact (Berven and colleagues, 2023).
- Trial evidence — more human trials have used NR than NMN, because NR has been studied clinically for longer.
- Commercial ties — researchers on both sides have commercial ties disclosed in their papers: Brenner has advised a company that sells NR, and Sinclair co-founded a company developing a pharmaceutical-grade NMN drug candidate.
On the central biochemical question, a 2026 randomized, open-label, placebo-controlled study in 65 healthy adults compared the three precursors directly: 14 days of NR or NMN comparably increased circulating NAD+, while nicotinamide did not, and laboratory work in the same paper pointed to gut-microbial conversion to nicotinic acid as the route (Christen and colleagues, 2026). Most of that paper's authors are employees of a food and nutrition company. Both NR and NMN raise blood NAD+ in people; which, if either, produces lasting clinical benefit has not been shown.
What Is and Is Not Proven in Humans
An account of the human evidence through October 2026, from the trials described on the NAD+ & NMN main page:
Consistently found
- NMN and NR raise NAD+ or its metabolites in blood (and, in one study, muscle) in every trial that measured it; in a dose-ranging trial in 80 healthy middle-aged adults, blood NAD+ was highest at 600 and 900 mg of NMN (Yi and colleagues, 2023, whose authors include employees of chemical-manufacturing companies).
- In short trials both are well tolerated: a 2026 meta-analysis of randomized NMN trials (250 to 2,000 mg a day for 14 days to 24 weeks) found no increase in overall, serious or withdrawal-related adverse events (Yang and colleagues, 2026), and NR at 2,000 mg a day for 12 weeks caused no serious adverse events in obese men (Dollerup and colleagues, 2018).
Single or exploratory positive findings
- NMN 250 mg a day for 10 weeks increased muscle insulin sensitivity in 25 postmenopausal women with prediabetes (Yoshino Science 2021).
- Six-minute walking distance increased more with NMN than placebo in the 80-adult dose-ranging trial (Yi and colleagues, 2023).
- In runners training 5 to 6 times a week, several aerobic measures rose more with NMN at 600 and 1,200 mg than with placebo; VO2max itself did not change (Liao and colleagues, 2021).
- NR tended to lower blood pressure in 24 healthy middle-aged and older adults, but blood pressure was an exploratory outcome and the differences were not statistically significant after correction for multiple comparisons (Martens and colleagues, 2018).
Tested and not found
- Cognition did not change with NMN 250 mg a day in older men — 42 men randomized, 20 analysed at 12 weeks; gait speed and left-hand grip improved only nominally; the trial was funded by an NMN manufacturer (Igarashi and colleagues, 2022).
- Muscle mitochondrial bioenergetics did not change with NR in 12 older men (Elhassan and colleagues, 2019).
- Insulin sensitivity did not improve with NR at 2,000 mg a day in 40 obese men (Dollerup and colleagues, 2018).
- In a 2026 crossover trial in 11 young men, NMN at 1,200 mg a day abolished the exercise-induced rise in muscle mitochondrial content (Yang and colleagues, 2026).
Not studied in humans
- Lifespan — no study has measured lifespan in people taking NMN or NR. In mice the results are mixed: NR increased lifespan when started late in life in one study (Zhang and colleagues, 2016) but not in the multi-site Interventions Testing Program (Harrison and colleagues, 2021); nicotinamide improved healthspan but not lifespan (Mitchell and colleagues, 2018); and the only NMN lifespan data are a not-yet-peer-reviewed preprint reporting an 8.5% increase in median lifespan in female mice but not males (Kane and colleagues, preprint).
- Reversal of established cognitive decline, frailty or sarcopenia.
- Fertility in older women (the mouse data are striking; no human trials have been published).
- Slowing of biological-age clocks at the population level.
In summary, NMN and NR do what they are expected to do biochemically — raise NAD+ — and have been well tolerated in short trials. Whether this produces a clinically meaningful longevity benefit in humans has not been shown, and no human trial has shown a slowing of aging itself. Many of the trials were funded by, supplied by, or partly staffed by companies that make these compounds.
Combinations Discussed for Sirtuin Activation
Longevity writers and practitioners often discuss combining NMN or NR with other compounds on mechanistic grounds. None of these combinations has been tested for clinical benefit in a published human trial found for this page. The compounds most often discussed, and what the research reports:
- NMN or NR — trials have used NMN at 250 to 2,000 mg a day and NR mostly at 1,000 to 2,000 mg a day; these are the doses tested, not established effective doses. Popular advice to take NMN in the morning on an empty stomach has not been supported by trials: the one trial that compared morning and afternoon intake found the largest effect sizes for sit-to-stand time and drowsiness in the afternoon NMN group (Kim and colleagues, 2022).
- TMG (trimethylglycine) — proposed as a methyl donor to offset the methylation cost of NMN/NR metabolism; the depletion it is meant to offset has not been measured in NMN trials.
- Resveratrol — proposed to speed sirtuins while NMN supplies their NAD+; resveratrol activated SIRT1 only with an artificial test substrate in one study (Pacholec and colleagues, 2010) and did not extend mouse lifespan in the Interventions Testing Program (Miller and colleagues, 2011).
- Quercetin — identified with the cancer drug dasatinib as a senolytic that reduced senescent-cell burden in mice (Zhu and colleagues, 2015); the idea that it would lower CD38-driven NAD+ consumption has not been tested.
- Fisetin — another flavonoid studied as a senolytic in animals.
- Apigenin — a flavonoid that inhibited CD38 and raised NAD+ in cells and obese mice (Escande and colleagues, 2013); not tested with NMN in people.
Exercise has its own NAD+ data: in a cross-sectional study, muscle NAD+ in exercise-trained older people was closer to young levels than in sedentary older people (Janssens and colleagues, 2022). For the wider picture of how these interventions are combined, see Longevity Protocols.
Safety Findings and Open Questions
- The cancer question — because cancer cells depend on NAD+, researchers have asked whether raising NAD+ could help existing tumors. In mice, NMN promoted progression of an oncogenic-Kras pancreatic cancer model (Nacarelli and colleagues, 2019), NR increased triple-negative breast cancer prevalence and brain metastasis (Maric and colleagues, 2023), and NMN and nicotinamide made pancreatic cancer cells more resistant to chemotherapy (Nakazzi and colleagues, 2026). Other studies point the other way: SIRT1 overexpression reduced spontaneous cancers in mice (Herranz and colleagues, 2010). There are no human data on NMN or NR and cancer risk. The research raises a concern mainly for people with an existing or past cancer, and for people receiving chemotherapy.
- Methylation cofactor demand — a theoretical concern for chronic high-dose NMN or NR; it has not been measured in the NMN trials found for this page (see the Brenner debate above).
- Long-term safety unknown — the longest NMN trials in the 2026 safety meta-analysis ran 24 weeks. Effects over years are not characterized.
- Product quality — supplement quality, including whether a product contains the amount of NMN on its label, is not checked by the FDA before sale.
- Pregnancy and breastfeeding — the safety of NMN and NR in pregnancy and breastfeeding has not been studied.
- Glucose-lowering medicines — NMN increased muscle insulin sensitivity in one trial in women with prediabetes (Yoshino 2021); its effect in people taking insulin or sulfonylureas has not been studied in the trials found for this page (see Energy & Mitochondria). Decisions about supplements, especially for people with medical conditions or taking prescription medicines, belong with a clinician.
Key Research Papers
- Imai, S., Guarente, L. (2014). NAD+ and Sirtuins in Aging and Disease. Trends in Cell Biology 24(8), 464–471. — doi:10.1016/j.tcb.2014.04.002
- Bonkowski, M.S., Sinclair, D.A. (2016). Slowing Ageing by Design: The Rise of NAD+ and Sirtuin-Activating Compounds. Nature Reviews Molecular Cell Biology 17(11), 679–690. — doi:10.1038/nrm.2016.93
- Mills, K.F., et al. (2016). Long-Term Administration of Nicotinamide Mononucleotide Mitigates Age-Associated Physiological Decline in Mice. Cell Metabolism 24(6), 795–806. — doi:10.1016/j.cmet.2016.09.013
- Camacho-Pereira, J., et al. (2016). CD38 Dictates Age-Related NAD Decline and Mitochondrial Dysfunction Through a SIRT3-Dependent Mechanism. Cell Metabolism 23(6), 1127–1139. — doi:10.1016/j.cmet.2016.05.006
- Kanfi, Y., et al. (2012). The Sirtuin SIRT6 Regulates Lifespan in Male Mice. Nature 483(7388), 218–221. — PubMed PMID: 22367546
- Yoshino, J., Baur, J.A., Imai, S. (2018). NAD+ Intermediates: The Biology and Therapeutic Potential of NMN and NR. Cell Metabolism 27(3), 513–528. — doi:10.1016/j.cmet.2017.11.002
- Covarrubias, A.J., et al. (2021). NAD+ Metabolism and Its Roles in Cellular Processes During Ageing. Nature Reviews Molecular Cell Biology 22(2), 119–141. — doi:10.1038/s41580-020-00313-x
- Verdin, E. (2015). NAD+ in Aging, Metabolism, and Neurodegeneration. Science 350(6265), 1208–1213. — doi:10.1126/science.aac4854
- Yoshino, M., et al. (2021). Nicotinamide Mononucleotide Increases Muscle Insulin Sensitivity in Prediabetic Women. Science 372(6547), 1224–1229. — doi:10.1126/science.abe9985
- Martens, C.R., et al. (2018). Chronic Nicotinamide Riboside Supplementation Is Well-Tolerated and Elevates NAD+ in Healthy Middle-Aged and Older Adults. Nature Communications 9(1), 1286. — doi:10.1038/s41467-018-03421-7
- Gomes, A.P., et al. (2013). Declining NAD+ Induces a Pseudohypoxic State Disrupting Nuclear-Mitochondrial Communication During Aging. Cell 155(7), 1624–1638. — PubMed PMID: 24360282
- Khatri, S., Abdellatif, M., Sedej, S. (2025). Clinical Evidence for the Use of NAD+ Precursors to Slow Aging. Geromedicine 2025, 0008. (Not indexed in PubMed; the earlier version of this entry named the wrong authors.) — doi:10.70401/geromedicine.2025.0008
- Sinclair, D.A., Guarente, L. (1997). Extrachromosomal rDNA Circles — A Cause of Aging in Yeast. Cell 91(7), 1033–1042. — PubMed PMID: 9428525
- Howitz, K.T., et al. (2003). Small Molecule Activators of Sirtuins Extend Saccharomyces cerevisiae Lifespan. Nature 425, 191–196. — PubMed PMID: 12939617
- Bieganowski, P., Brenner, C. (2004). Discoveries of Nicotinamide Riboside as a Nutrient and Conserved NRK Genes Establish a Preiss-Handler Independent Route to NAD+ in Fungi and Humans. Cell 117(4), 495–502. — PubMed PMID: 15137942
- Massudi, H., et al. (2012). Age-Associated Changes in Oxidative Stress and NAD+ Metabolism in Human Tissue. PLoS One 7, e42357. — PubMed PMID: 22848760
- Zhu, X.H., et al. (2015). In Vivo NAD Assay Reveals the Intracellular NAD Contents and Redox State in Healthy Human Brain and Their Age Dependences. PNAS 112, 2876–2881. — PubMed PMID: 25730862
- Camacho-Pereira, J., et al. (2023). The NADase CD38 May Not Dictate NAD Levels in Brain Mitochondria of Aged Mice but Regulates Hydrogen Peroxide Generation. Free Radical Biology & Medicine 209, 29–39. — PubMed PMID: 37774804
- Mostoslavsky, R., et al. (2006). Genomic Instability and Aging-Like Phenotype in the Absence of Mammalian SIRT6. Cell 124(2), 315–329. — PubMed PMID: 16439206
- Pearson, K.J., et al. (2008). Resveratrol Delays Age-Related Deterioration and Mimics Transcriptional Aspects of Dietary Restriction Without Extending Life Span. Cell Metabolism 8, 157–168. — PubMed PMID: 18599363
- Pacholec, M., et al. (2010). SRT1720, SRT2183, SRT1460, and Resveratrol Are Not Direct Activators of SIRT1. Journal of Biological Chemistry 285, 8340–8351. — PubMed PMID: 20061378
- Herranz, D., et al. (2010). Sirt1 Improves Healthy Ageing and Protects From Metabolic Syndrome-Associated Cancer. Nature Communications 1, 3. — PubMed PMID: 20975665
- Miller, R.A., et al. (2011). Rapamycin, but Not Resveratrol or Simvastatin, Extends Life Span of Genetically Heterogeneous Mice. Journals of Gerontology: Series A 66, 191–201. — PubMed PMID: 20974732
- Hubbard, B.P., et al. (2013). Evidence for a Common Mechanism of SIRT1 Regulation by Allosteric Activators. Science 339, 1216–1219. — PubMed PMID: 23471411
- Satoh, A., et al. (2013). Sirt1 Extends Life Span and Delays Aging in Mice Through the Regulation of Nk2 Homeobox 1 in the DMH and LH. Cell Metabolism 18, 416–430. — PubMed PMID: 24011076
- Escande, C., et al. (2013). Flavonoid Apigenin Is an Inhibitor of the NAD+ase CD38. Diabetes 62(4), 1084–1093. — PubMed PMID: 23172919
- Mercken, E.M., et al. (2014). SRT2104 Extends Survival of Male Mice on a Standard Diet and Preserves Bone and Muscle Mass. Aging Cell 13, 787–796. — PubMed PMID: 24931715
- Zhu, Y., et al. (2015). The Achilles' Heel of Senescent Cells: From Transcriptome to Senolytic Drugs. Aging Cell 14, 644–658. — PubMed PMID: 25754370
- Zhang, H., et al. (2016). NAD+ Repletion Improves Mitochondrial and Stem Cell Function and Enhances Life Span in Mice. Science 352, 1436–1443. — PubMed PMID: 27127236
- Mitchell, S.J., et al. (2018). Nicotinamide Improves Aspects of Healthspan, but Not Lifespan, in Mice. Cell Metabolism 27, 667–676. — PubMed PMID: 29514072
- Dollerup, O.L., et al. (2018). A Randomized Placebo-Controlled Clinical Trial of Nicotinamide Riboside in Obese Men: Safety, Insulin-Sensitivity, and Lipid-Mobilizing Effects. American Journal of Clinical Nutrition 108, 343–353. — PubMed PMID: 29992272
- Elhassan, Y.S., et al. (2019). Nicotinamide Riboside Augments the Aged Human Skeletal Muscle NAD+ Metabolome and Induces Transcriptomic and Anti-inflammatory Signatures. Cell Reports 28, 1717–1728. — PubMed PMID: 31412242
- Grozio, A., et al. (2019). Slc12a8 Is a Nicotinamide Mononucleotide Transporter. Nature Metabolism 1, 47–57. — PubMed PMID: 31131364
- Schmidt, M.S., Brenner, C. (2019). Absence of Evidence That Slc12a8 Encodes a Nicotinamide Mononucleotide Transporter. Nature Metabolism 1, 660–661. — PubMed PMID: 32694648
- Nacarelli, T., et al. (2019). NAD+ Metabolism Governs the Proinflammatory Senescence-Associated Secretome. Nature Cell Biology 21, 397–407. — PubMed PMID: 30778219
- Harrison, D.E., et al. (2021). 17-a-Estradiol Late in Life Extends Lifespan in Aging UM-HET3 Male Mice; Nicotinamide Riboside and Three Other Drugs Do Not Affect Lifespan in Either Sex. Aging Cell 20, e13328. — PubMed PMID: 33788371
- McReynolds, M.R., et al. (2021). NAD+ Flux Is Maintained in Aged Mice Despite Lower Tissue Concentrations. Cell Systems 12, 1160–1172. — PubMed PMID: 34559996
- Roichman, A., et al. (2021). Restoration of Energy Homeostasis by SIRT6 Extends Healthy Lifespan. Nature Communications 12, 3208. — PubMed PMID: 34050173
- Igarashi, M., et al. (2022). Chronic Nicotinamide Mononucleotide Supplementation Elevates Blood Nicotinamide Adenine Dinucleotide Levels and Alters Muscle Function in Healthy Older Men. npj Aging 8, 5. — PubMed PMID: 35927255
- Kim, M., et al. (2022). Effect of 12-Week Intake of Nicotinamide Mononucleotide on Sleep Quality, Fatigue, and Physical Performance in Older Japanese Adults. Nutrients 14(4), 755. — PubMed PMID: 35215405
- Janssens, G.E., et al. (2022). Healthy Aging and Muscle Function Are Positively Associated With NAD+ Abundance in Humans. Nature Aging 2, 254–263. — PubMed PMID: 37118369
- Yi, L., et al. (2023). The Efficacy and Safety of β-Nicotinamide Mononucleotide (NMN) Supplementation in Healthy Middle-Aged Adults. GeroScience 45(1), 29–43. — PubMed PMID: 36482258
- Liao, B., et al. (2021). Nicotinamide Mononucleotide Supplementation Enhances Aerobic Capacity in Amateur Runners: A Randomized, Double-Blind Study. Journal of the International Society of Sports Nutrition 18(1), 54. — PubMed PMID: 34238308
- Maric, T., et al. (2023). A Bioluminescent-Based Probe for In Vivo Non-Invasive Monitoring of Nicotinamide Riboside Uptake Reveals a Link Between Metastasis and NAD+ Metabolism. Biosensors & Bioelectronics 220, 114826. — PubMed PMID: 36371959
- Yang, J.H., et al. (2023). Loss of Epigenetic Information as a Cause of Mammalian Aging. Cell 186, 305–326. — PubMed PMID: 36638792
- Berven, H., et al. (2023). NR-SAFE: A Randomized, Double-Blind Safety Trial of High Dose Nicotinamide Riboside in Parkinson's Disease. Nature Communications 14, 7793. — PubMed PMID: 38016950
- Yaku, K., et al. (2025). Nicotinamide Riboside and Nicotinamide Mononucleotide Facilitate NAD+ Synthesis via Enterohepatic Circulation. Science Advances 11, eadr1538. — PubMed PMID: 40117359
- Christen, S., et al. (2026). The Differential Impact of Three Different NAD+ Boosters on Circulatory NAD and Microbial Metabolism in Humans. Nature Metabolism 8, 62–73. — PubMed PMID: 41540253
- Trętowicz, M.M., et al. (2026). Human Whole-Blood NAD+ Levels Do Not Vary With Age or Lifestyle Interventions. Nature Metabolism 8, 1282–1290. — PubMed PMID: 42135539
- Yang, D.L., et al. (2026). Anti-Inflammatory Effects of Nicotinamide Mononucleotide (NMN) in Human Skeletal Muscle After BFR-Exercise. Journal of the International Society of Sports Nutrition 23, 2632284. — PubMed PMID: 41705654
- Yang, W., et al. (2026). Safety and Metabolism-Related Outcomes of Oral Nicotinamide Mononucleotide Supplementation in Adults: A Systematic Review and Meta-Analysis. Nutrients 18(14), 2251. — PubMed PMID: 42514320
- Nakazzi, F., et al. (2026). Vitamin B3 Derivatives Support Pancreatic Cancer Cell Survival and Chemotherapy Resistance. Cancer Letters 645, 218334. — PubMed PMID: 41724424
- Kane, A.E., et al. (2026). Long-Term NMN Treatment Increases Lifespan and Healthspan in Mice in a Sex Dependent Manner. Preprint, Research Square (earlier version posted to bioRxiv 2024); not peer-reviewed. — doi:10.21203/rs.3.rs-10913337/v1
PubMed Topic Searches
Connections
- NAD+ & NMN Overview
- NAD+ Benefits Hub
- NAD+ for Cognition
- NAD+ for Energy & Mitochondria
- NAD Precursors Compared
- Longevity Protocols
- Fasting
- Rapamycin
- Vitamin B3 (Niacin)
- Quercetin (Senolytic)
- Fisetin (Senolytic)
- All Antioxidants
- Methylene Blue
- Alpha Lipoic Acid
- Oxidative Stress
- Cancer (theoretical concern)
- History