NAD+ & NMN for Energy and Mitochondrial Function
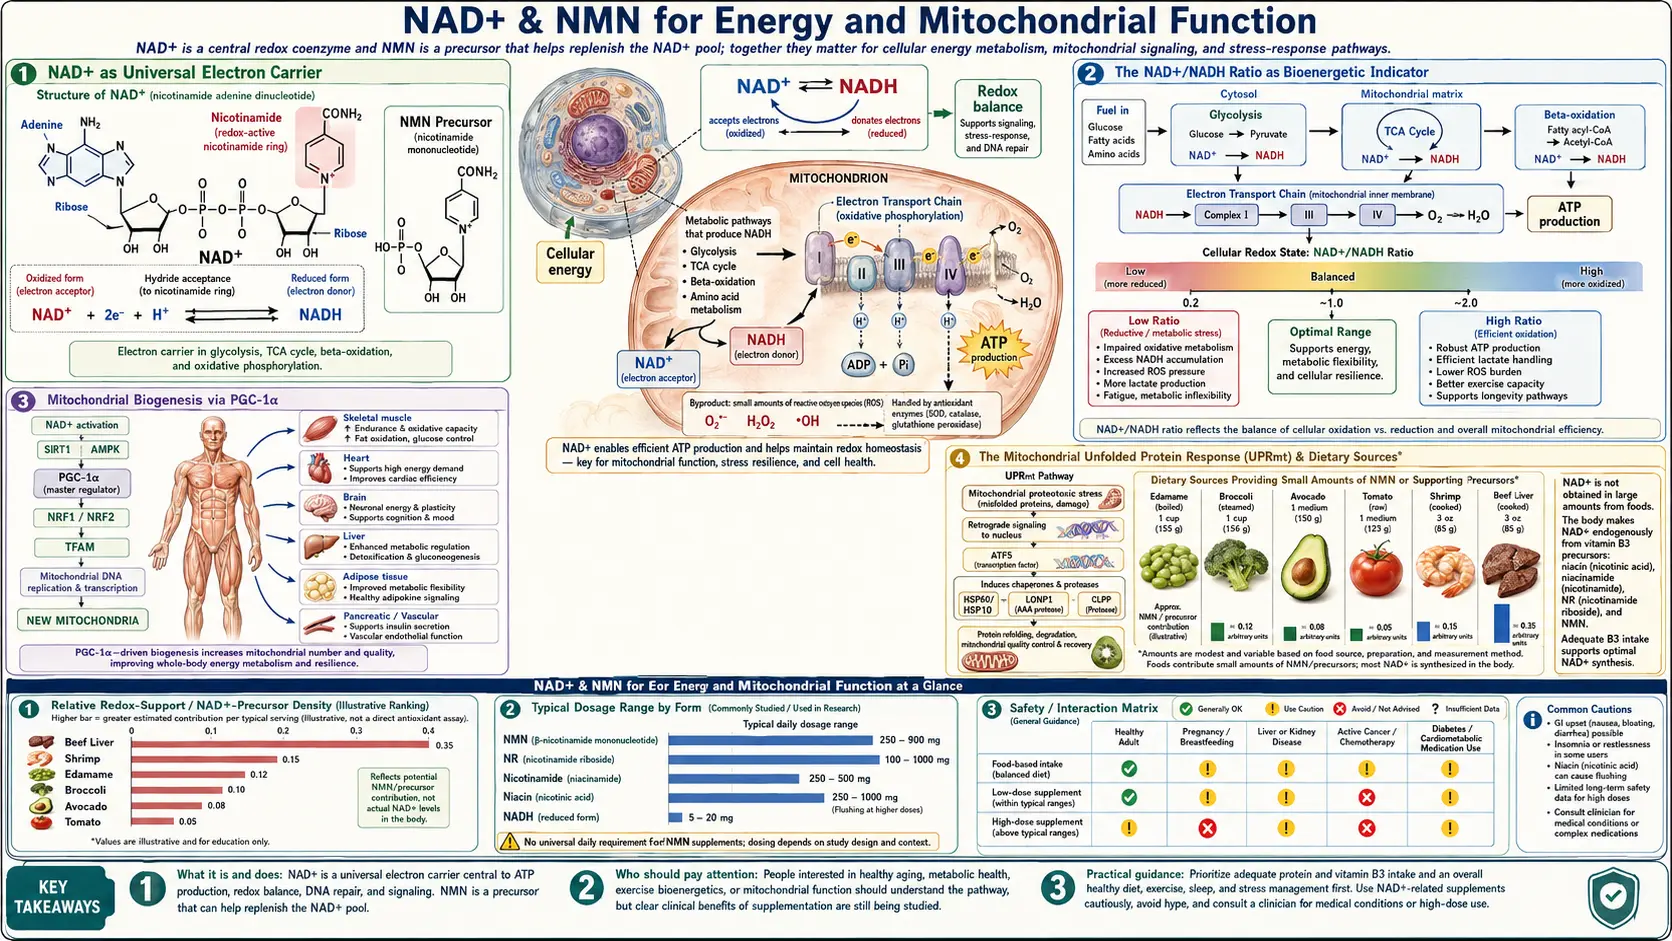
NAD+ is the universal electron carrier without which the mitochondrial electron transport chain cannot operate. When NAD+ falls, ATP production falls with it, reactive oxygen species leak from the chain, and cells lose the energy they need for repair, signaling, and resilience. These findings come mainly from cell and animal studies, and they are why NAD+ repletion is studied in fatigue states — chronic fatigue syndrome, long-COVID, post-viral fatigue, mitochondrial myopathies, age-related sarcopenia, and the everyday fatigue of midlife. In people, the muscle data so far do not show a mitochondrial effect. This deep-dive walks through NAD+ as electron carrier, the NAD+/NADH ratio as a bioenergetic readout, the mitochondrial unfolded protein response, AMPK and sirtuin cross-talk, the published exercise-capacity trials, what is known about IV NAD+ infusions, and the doses used in trials.
Table of Contents
- NAD+ as Universal Electron Carrier
- The NAD+/NADH Ratio as Bioenergetic Indicator
- Mitochondrial Biogenesis via PGC-1α
- The Mitochondrial Unfolded Protein Response (UPRmt)
- AMPK and Sirtuin Cross-Talk
- Exercise Capacity Trials
- Chronic Fatigue Syndrome and Mitochondrial Dysfunction
- Long COVID and Post-Viral Fatigue
- IV NAD+ Infusions
- Sarcopenia and Aging Muscle
- Cardiac Energetics
- Doses Used in Trials
- Safety Findings and Open Questions
- Key Research Papers
- Connections
- Featured Videos
NAD+ as Universal Electron Carrier
Cellular energy production reduces to a single chemical operation: capturing electrons from food molecules and using their movement down an energy gradient to drive ATP synthesis. NAD+ is the molecule that does the capturing. During glycolysis, the citric acid cycle, and fatty acid β-oxidation, NAD+ accepts electrons (and a proton) from carbon-bearing substrates to become NADH. The NADH then carries those electrons to Complex I of the mitochondrial electron transport chain, where they are passed down through Complexes I, III, and IV while pumping protons across the inner mitochondrial membrane. The proton gradient drives ATP synthase, and ATP is produced.
The arithmetic of the system explains why NAD+ is so central:
- Glycolysis (one glucose to two pyruvate) generates 2 NADH
- Pyruvate dehydrogenase (two pyruvate to two acetyl-CoA) generates 2 NADH
- Citric acid cycle (two acetyl-CoA fully oxidized) generates 6 NADH and 2 FADH2
- Each NADH that enters the electron transport chain at Complex I yields ~2.5 ATP
Without enough NAD+, glycolysis stalls (no acceptor for the GAPDH-generated electrons), pyruvate cannot be oxidized to acetyl-CoA, the citric acid cycle slows, and cellular ATP production collapses. The cell then resorts to anaerobic glycolysis (lactate production), which yields only 2 ATP per glucose instead of ~36, and acidifies the cytoplasm.
This is why NAD+ depletion is so consequential: it does not just dial down one pathway but disables the entire oxidative metabolic apparatus on which cells depend for sustained energy production.
The NAD+/NADH Ratio as Bioenergetic Indicator
The cell does not just care about the absolute amount of NAD+ — it cares about the ratio of NAD+ to NADH. This ratio is the bioenergetic readout that triggers downstream signaling. A high NAD+/NADH ratio (more oxidized form) signals fasting, exercise, caloric restriction, and metabolic stress; a low NAD+/NADH ratio (more reduced form) signals fed state, abundant fuel availability, and storage mode.
The NAD+/NADH ratio influences cellular function through:
- Sirtuin activity — sirtuins require NAD+ specifically (not NADH) as substrate. A high NAD+/NADH ratio means active sirtuins and the caloric-restriction-mimetic phenotype: autophagy, mitochondrial biogenesis, stress resistance, anti-inflammatory signaling.
- SIRT3 in mitochondria — the mitochondrial NAD+/NADH ratio drives SIRT3, which deacetylates and activates the antioxidant defenses and the fatty acid oxidation enzymes.
- Pyruvate-lactate balance — lactate dehydrogenase uses the cytoplasmic NAD+/NADH ratio to set the pyruvate-to-lactate equilibrium. Low NAD+/NADH (high NADH) drives pyruvate to lactate, contributing to lactic acidosis in mitochondrial dysfunction states.
- Gluconeogenesis — the liver's ability to make glucose from non-carbohydrate precursors during fasting depends on the cytoplasmic NAD+/NADH ratio.
NMN/NR supplementation raises the NAD+ pool in blood, and researchers propose that it raises the NAD+/NADH ratio in tissues as well. This is the biochemical basis for describing NMN as a fasting mimetic or exercise mimetic, a framing that human trials have not borne out so far (see the exercise section).
Mitochondrial Biogenesis via PGC-1α
Beyond serving as electron carrier, NAD+ regulates the number and quality of mitochondria in each cell through the PGC-1α (peroxisome proliferator-activated receptor gamma coactivator 1-alpha) pathway. PGC-1α is the master regulator of mitochondrial biogenesis — the cellular program for assembling new mitochondria from scratch.
The pathway works as follows:
- Caloric restriction, exercise, or other energy stress raises the cellular NAD+/NADH ratio.
- Elevated NAD+ activates SIRT1.
- Activated SIRT1 deacetylates PGC-1α, converting it from an inactive to an active state.
- Active PGC-1α drives transcription of nuclear-encoded mitochondrial genes (mitochondrial transcription factor A, respiratory chain subunits, fatty acid oxidation enzymes).
- New mitochondria are assembled, increasing cellular oxidative capacity.
This is the molecular basis of one of the foundational principles of exercise physiology: aerobic training increases mitochondrial density in skeletal muscle, which then enables greater endurance capacity. Researchers propose that NAD+ availability limits the SIRT1 deacetylation step. In mice, 12 months of NMN enhanced mitochondrial oxidative metabolism in skeletal muscle (Mills and colleagues, 2016). In people the result has been different: in a 2026 crossover trial in 11 untrained young men, NMN at 1,200 mg a day for 7 days abolished the exercise-induced rise in muscle mitochondrial content (Yang and colleagues, 2026).
AMPK provides a parallel pathway: AMPK phosphorylates PGC-1α at sites that prime it for SIRT1-mediated deacetylation. NAD+ and AMPK therefore cooperate to drive mitochondrial biogenesis (see the AMPK section below).
The Mitochondrial Unfolded Protein Response (UPRmt)
Mitochondria have their own quality-control system that monitors the folding state of their proteins and triggers a stress response when too many are misfolded. This system, called the mitochondrial unfolded protein response (UPRmt), is the mitochondrial equivalent of the better-known endoplasmic reticulum UPR.
The UPRmt was first characterized in C. elegans, where mild activation of the response extends lifespan substantially. Subsequent work in mammals has shown that the UPRmt is regulated in part by NAD+/sirtuin signaling and that it activates a coordinated program including:
- Mitochondrial chaperone induction (mtHSP70, HSP60) to refold misfolded proteins
- Mitochondrial protease induction (LonP1, ClpXP) to degrade terminally misfolded proteins
- Mitochondrial biogenesis to replace damaged mitochondria with new ones
- Reduced cytoplasmic translation to lower the demand on mitochondrial protein import machinery
- Mitochondrial-derived peptide signaling (e.g., MOTS-c) to non-mitochondrial systems
Worm and mouse studies report that mitonuclear protein imbalance triggers the UPRmt and is associated with longer life in worms (Houtkooper and colleagues, 2013), and NAD+ precursors have been reported to activate the UPRmt in animal studies. The UPRmt is therefore one of the proposed mechanisms for NAD+ precursor effects in preclinical models. Mouse lifespan results with NAD+ precursors are mixed: NR extended lifespan in one study (Zhang and colleagues, 2016) but not in the multi-site Interventions Testing Program (Harrison and colleagues, 2021), and the only NMN lifespan data are a not-yet-peer-reviewed preprint (Kane and colleagues, preprint).
AMPK and Sirtuin Cross-Talk
AMPK (AMP-activated protein kinase) and the sirtuins are the cell's two principal energy-status sensors, and they cooperate extensively. AMPK is activated when the AMP/ATP ratio rises (signaling low energy); sirtuins are activated when the NAD+/NADH ratio rises (signaling oxidative metabolic stress).
The cross-talk runs in both directions:
- AMPK phosphorylates and activates NAMPT, increasing NAD+ salvage synthesis — raising NAD+ availability for sirtuins.
- AMPK phosphorylates PGC-1α, priming it for SIRT1-mediated deacetylation.
- Sirtuins deacetylate LKB1, the upstream activator of AMPK, increasing AMPK activity.
- SIRT1 deacetylates PGC-1α that has been phosphorylated by AMPK, fully activating it for transcriptional duty.
In this model, interventions that activate either pathway tend to amplify the other: caloric restriction, exercise, metformin (an AMPK activator), berberine (also AMPK), and NMN/NR (sirtuin substrate) are proposed to converge on the same downstream metabolic adaptation. Some integrative practitioners combine NMN with metformin or berberine on this rationale; the combinations have not been tested in published human trials found for this page.
Exercise activates the whole system: an aerobic exercise session raises AMPK, raises the NAD+/NADH ratio, activates sirtuins, and triggers PGC-1α-driven mitochondrial biogenesis. In a cross-sectional study, muscle NAD+ in exercise-trained older people was closer to young levels than in sedentary older people (Janssens and colleagues, 2022).
Exercise Capacity Trials
The largest human exercise trial of NMN is Liao and colleagues (2021), a 6-week randomized, double-blind, placebo-controlled trial in 48 young and middle-aged recreational runners (ten men and two women per group). Participants received placebo, 300 mg, 600 mg, or 1,200 mg NMN per day while training 5–6 times a week.
Results:
- Oxygen uptake, the percentage of VO2max at which participants worked, and power at the first and second ventilatory thresholds rose more in the 600 mg and 1,200 mg groups than with placebo
- The 300 mg group did not differ from placebo on these measures
- VO2max itself, O2-pulse, and peak power did not change in any group
- The authors reported no conflicts of interest; the trial was funded by a national government research program
The authors attributed the pattern to better oxygen use by skeletal muscle during submaximal exercise rather than greater peak capacity.
Other exercise and physical-function results are mixed:
- In a 2026 crossover trial in 11 untrained young men, NMN at 1,200 mg a day for 7 days blunted inflammatory signaling in muscle after blood-flow-restricted exercise, but abolished the exercise-induced rise in muscle mitochondrial content and moderately delayed the clearing of damaged tissue (Yang and colleagues, 2026).
- In a dose-ranging trial in 80 healthy middle-aged adults, six-minute walking distance increased more in all NMN groups than with placebo (Yi and colleagues, 2023; three authors are employees of chemical-manufacturing companies).
- In 108 older Japanese adults, sit-to-stand times improved in all four groups, including placebo; the afternoon NMN group showed the largest effect size (Kim and colleagues, 2022).
- A 2025 meta-analysis of NMN and NR trials in adults with a mean age over 60 found no significant effect of NMN on muscle mass, grip strength, gait speed or chair-stand time (Prokopidis and colleagues, 2025).
Taken together, the exercise evidence consists of a few small trials with mixed findings; none tested competitive performance.
Chronic Fatigue Syndrome and Mitochondrial Dysfunction
Myalgic encephalomyelitis/chronic fatigue syndrome (ME/CFS) is the prototypical chronic fatigue disorder — a complex, multisystem illness characterized by post-exertional malaise, unrefreshing sleep, cognitive dysfunction, and severe functional impairment lasting more than six months. A consistent biological finding in ME/CFS is impaired mitochondrial function: reduced ATP production from peripheral blood mononuclear cells, increased lactate production with mild exertion, and abnormal cellular bioenergetic profiles on Seahorse XF analysis.
The mitochondrial dysfunction in ME/CFS has multiple proposed contributors:
- Oxidative damage to mitochondrial DNA and respiratory chain proteins from chronic inflammation
- Reduced NAD+ availability from chronic immune activation (CD38 upregulation, PARP activation from chronic DNA damage)
- Abnormal pyruvate dehydrogenase activity reducing acetyl-CoA generation
- Impaired fatty acid oxidation
- Reactivation of latent herpesviruses (EBV, HHV-6) producing chronic immune activation
The proposed rationale for NAD+ precursors in ME/CFS is to replenish the NAD+ pool, support the impaired bioenergetic machinery, and reduce the chronic inflammation proposed to drive ongoing NAD+ depletion. Clinical evidence is anecdotal and preliminary — no large RCT has tested NMN or NR specifically in ME/CFS — although some integrative practitioners include NMN/NR, often with CoQ10, D-ribose, magnesium, and L-carnitine, in ME/CFS protocols; those combinations have not been tested in published trials found for this page. See our Chronic Fatigue Syndrome page for the broader clinical picture.
Long COVID and Post-Viral Fatigue
The post-acute sequelae of viral infection — including the syndrome popularly known as long COVID and the broader category of post-viral fatigue syndromes following EBV, mononucleosis, Ross River virus, and others — share substantial overlap with ME/CFS in symptoms and proposed mechanism. Mitochondrial dysfunction, persistent low-grade immune activation, and reduced NAD+ availability have been proposed as common features across the post-viral fatigue spectrum.
Some integrative-medicine practitioners have used NMN, NR, and IV NAD+ infusions for post-viral fatigue. The proposed rationale draws on:
- Reports of NAD+ depletion in COVID-19, proposed to be driven by PARP activation and by CD38 upregulation from immune activation
- Reports of mitochondrial dysfunction in long-COVID patients, including reduced oxidative capacity and increased lactate production
- The hypothesis that restoring NAD+ would support recovery of mitochondrial function
Controlled clinical trial evidence remains limited, and anecdotal reports are not equivalent to controlled data. The approaches with a longer record in post-viral fatigue management are activity pacing, attention to sleep, gradual rather than sudden return to exercise, and addressing comorbid conditions like POTS and MCAS.
IV NAD+ Infusions
Intravenous NAD+ is offered in longevity clinics, addiction treatment centers, and IV nutrient therapy practices, often as part of a multi-day course. Session lengths, doses and schedules are set by the clinics; they come from clinic practice, not from trials. Proponents say bypassing the gut gives higher blood levels than oral supplements.
What the published data show
- A 2019 pilot study in 11 healthy men aged 30 to 55 gave 8 of them 750 mg of NAD+ by infusion over 6 hours and 3 a saline infusion (Grant and colleagues, 2019). Plasma NAD+ and its metabolites did not change for the first 2 hours, indicating that the infused NAD+ was rapidly and completely removed from the plasma; the metabolite pattern pointed to breakdown by NAD+-degrading enzymes, and NAD+ itself and methylnicotinamide appeared in urine.
- No adverse events were observed during those infusions. The study measured blood and urine chemistry, not clinical outcomes.
- NAD+ is a large, charged molecule that does not readily cross cell membranes, and how much infused NAD+ reaches the inside of cells is unknown; it may be broken down outside cells to NMN or nicotinamide first.
- IV NAD+ is not an FDA-approved treatment for any condition. Side-effect rates in routine clinic use have not been reported in controlled studies found for this page.
Claims made for IV NAD+
- Clinics and users report improved energy, mental clarity, and reduced cravings, particularly in addiction-recovery settings; these reports are subjective and uncontrolled
- Clinics also offer it for chronic fatigue, post-viral fatigue, and people who do not tolerate oral supplements
- No controlled trial found for this page has compared IV NAD+ with oral NMN or NR, or tested any of these clinical claims
Sarcopenia and Aging Muscle
Sarcopenia — the progressive loss of skeletal muscle mass, strength, and function with aging — is one of the most consequential aging-related changes, contributing to falls, fractures, disability, and mortality. Mitochondrial dysfunction is central to sarcopenia: aged skeletal muscle shows reduced mitochondrial density, impaired oxidative phosphorylation, and decreased oxidative capacity.
NAD+ repletion has been tested in aging-muscle contexts:
- Mouse studies: raising NAD+ with NMN restored mitochondrial function in aged mouse skeletal muscle within one week (Gomes et al., Cell 2013), and 12 months of NMN enhanced mitochondrial oxidative metabolism in muscle (Mills and colleagues, 2016)
- Human exercise trials: NMN improved several submaximal aerobic measures in young and middle-aged recreational runners (Liao 2021), but abolished the exercise-induced rise in muscle mitochondrial content in a 2026 trial in young men (Yang 2026)
- The Igarashi 2022 NMN trial in older men (42 randomized, 20 analysed at 12 weeks; funded by an NMN manufacturer) found only nominally significant improvements in gait speed and left-hand grip, and no change in body composition
- NR at 1 g a day for 21 days did not change muscle mitochondrial bioenergetics in 12 older men (Elhassan 2019)
- A 2025 meta-analysis found no significant effect of NMN on muscle mass, grip strength, gait speed or chair-stand time in adults with a mean age over 60, and concluded that current evidence does not support NMN or NR for preserving muscle mass and function in that age group (Prokopidis 2025)
- Yoshino 2021 showed improved skeletal muscle insulin signaling in 25 postmenopausal women with prediabetes
In sarcopenia research, resistance exercise and adequate protein intake (1.2–1.6 g/kg/day is a range often cited for older adults) have the strongest evidence. No trial found for this page has shown that adding an NAD+ precursor to resistance training preserves muscle.
Cardiac Energetics
The heart beats approximately 100,000 times per day and requires sustained, reliable ATP production to do so. Heart failure, whether with reduced ejection fraction (HFrEF) or preserved ejection fraction (HFpEF), is increasingly understood as a disease of cardiac energetics: the failing heart cannot meet its ATP demand because of impaired mitochondrial function.
In animal studies, cardiac NAD+ levels decline with age and decline further in heart failure. SIRT3, the mitochondrial sirtuin, is particularly important in cardiac myocytes. Preclinical studies have shown that boosting NAD+ levels with NMN or NR improves cardiac function in mouse models of:
- Ischemic cardiomyopathy
- Diabetic cardiomyopathy
- Dilated cardiomyopathy
- Hypertrophic cardiomyopathy
- Arrhythmogenic cardiomyopathy
- Heart failure with preserved ejection fraction
Human data are limited and mostly exploratory. In the Martens 2018 NR trial (24 healthy middle-aged and older adults who completed a 6-week crossover), NR tended to lower systolic and diastolic blood pressure, but blood pressure was exploratory and the differences were not statistically significant after correction for multiple comparisons. In a 28-day trial in 30 overweight or obese adults aged 45 or older, body weight, diastolic blood pressure, and total and LDL cholesterol fell more with a pharmaceutical-grade NMN tablet than with placebo, while muscle strength, aerobic capacity, insulin sensitivity and liver fat did not differ; the trial was funded partly by the drug's developer and partly by NIH grants (Pencina and colleagues, 2023).
No trial has tested NMN or NR alongside standard cardiac care (statins, ACE inhibitors, beta-blockers, SGLT2 inhibitors, diet, exercise) in people with heart disease. The preclinical case is extensive (reviewed by Kane and Sinclair, 2018); the clinical-trial case is not yet established.
Doses Used in Trials
These are the doses tested in the trials on this page, not established effective doses; no dose of NMN or NR has been shown to produce a lasting clinical benefit.
NMN
- 250 mg/day for 6 to 12 weeks in older adults (Igarashi 2022; Kim 2022) and for 10 weeks in women with prediabetes (Yoshino 2021)
- 300 to 900 mg/day for 60 days in the dose-ranging trial in healthy middle-aged adults (Yi 2023)
- 300, 600 and 1,200 mg/day for 6 weeks in runners; aerobic measures improved at 600 and 1,200 mg but not 300 mg (Liao 2021)
- 1,200 mg/day for 7 days in the 2026 exercise trial that found a loss of the exercise mitochondrial gain (Yang 2026)
- Overall, 250 to 2,000 mg/day for 14 days to 24 weeks in the trials pooled by the 2026 safety meta-analysis
NR
- 1,000 mg/day in most trials (Martens 2018; Elhassan 2019); 2,000 mg/day for 12 weeks in obese men (Dollerup 2018)
Timing
- The one trial that compared morning and afternoon NMN found the largest effects with afternoon intake (Kim 2022). Claims that NMN works best in the morning, on an empty stomach, or 30–60 minutes before training have not been tested in trials found for this page.
Combinations discussed
- Practitioner protocols for chronic or post-viral fatigue often combine NMN or NR with CoQ10, D-ribose, L-carnitine or acetyl-L-carnitine, magnesium, and TMG, and some cardiac protocols pair NMN or NR with CoQ10; none of these combinations has been tested in a published trial found for this page.
- Comorbid conditions that drive ongoing fatigue (POTS, MCAS, SIBO, hypothyroidism, low iron) are addressed separately in clinical care.
Decisions about supplements, especially for people with medical conditions or taking prescription medicines, belong with a clinician.
Safety Findings and Open Questions
- Glucose-lowering medicines — NMN increased muscle insulin sensitivity in one trial in women with prediabetes (Yoshino 2021), and meta-analyses of NMN trials found no effect on fasting glucose. Its effect in people taking insulin or sulfonylureas has not been studied in the trials found for this page; the question of hypoglycemia in that group is open.
- Sleep and time of day — some users report that NMN taken late in the day disturbs sleep; in the one trial that compared morning and afternoon intake, the afternoon NMN group showed the largest reduction in drowsiness (Kim 2022).
- Methylation cofactor demand — a theoretical concern for chronic high-dose NMN/NR; it has not been measured in the NMN trials found for this page.
- IV NAD+ infusions — chest tightness, abdominal discomfort, flushing, and nausea are reported during infusions, particularly when they are run fast; side-effect rates in routine clinic use have not been reported in controlled studies.
- Heart failure — NMN and NR have not been tested alongside standard heart-failure medicines; decisions about adding a supplement belong with the treating cardiologist.
- The cancer question — mouse and cell studies report that NMN or NR promoted some cancers or chemotherapy resistance; see Longevity & Sirtuins for the discussion.
- Long-term safety unknown — the longest NMN trials in the 2026 safety meta-analysis ran 24 weeks; multi-year effects are uncharacterized.
Key Research Papers
- Liao, B., et al. (2021). Nicotinamide Mononucleotide Supplementation Enhances Aerobic Capacity in Amateur Runners: A Randomized, Double-Blind Study. Journal of the International Society of Sports Nutrition 18(1), 54. — doi:10.1186/s12970-021-00442-4
- Gomes, A.P., et al. (2013). Declining NAD+ Induces a Pseudohypoxic State Disrupting Nuclear-Mitochondrial Communication During Aging. Cell 155(7), 1624–1638. — PubMed PMID: 24360282
- Mills, K.F., et al. (2016). Long-Term Administration of Nicotinamide Mononucleotide Mitigates Age-Associated Physiological Decline in Mice. Cell Metabolism 24(6), 795–806. — doi:10.1016/j.cmet.2016.09.013
- Yoshino, M., et al. (2021). Nicotinamide Mononucleotide Increases Muscle Insulin Sensitivity in Prediabetic Women. Science 372(6547), 1224–1229. — doi:10.1126/science.abe9985
- Martens, C.R., et al. (2018). Chronic Nicotinamide Riboside Supplementation Is Well-Tolerated and Elevates NAD+ in Healthy Middle-Aged and Older Adults. Nature Communications 9(1), 1286. — doi:10.1038/s41467-018-03421-7
- Igarashi, M., et al. (2022). Chronic Nicotinamide Mononucleotide Supplementation Elevates Blood NAD Levels and Alters Muscle Function in Healthy Older Men. NPJ Aging 8, 5. — PubMed PMID: 35927255
- Camacho-Pereira, J., et al. (2016). CD38 Dictates Age-Related NAD Decline and Mitochondrial Dysfunction Through a SIRT3-Dependent Mechanism. Cell Metabolism 23(6), 1127–1139. — doi:10.1016/j.cmet.2016.05.006
- Houtkooper, R.H., et al. (2013). Mitonuclear Protein Imbalance as a Conserved Longevity Mechanism. Nature 497(7450), 451–457. — PubMed PMID: 23698443
- Canto, C., et al. (2009). AMPK Regulates Energy Expenditure by Modulating NAD+ Metabolism and SIRT1 Activity. Nature 458(7241), 1056–1060. — PubMed PMID: 19262508
- Tomás-Loba, A., et al. (2008). Telomerase Reverse Transcriptase Delays Aging in Cancer-Resistant Mice. Cell 135, 609–622. (Editorial note: this paper concerns telomerase, not sirtuins; the earlier annotation "context for sirtuin-telomere interaction" did not match it.) — PubMed PMID: 19013273
- Grant, R., et al. (2019). A Pilot Study Investigating Changes in the Human Plasma and Urine NAD+ Metabolome During a 6-Hour Intravenous Infusion of NAD+. Frontiers in Aging Neuroscience 11, 257. — PubMed PMID: 31572171
- Bonkowski, M.S., Sinclair, D.A. (2016). Slowing Ageing by Design: The Rise of NAD+ and Sirtuin-Activating Compounds. Nature Reviews Molecular Cell Biology 17(11), 679–690. — doi:10.1038/nrm.2016.93
- Zhang, H., et al. (2016). NAD+ Repletion Improves Mitochondrial and Stem Cell Function and Enhances Life Span in Mice. Science 352, 1436–1443. — PubMed PMID: 27127236
- Kane, A.E., Sinclair, D.A. (2018). Sirtuins and NAD+ in the Development and Treatment of Metabolic and Cardiovascular Diseases. Circulation Research 123(7), 868–885. — PubMed PMID: 30355082
- Dollerup, O.L., et al. (2018). A Randomized Placebo-Controlled Clinical Trial of Nicotinamide Riboside in Obese Men: Safety, Insulin-Sensitivity, and Lipid-Mobilizing Effects. American Journal of Clinical Nutrition 108, 343–353. — PubMed PMID: 29992272
- Elhassan, Y.S., et al. (2019). Nicotinamide Riboside Augments the Aged Human Skeletal Muscle NAD+ Metabolome and Induces Transcriptomic and Anti-inflammatory Signatures. Cell Reports 28, 1717–1728. — PubMed PMID: 31412242
- Harrison, D.E., et al. (2021). 17-a-Estradiol Late in Life Extends Lifespan in Aging UM-HET3 Male Mice; Nicotinamide Riboside and Three Other Drugs Do Not Affect Lifespan in Either Sex. Aging Cell 20, e13328. — PubMed PMID: 33788371
- Kim, M., et al. (2022). Effect of 12-Week Intake of Nicotinamide Mononucleotide on Sleep Quality, Fatigue, and Physical Performance in Older Japanese Adults. Nutrients 14(4), 755. — PubMed PMID: 35215405
- Janssens, G.E., et al. (2022). Healthy Aging and Muscle Function Are Positively Associated With NAD+ Abundance in Humans. Nature Aging 2, 254–263. — PubMed PMID: 37118369
- Yi, L., et al. (2023). The Efficacy and Safety of β-Nicotinamide Mononucleotide (NMN) Supplementation in Healthy Middle-Aged Adults. GeroScience 45(1), 29–43. — PubMed PMID: 36482258
- Pencina, K.M., et al. (2023). Nicotinamide Adenine Dinucleotide Augmentation in Overweight or Obese Middle-Aged and Older Adults: A Physiologic Study. Journal of Clinical Endocrinology & Metabolism 108, 1968–1980. — PubMed PMID: 36740954
- Prokopidis, K., et al. (2025). The Effect of Nicotinamide Mononucleotide and Riboside on Skeletal Muscle Mass and Function: A Systematic Review and Meta-Analysis. Journal of Cachexia, Sarcopenia and Muscle 16, e13799. — PubMed PMID: 40275690
- Yang, D.L., et al. (2026). Anti-Inflammatory Effects of Nicotinamide Mononucleotide (NMN) in Human Skeletal Muscle After BFR-Exercise. Journal of the International Society of Sports Nutrition 23, 2632284. — PubMed PMID: 41705654
- Yang, W., et al. (2026). Safety and Metabolism-Related Outcomes of Oral Nicotinamide Mononucleotide Supplementation in Adults: A Systematic Review and Meta-Analysis. Nutrients 18(14), 2251. — PubMed PMID: 42514320
- Kane, A.E., et al. (2026). Long-Term NMN Treatment Increases Lifespan and Healthspan in Mice in a Sex Dependent Manner. Preprint, Research Square (earlier version posted to bioRxiv 2024); not peer-reviewed. — doi:10.21203/rs.3.rs-10913337/v1
PubMed Topic Searches
Connections
- NAD+ & NMN Overview
- NAD+ Benefits Hub
- NAD+ for Longevity & Sirtuins
- NAD+ for Cognition
- NAD Precursors Compared
- CoQ10
- Alpha Lipoic Acid for Mitochondria
- All Antioxidants
- Chronic Fatigue Syndrome
- Cardiovascular Disease
- Insulin Resistance
- Longevity Protocols
- Berberine (AMPK)
- Fasting
- Creatine
- Vitamin B3 (Niacin)
- Magnesium
- History