⚠ Evidence warning: Clinical trials or other evidence do not support the claim that passionflower has a legitimate role in benzodiazepine tapering protocols, or the claim that its benzoflavone reverses morphine, nicotine and cannabinoid tolerance (animal studies from one research group only; an independent laboratory found the benzoflavone only in trace amounts, in one of three herb samples). This page keeps it as a report of what people, websites or other media say.
Passionflower Gamma-Aminobutyric Acid (GABA) Modulation
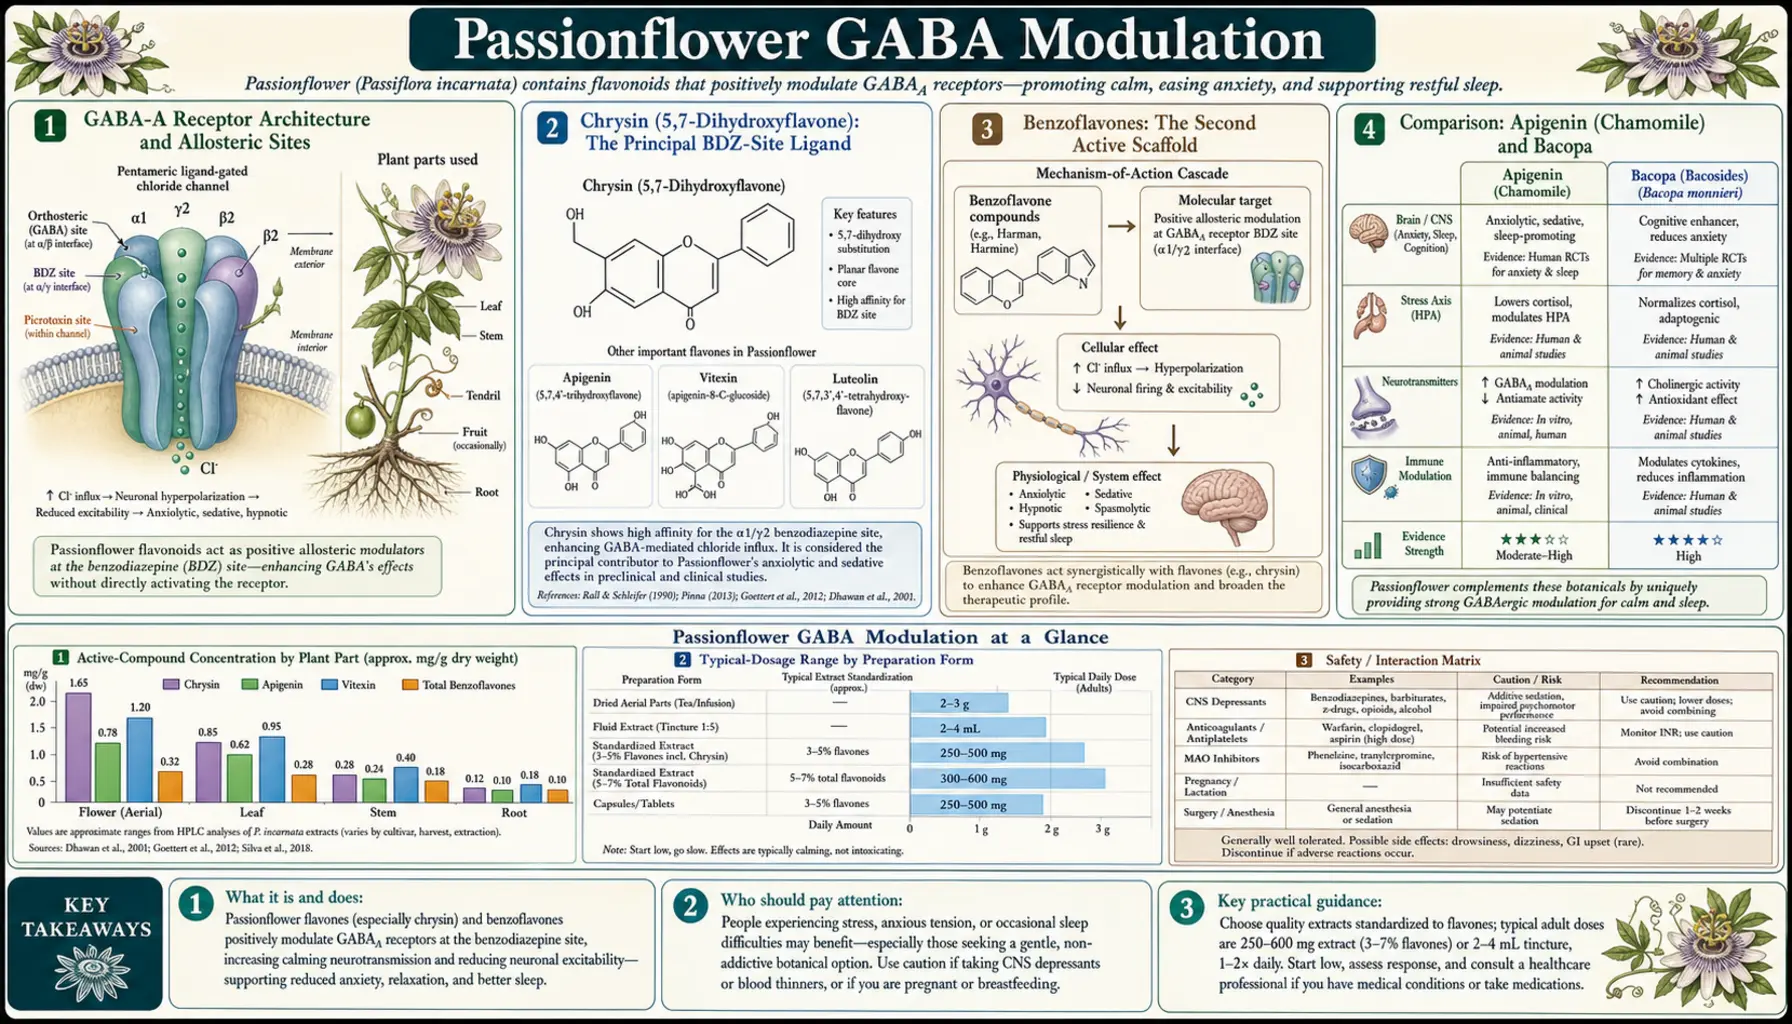
The pharmacology of passionflower centers on the gamma-aminobutyric acid-A receptor, the principal inhibitory ionotropic receptor of the mammalian central nervous system. Wolfman and Medina's 1994 work isolated chrysin (5,7-dihydroxyflavone) from Passiflora coerulea and demonstrated it bound the benzodiazepine site of the gamma-aminobutyric acid-A receptor — the same allosteric pocket where diazepam, lorazepam, alprazolam, and zolpidem exert their effects. Dhawan's 2001 work proposed a second active scaffold, a benzoflavone moiety, after finding an anxiolytic fraction of the extract in mice; an independent laboratory later found a compound matching it only in trace amounts, in one of three herb samples. The combined effect of chrysin, benzoflavones, and several other flavone aglycones is partial-agonist potentiation of gamma-aminobutyric acid-A current, producing modest amplification of endogenous GABAergic inhibition without the powerful clamping effect of full benzodiazepine agonists. Beyond gamma-aminobutyric acid (GABA), passionflower also contains trace beta-carboline alkaloids (harman, harmine, harmaline, harmol) that are weak reversible inhibitors of monoamine oxidase A — the basis for theoretical interaction concerns with selective serotonin reuptake inhibitors (SSRIs), monoamine oxidase inhibitors (MAOIs), and tyramine-containing foods. This deep-dive explores the receptor-level pharmacology, comparison with related botanical anxiolytics (apigenin/chamomile, bacopa, valerian), the harman alkaloid story, and what the multi-mechanism profile means for clinical use.
Table of Contents
- Gamma-Aminobutyric Acid-A Receptor Architecture and Allosteric Sites
- Chrysin (5,7-Dihydroxyflavone): The Principal BDZ-Site Ligand
- Benzoflavones: The Second Active Scaffold
- Comparison: Apigenin (Chamomile) and Bacopa
- Non-Benzodiazepine-Site Gamma-Aminobutyric Acid-A Modulation
- Harman Beta-Carboline Alkaloids and MAO-A
- Why Partial Agonism Produces Gentler Effects
- Tolerance, Dependence, and Withdrawal Profile
- Flumazenil Blocked Chrysin and the Whole Extract in Mice
- Theoretical and Real Drug Interaction Concerns
- GABA Itself Is in the Extract
- Key Research Papers
- Connections
- Featured Videos
Gamma-Aminobutyric Acid-A Receptor Architecture and Allosteric Sites
The gamma-aminobutyric acid-A receptor is a pentameric chloride-channel ligand-gated ion channel, the dominant fast-inhibitory neurotransmitter receptor in the mammalian central nervous system. Each receptor is built from five protein subunits drawn from a family of 19 known mammalian subunits (alpha1-6, beta1-3, gamma1-3, delta, epsilon, theta, pi, and rho1-3). The most common configuration in adult cortex is 2×alpha, 2×beta, and 1×gamma2, typically with the alpha1 subunit subtype, though other compositions (alpha2, alpha3, alpha5, delta-containing) predominate in specific brain regions and produce distinct pharmacology.
When gamma-aminobutyric acid binds the orthosteric site (located at the alpha-beta subunit interface), the chloride channel opens, chloride flows into the neuron, the neuron hyperpolarizes, and excitability decreases. This is the basic inhibitory function. Multiple allosteric sites on the receptor modulate this response, increasing or decreasing the chloride current produced by a given amount of orthosteric gamma-aminobutyric acid. The pharmacologically important allosteric sites include:
- Benzodiazepine binding site — located at the alpha-gamma subunit interface, requires gamma2 subunit. Positive modulators (diazepam, lorazepam, alprazolam, chrysin, apigenin) potentiate gamma-aminobutyric acid current; negative modulators (beta-carbolines like DMCM) reduce it; antagonists (flumazenil) block other ligands without intrinsic activity
- Barbiturate site — pentobarbital, phenobarbital, propofol. At high doses, can directly open the channel without gamma-aminobutyric acid, which is why barbiturate overdose is lethal in a way benzodiazepine overdose typically is not
- Neurosteroid site — allopregnanolone, THDOC, brexanolone (U.S. Food and Drug Administration-approved for postpartum depression). Powerful positive modulators
- Anesthetic site — volatile anesthetics, etomidate, etc.
- Alcohol site(s) — ethanol modulates multiple gamma-aminobutyric acid-A subtypes through poorly defined sites
Passionflower's primary action is at the benzodiazepine site through chrysin and related flavones, with additional activity at non-benzodiazepine-site allosteric pockets through other flavone aglycones (discussed below). This multi-site profile is what distinguishes botanical gamma-aminobutyric acid modulation from single-target pharmaceutical benzodiazepines.
Chrysin (5,7-Dihydroxyflavone): The Principal BDZ-Site Ligand
Chrysin is a flavone (a subclass of flavonoid) with the structural formula 5,7-dihydroxyflavone — a relatively simple flavone with two hydroxyl groups on the A-ring and no substitution on the B-ring. It is widely distributed in plants and is found in honey, propolis, passionflower, and other botanical sources. Medina and colleagues first demonstrated in 1990 that chrysin bound the central benzodiazepine receptor with measurable (though modest) affinity in rat brain membrane assays (Ki = 3 µM at the central site and 13 µM at the peripheral site). Wolfman et al. extended this in 1994 by isolating chrysin from Passiflora coerulea and demonstrating anxiolytic effects in the elevated plus maze in mice at 1 mg/kg, with the effect abolished by pretreatment with the benzodiazepine-receptor antagonist Ro 15-1788 (flumazenil) — pointing to the BDZ-site mechanism. In the same study, chrysin at 0.6–30 mg/kg produced no muscle-relaxing effect in the horizontal wire test, while diazepam at 6 mg/kg did, and the authors postulated that chrysin is a partial agonist of the central benzodiazepine receptor.
The pharmacologic profile of chrysin at the BDZ site is partial-agonist with low-to-moderate affinity. Compared to a full agonist like diazepam (Ki ~10 nM), chrysin's affinity is in the micromolar range, and even at saturating concentrations chrysin produces only a fraction of the maximal positive modulation that diazepam produces. This is exactly the pharmacology one would design for a gentle anxiolytic: enough BDZ-site occupation to amplify GABAergic inhibition modestly, but never enough to clamp the chloride channel and produce the cognitive impairment, motor incoordination, amnestic effect, and dependence liability of full benzodiazepine agonists.
Bioavailability is a significant constraint. Chrysin has poor oral bioavailability in humans (typically < 1% reported in pharmacokinetic studies), with extensive first-pass metabolism producing chrysin glucuronide and sulfate conjugates. This raises the legitimate question of whether enough free chrysin reaches the brain after an oral passionflower dose to account for the clinical effect. The answer is probably partly chrysin and partly the other actives discussed below — benzoflavones, additional flavone aglycones, and the still-undefined contribution of the harman alkaloids. The whole-extract is more active than isolated chrysin would predict, consistent with multi-component synergy.
Benzoflavones: The Second Active Scaffold
Dhawan and colleagues searched Passiflora incarnata methanol extract by bioassay-guided fractionation. Their 2001 study found a fraction with significant anxiolytic activity at 10 mg/kg in mice in the elevated plus maze, and proposed that a compound with a benzoflavone nucleus was responsible; later papers by the same author describe a tri-substituted benzoflavone moiety (BZF) isolated from the extract. The benzoflavone is structurally distinct from chrysin — an additional fused benzene ring extends the flavone scaffold.
An independent laboratory (Holbik and colleagues, 2010) then tried to isolate the compound from passionflower herb grown in India, Italy and France. A compound with the published characteristics was found in trace amounts only in the Italian material, and no traces were found in the Indian or French herb. The authors concluded that the benzoflavone is not the active principle of the herb and should not serve as an active marker.
Studies by Dhawan, summarised in a 2003 review of the author's own work, reported for the benzoflavone moiety:
- Reversal of morphine tolerance and dependence in mice (Dhawan 2002)
- Reversal of nicotine tolerance and dependence in mice (Dhawan 2002)
- Reversal of cannabinoid (delta-9-THC) tolerance in mice (Dhawan 2002)
- Improved sexual function, sperm count and litter size in 2-year-old male rats, alongside chrysin (Dhawan 2002)
The mechanism by which the benzoflavone produces these diverse effects is not fully characterized but likely involves modulation of multiple receptor systems including the gamma-aminobutyric acid-A receptor, possibly the cannabinoid CB1 receptor (theorized but not confirmed), and downstream effects on stress-hormone axes. The reversal-of-tolerance effects across opiate, nicotine, and cannabinoid models is a particularly intriguing common-pathway finding that has guided the use of passionflower in addiction medicine.
Standardization of passionflower extracts to benzoflavone content (rather than chrysin or vitexin) has been proposed by some authors as more clinically meaningful, but commercial standardization remains heterogeneous — some products specify vitexin equivalents, others specify total flavonoid content, others use no standardization at all. The independent 2010 analysis described above concluded that the benzoflavone should not serve as an active marker.
Comparison: Apigenin (Chamomile) and Bacopa
Several other widely used botanical anxiolytics work through the same gamma-aminobutyric acid-A benzodiazepine binding site as chrysin, with structurally similar flavone scaffolds:
- Apigenin (chamomile) — structurally chrysin + a 4'-hydroxyl on the B-ring (so apigenin = 4',5,7-trihydroxyflavone). Apigenin binds the benzodiazepine site with similar affinity to chrysin and produces similar partial-agonist effects. Chamomile's anxiolytic effect is documented in the Amsterdam 2009 GAD trial. Apigenin is generally considered slightly milder than chrysin in animal models, consistent with chamomile's clinical reputation as gentler than passionflower
- Bacopasides (Bacopa monnieri) — the triterpene saponins of bacopa modulate gamma-aminobutyric acid-A receptors among multiple other targets (including serotonin, dopamine, and cholinergic systems). Bacopa is more often used for cognitive enhancement than anxiolysis specifically, but the gamma-aminobutyric acid mechanism contributes to its calming side effect
- Honokiol and magnolol (Magnolia officinalis) — biphenolic compounds that modulate gamma-aminobutyric acid-A through a site distinct from the benzodiazepine site. Stronger sedative effect than passionflower
- Skullcap (Scutellaria baicalensis) — the flavone baicalein has BDZ-site affinity. Used in traditional Chinese medicine for anxiety
- Hops (Humulus lupulus) — 2-methyl-3-buten-2-ol and related compounds at gamma-aminobutyric acid-A site. Often combined with passionflower and valerian in sleep formulations
- Wild lettuce (Lactuca virosa) — lactucin and lactucopicrin produce mild sedation through poorly characterized gamma-aminobutyric acid modulation
The therapeutic implication of this large family of gamma-aminobutyric acid-A modulating flavones is that combination herbal formulations can layer multiple low-affinity ligands to produce additive effect without redundancy. A formulation containing passionflower + chamomile + skullcap may produce more robust anxiolysis than any single herb alone at comparable total dose, while maintaining the cognitive-preservation profile of partial-agonist pharmacology.
Non-Benzodiazepine-Site Gamma-Aminobutyric Acid-A Modulation
An important pharmacologic nuance: not all of passionflower's activity on the gamma-aminobutyric acid system runs through the benzodiazepine binding site. The Appel 2011 laboratory study tested a dry extract of Passiflora incarnata on rat brain tissue. The extract slowed the uptake of gamma-aminobutyric acid into rat cortical nerve endings (synaptosomes), but did not change its release or its breakdown by the enzyme GABA transaminase. It blocked radioligand binding at both gamma-aminobutyric acid-A and gamma-aminobutyric acid-B receptors, and in a further assay it behaved as a gamma-aminobutyric acid-B receptor antagonist (blocker). The benzodiazepine site and the ethanol (alcohol) site of the gamma-aminobutyric acid-A receptor were not affected by the extract.
The Elsas 2010 study, in hippocampal brain slices, found that whole passionflower extract produced prominent, dose-dependent direct gamma-aminobutyric acid-A currents, but not the expected modulation of synaptic gamma-aminobutyric acid-A currents. The currents came from gamma-aminobutyric acid contained in the extract itself (see GABA Itself Is in the Extract).
Harman Beta-Carboline Alkaloids and MAO-A
Beyond flavonoids, Passiflora incarnata contains trace amounts of beta-carboline alkaloids in the harman family — harman (1-methyl-beta-carboline), harmine (1-methyl-7-methoxy-beta-carboline), harmaline (the dihydro analog of harmine), and harmol (the 7-hydroxy analog). These compounds are weak reversible inhibitors of monoamine oxidase A (MAO-A), the enzyme that catabolizes serotonin, norepinephrine, and dietary tyramine.
The harman alkaloid content in passionflower is low — typically reported in the range of 0.01-0.1% of dried herb weight, with substantial variation across cultivars, growing conditions, and harvest timing. The pharmacologically relevant concentrations achieved with normal therapeutic passionflower doses are well below those required to produce clinically meaningful MAO inhibition in vivo. For comparison, the same beta-carboline alkaloids in much higher concentration in the Amazonian vine Banisteriopsis caapi (ayahuasca) do produce potent MAO-A inhibition, but at orders-of-magnitude higher concentration than is achieved with normal passionflower dosing.
That said, the presence of these alkaloids creates a theoretical concern for drug interactions:
- Selective serotonin reuptake inhibitors and serotonin-norepinephrine reuptake inhibitors (SNRIs) — theoretical risk of serotonin syndrome from additive serotonin elevation. Clinical reports with passionflower alone are essentially absent; the interaction remains theoretical
- Prescribed monoamine oxidase inhibitors (phenelzine, tranylcypromine, selegiline) — theoretical additive MAO inhibition. The concern is a precautionary one, since the actual MAO-inhibitor contribution of passionflower is minimal
- Tyramine-containing foods — the classic monoamine oxidase inhibitor (MAOI) dietary interaction. Not a real concern at normal passionflower doses but worth understanding the underlying mechanism
- Triptans (sumatriptan, etc.) — theoretical serotonin syndrome risk; clinically not documented
- Tramadol, meperidine — theoretical risk; clinically not documented
The Avula 2012 work developed a UPLC method that measures five beta-carboline (indole) alkaloids and four flavonoids together in several Passiflora species and in dietary supplements that claim to contain Passiflora, providing an analytical basis for quality-control standardization. Most clinical concerns about MAO-mediated interactions are theoretical rather than documented in practice; the actual clinical safety record of passionflower in routine use is excellent.
Why Partial Agonism Produces Gentler Effects
The partial-agonist character of chrysin and benzoflavones at the gamma-aminobutyric acid-A benzodiazepine site is the central mechanistic explanation for passionflower's gentler clinical profile relative to prescription benzodiazepines. The pharmacologic principle:
- Full agonist (diazepam, alprazolam, lorazepam) — produces maximal positive modulation of gamma-aminobutyric acid-A current at saturating concentration. The receptor functions at its maximum gain. At therapeutic doses, occupancy of the BDZ site is high (50-90% in positron emission tomography (PET) imaging studies), producing strong global GABAergic inhibition. The result is robust anxiolysis but also cognitive impairment, motor incoordination, amnesia, sedation, and (with chronic use) downregulation of gamma-aminobutyric acid-A receptors producing tolerance and physiologic dependence
- Partial agonist (chrysin, benzoflavones) — produces only a fraction of the maximal positive modulation, even at saturating concentration. Plus, low affinity means that at clinically achievable concentrations, BDZ-site occupancy is modest (likely 10-30% in animal models). The combined effect is modest amplification of basal gamma-aminobutyric acid-A current — enough to reduce pathologic anxiety but insufficient to clamp arousal, cognition, or motor coordination
The partial-agonist profile also has a self-limiting ceiling on effect: increasing the dose beyond a certain point does not produce proportionally more anxiolysis because the inherent intrinsic activity of the molecule is limited. This is why passionflower has an excellent overdose safety profile — it is essentially impossible to produce life-threatening respiratory depression with passionflower alone, in contrast to benzodiazepines (especially in combination with opioids or alcohol).
The trade-off is that severe acute anxiety, panic attacks, status epilepticus, or severe insomnia — situations that require maximal gamma-aminobutyric acid-A potentiation — will not be adequately treated by passionflower or any partial-agonist botanical. Full benzodiazepine agonism remains the standard for these acute indications.
Tolerance, Dependence, and Withdrawal Profile
The published clinical and observational evidence base for passionflower does not document significant tolerance development, physiologic dependence, or withdrawal syndrome with chronic use. This is mechanistically consistent with the low-occupancy, partial-agonist binding profile:
- Tolerance — full benzodiazepine agonists produce tolerance through gamma-aminobutyric acid-A receptor downregulation and subunit composition shifts in chronic use. The signaling required to drive these adaptive changes is proportional to receptor occupancy and activation. Partial agonists at low occupancy do not generate enough adaptive signaling to produce meaningful tolerance over weeks-to-months of chronic dosing
- Physiologic dependence — the molecular basis of benzodiazepine dependence is the same downregulation that drives tolerance. Without downregulation, abrupt discontinuation does not produce a rebound hyperexcitable state. Passionflower discontinuation does not produce documented withdrawal in clinical use
- Psychological dependence — possible in patients who have come to associate the ritual of taking passionflower with sleep onset or anxiety relief. Generally mild and reversible when the routine is tapered
A 2020 systematic review of nine randomized clinical trials, lasting from one day up to 30 days in adults, found that most reported reduced anxiety after passionflower preparations, with the effect less evident in people with mild anxiety symptoms. No adverse effects, including memory loss or collapse of psychometric functions, were observed.
This favorable profile is one of the main reasons passionflower has a legitimate role in benzodiazepine tapering protocols, where its mild gamma-aminobutyric acid-A potentiation can help ease the rebound anxiety and insomnia of taper without becoming a substitute dependence target.
Flumazenil Blocked Chrysin and the Whole Extract in Mice
Flumazenil is a pharmaceutical antagonist at the gamma-aminobutyric acid-A benzodiazepine binding site, used in the emergency department to reverse benzodiazepine overdose. A purely BDZ-site ligand should have its effect completely blocked by flumazenil pretreatment.
In a 2008 mouse study, a characterized Passiflora incarnata extract given by mouth at 375 mg/kg had an anxiolytic effect in the elevated plus maze comparable to diazepam (1.5 mg/kg), with a U-shaped dose-response curve. Flumazenil effectively blocked this effect, while the serotonin 5-HT1A receptor blocker WAY-100635 did not. The Wolfman 1994 work with isolated chrysin likewise found that pretreatment with flumazenil (Ro 15-1788) abolished chrysin's effect in the elevated plus maze, consistent with BDZ-site action. Neither the Appel 2011 nor the Elsas 2010 study tested flumazenil.
These animal results sit alongside the laboratory findings above: in rat brain tissue the extract slowed gamma-aminobutyric acid uptake and bound gamma-aminobutyric acid-A and gamma-aminobutyric acid-B receptors without acting at the benzodiazepine site (Appel 2011), and gamma-aminobutyric acid contained in the extract produced direct gamma-aminobutyric acid-A currents in brain slices (Elsas 2010). Passionflower extract therefore acts on the gamma-aminobutyric acid system in more than one way, and the whole-extract pharmacology is more complex than isolated chrysin would predict. A 2011 review of flavonoids and gamma-aminobutyric acid-A receptors lists flumazenil-insensitive modulation by some flavonoids as one area of research interest.
The findings also fit the general principle that whole-plant botanical pharmacology is rarely reducible to a single isolated active compound.
Theoretical and Real Drug Interaction Concerns
- Benzodiazepines and Z-drugs — theoretical additive gamma-aminobutyric acid-A potentiation. Practically, the additive effect is mild because passionflower's contribution is modest. Useful in benzodiazepine tapering; the added sedation with full agonists matters most in elderly or frail people
- Alcohol — additive central nervous system (CNS) depression via gamma-aminobutyric acid-A modulation and other mechanisms. The added sedation from significant alcohol intake with passionflower matters most for driving or operating machinery
- Opioids — theoretical additive sedation. Useful in opioid withdrawal protocols (see Withdrawal & Addiction Support) under supervision; recreational opioid use combined with passionflower at home adds sedation on top of the opioid
- Sedating antihistamines (diphenhydramine, doxylamine) — additive sedation
- Sedating antidepressants (trazodone, mirtazapine, doxepin) — additive sedation; sometimes combined for stubborn insomnia, where excessive morning sedation is the concern
- Selective serotonin reuptake inhibitors/serotonin-norepinephrine reuptake inhibitors — theoretical serotonin elevation from harman MAO-A inhibition. Clinically not a documented concern at normal doses
- Prescribed monoamine oxidase inhibitors (rare) — theoretical additive MAO inhibition; the concern is precautionary
- Warfarin and other anticoagulants — some sources suggest theoretical platelet effects from passionflower flavonoids; clinical reports of bleeding are absent; the platelet effect is theoretical
- General anesthesia — standard practice is to stop herbal sedatives 1-2 weeks before scheduled surgery as precaution. Probably overcautious but the standard recommendation
- Pregnancy — insufficient safety data plus theoretical uterine stimulant effects from harman alkaloids
- Breastfeeding — limited safety data in breastfeeding
A laboratory study published in 2026 found that a standardized passionflower extract also bound adenosine A1, adenosine A2A and serotonin 5-HT2A receptors (but not melatonin MT1 or orexin OX1 receptors), and slowed the uptake of dopamine, norepinephrine and serotonin into rat brain nerve endings — actions beyond the gamma-aminobutyric acid system that bear on the serotonin-interaction question above. It was an exploratory test-tube study; it did not test people.
GABA Itself Is in the Extract
A 2010 study (Elsas and colleagues) found that gamma-aminobutyric acid itself is a prominent ingredient of passionflower extract. Whole extract produced prominent, dose-dependent gamma-aminobutyric acid-A currents in hippocampal brain slices, and these currents were absent when the amino acids were removed from the extract.
The same study showed that the way the herb is extracted changes what is in it: from the same batch of plant material, hot extraction gave substantially higher total flavonoid yields than cold extraction. Five different extracts from a single batch were then given to mice in their drinking water for one week. Two of the five protected the mice against chemically induced (pentylenetetrazol) seizures. Instead of the anxiolytic effects described by other groups, all five extracts produced more anxiety-like behaviour (anxiogenic effects) in the elevated plus maze.
Key Research Papers
- Medina JH, Paladini AC, Wolfman C, Levi de Stein M, Calvo D, Diaz LE, Pena C (1990). Chrysin (5,7-di-OH-flavone), a naturally occurring ligand for benzodiazepine receptors, with anticonvulsant properties. Biochemical Pharmacology, 40(10), 2227-2231. — PubMed PMID: 2173925
- Wolfman C, Viola H, Paladini A, Dajas F, Medina JH (1994). Possible anxiolytic effects of chrysin, a central benzodiazepine receptor ligand isolated from Passiflora coerulea. Pharmacology Biochemistry and Behavior, 47(1), 1-4. — PubMed PMID: 7906886
- Dhawan K, Kumar S, Sharma A (2001). Anti-anxiety studies on extracts of Passiflora incarnata Linneaus. Journal of Ethnopharmacology, 78(2-3), 165-170. — PubMed PMID: 11694362
- Dhawan K, Dhawan S, Sharma A (2004). Passiflora: a review update. Journal of Ethnopharmacology, 94(1), 1-23. — PubMed PMID: 15261959
- Marder M, Paladini AC (2002). GABA-A-receptor ligands of flavonoid structure. Current Topics in Medicinal Chemistry, 2(8), 853-867. — PubMed PMID: 12171576
- Appel K, Rose T, Fiebich B, Kammler T, Hoffmann C, Weiss G (2011). Modulation of the gamma-aminobutyric acid (GABA) system by Passiflora incarnata L. Phytotherapy Research, 25(6), 838-843. — PubMed PMID: 21089181
- Elsas SM, Rossi DJ, Raber J, White G, Seeley CA, Gregory WL, Mohr C, Pfankuch T, Soumyanath A (2010). Passiflora incarnata L. (passionflower) extracts elicit GABA currents in hippocampal neurons in vitro, and show anxiogenic and anticonvulsant effects in vivo, varying with extraction method. Phytomedicine, 17(12), 940-949. — PubMed PMID: 20382514
- Salgueiro JB, Ardenghi P, Dias M, Ferreira MB, Izquierdo I, Medina JH (1997). Anxiolytic natural and synthetic flavonoid ligands of the central benzodiazepine receptor have no effect on memory tasks in rats. Pharmacology Biochemistry and Behavior, 58(4), 887-891. — PubMed PMID: 9408191
- Avula B, Wang YH, Rumalla CS, Smillie TJ, Khan IA (2012). Simultaneous determination of alkaloids and flavonoids from aerial parts of Passiflora species and dietary supplements using UPLC-UV-MS and HPTLC. Natural Product Communications, 7(9), 1177-1180. — PubMed PMID: 23074901
- Sigel E, Steinmann ME (2012). Structure, function, and modulation of GABA-A receptors. Journal of Biological Chemistry, 287(48), 40224-40231. — PubMed PMID: 23038269
- Hanrahan JR, Chebib M, Johnston GA (2011). Flavonoid modulation of GABA(A) receptors. British Journal of Pharmacology, 163(2), 234-245. — PubMed PMID: 21244373
- Johnston GA (2015). Flavonoid nutraceuticals and ionotropic receptors for the inhibitory neurotransmitter GABA. Neurochemistry International, 89, 120-125. — PubMed PMID: 26190180
- Dhawan K, Kumar S, Sharma A (2002). Beneficial effects of chrysin and benzoflavone on virility in 2-year-old male rats. Journal of Medicinal Food, 5(1), 43-48. — PubMed PMID: 12511112
- Dhawan K (2003). Drug/substance reversal effects of a novel tri-substituted benzoflavone moiety (BZF) isolated from Passiflora incarnata Linn.—a brief perspective. Addiction Biology, 8(4), 379-386. — PubMed PMID: 14690874
- Holbik M, Krasteva S, Mayer N, Kählig H, Krenn L (2010). Apparently no sedative benzoflavone moiety in passiflorae herba. Planta Medica, 76(7), 662-664. — PubMed PMID: 20301055
- Grundmann O, Wang J, McGregor GP, Butterweck V (2008). Anxiolytic activity of a phytochemically characterized Passiflora incarnata extract is mediated via the GABAergic system. Planta Medica, 74(15), 1769-1773. — PubMed PMID: 19006051
- Janda K, Wojtkowska K, Jakubczyk K, Antoniewicz J, Skonieczna-Żydecka K (2020). Passiflora incarnata in Neuropsychiatric Disorders-A Systematic Review. Nutrients, 12(12), 3894. — PubMed PMID: 33352740
- Appel K, Schwarzensteiner I, Zimmermann C, Tober C, Günnewich N (2027). A Passiflora incarnata extract exerts multi-target effects on selected sleep-related receptors. Journal of Ethnopharmacology, 372, 122198 (published online 2026). — PubMed PMID: 42462921
PubMed Topic Searches
Connections
- All Herbs
- Passionflower Overview
- Passionflower Benefits Hub
- Passionflower for Anxiety Relief
- Passionflower for Sleep Quality
- Passionflower for Withdrawal
- Chamomile (Apigenin)
- Valerian (Valerenic Acid)
- Lavender (Linalool)
- Lemon Balm (Rosmarinic Acid)
- Kava (Kavalactones)
- Magnesium (Gamma-Aminobutyric Acid Cofactor)
- Anxiety
- Insomnia
- Natural Anxiety Relief
- Stress Management
- History