⚠ Evidence warning: Clinical trials or other evidence do not support the claim that tyrosine supplements help thyroid function in low iodine or subclinical hypothyroidism. This page keeps it as a report of what people, websites or other media say.
Tyrosine — Benefits Deep Dive
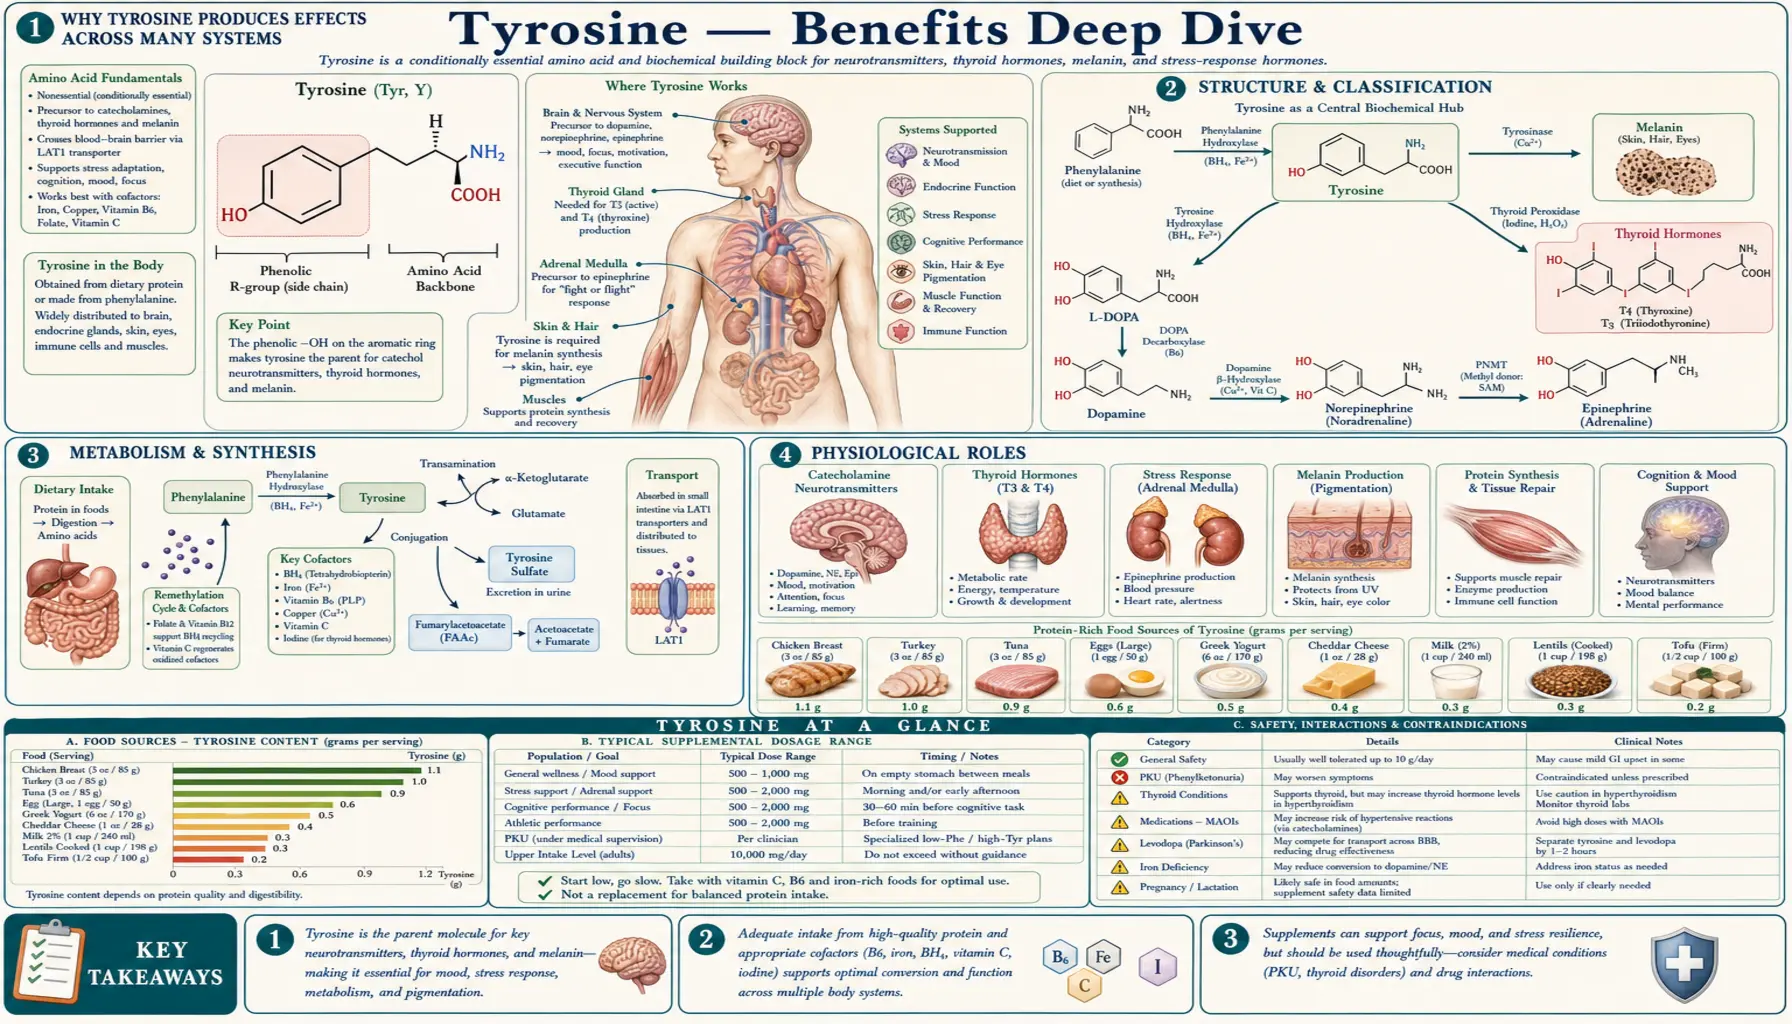
Tyrosine is the conditionally essential aromatic amino acid synthesized from phenylalanine by hepatic phenylalanine hydroxylase. It is the precursor of the entire catecholamine cascade — dopamine, norepinephrine, and epinephrine all begin as a single hydroxylation of tyrosine to L-DOPA. It is the substrate backbone of every molecule of thyroid hormone in the body, with T4 and T3 assembled as iodinated tyrosine pairs on the thyroglobulin scaffold. It is the source of all melanin in skin, hair, and eye, via tyrosinase-catalyzed conversion to dopaquinone. And it is the amino acid whose depletion under acute stress causes the cognitive performance failure observed in cold, hypoxia, and sleep deprivation operational trials, the substrate-limitation mechanism that tyrosine pre-loading is reported to prevent, though study results vary (see below). Four benefit pages below explore the conditions where tyrosine produces the largest documented clinical effect — stress and cognitive performance under operational demand, the catecholamine cascade and mood, the thyroid hormone substrate chemistry, and the cold-tolerance applications that founded the modern military operational supplement literature.
Deep-Dive Articles
Stress & Cognitive Performance
The Banderet & Lieberman 1989 USARIEM cold-plus-hypoxia trial and the Neri 1995 sleep-deprivation trial, the substrate-limitation model of catecholamine depletion under stress, the 100–150 mg/kg dose-response window, the 30–60 minute pre-load timing, military and aviation operational applications, and the cleanly negative finding that tyrosine produces no benefit in unstressed subjects.
Read the deep dive →Dopamine & Mood
Tyrosine hydroxylase as the rate-limiting enzyme in catecholamine synthesis, the tyrosine → DOPA → dopamine → norepinephrine → epinephrine cascade, the three brain dopamine systems (nigrostriatal motor, mesolimbic motivation, tuberoinfundibular prolactin), the tetrahydrobiopterin (BH4) cofactor and its iron and folate dependencies, the mixed evidence for tyrosine in depression (Gelenberg 1990 negative trial), the foundational Wood 1985 attention-deficit/hyperactivity disorder (ADHD) pilot, and the comparison to methylphenidate and amphetamine.
Read the deep dive →Thyroid Function
Thyroid hormone is made of tyrosine. T4 is two tyrosine residues joined ether-style with four iodines; T3 is the same with three iodines. The thyroid peroxidase (TPO) + iodide + tyrosyl assembly reaction on the thyroglobulin scaffold, the monoiodotyrosine/diiodotyrosine (MIT/DIT) coupling reactions producing T4 versus T3, the selenium-dependent peripheral deiodination, iodine as the universally limiting substrate, the realistic clinical role in subclinical hypothyroidism, and the hyperthyroidism contraindication.
Read the deep dive →Cold Tolerance
The Shurtleff 1994 cold-only working memory trial, the Mahoney 2007 repeat-cold paradigm, the O'Brien 2007 whole-body cooling protocol, the catecholamine demand of vasoconstriction plus shivering plus locus-coeruleus arousal during sustained cold exposure, the combined cold-plus-altitude-plus-sleep-loss operational profile, the Special Forces protocol, cold-water diving applications, and the explicit limits (will not prevent frostbite or hypothermia).
Read the deep dive →Interactive Visualization Dopamine, Reward & How Habits Hijack You Dopamine is not the pleasure chemical. Watch the spike migrate from the reward to the cue — then withhold the reward and see it dip below zero. That dip is craving. Launch →
Table of Contents
- Deep-Dive Articles
- Why Tyrosine Produces Effects Across Many Systems
- Research Papers: Stress & Cognitive Performance
- Research Papers: Dopamine & Mood
- Research Papers: Thyroid Function
- Research Papers: Cold Tolerance
- Research Papers: Cross-Cutting (Metabolism, PKU, Melanin)
- External Authoritative Resources
- Connections
- Featured Videos
Why Tyrosine Produces Effects Across Many Systems
Most amino acids act primarily as building blocks of protein, with only modest signaling or precursor roles. Tyrosine is unusual because a single amino acid molecule feeds four distinct hormone and neurotransmitter cascades, each of which has its own clinical literature and supplementation use case. The unusual versatility comes from the structural chemistry of the aromatic ring, which is amenable to multiple downstream modifications (hydroxylation, iodination, decarboxylation, beta-hydroxylation, methylation, oxidation to quinone) each producing a different bioactive end product.
- Catecholamine cascade (tyrosine → DOPA → dopamine → norepinephrine → epinephrine) — the rate-limiting enzyme is tyrosine hydroxylase (TH), which converts tyrosine to L-DOPA using oxygen and tetrahydrobiopterin cofactor with iron in the active site. From L-DOPA the cascade is fast: aromatic L-amino acid decarboxylase (AADC, vitamin B6-dependent) gives dopamine, dopamine beta-hydroxylase (DBH, copper- and vitamin C-dependent) gives norepinephrine, phenylethanolamine N-methyltransferase (PNMT, S-adenosylmethionine-dependent) gives epinephrine. Different cell types express different cascade fragments — dopaminergic neurons stop at dopamine, noradrenergic neurons at norepinephrine, adrenal medullary chromaffin cells go all the way to epinephrine. This is the mechanism behind tyrosine's stress / cognitive performance effects, the dopamine and mood applications, and the cold tolerance support.
- Thyroid hormone synthesis (tyrosine → monoiodotyrosine → diiodotyrosine → T4, T3) — thyroid peroxidase catalyzes the iodination of tyrosyl residues embedded in the thyroglobulin scaffold inside thyroid follicles, then catalyzes the coupling of two iodinated tyrosines into a thyronine. Two tyrosines per thyroid hormone molecule. Selenium-dependent deiodinases then convert T4 to active T3 (or to inactive reverse T3) in peripheral tissues. This is the mechanism behind tyrosine's role in thyroid hormone synthesis, where the substrate logic is sound but supplementation is reported to help only in marginal-iodine populations or in subclinical hypothyroidism.
- Melanin synthesis (tyrosine → DOPA → dopaquinone → eumelanin / pheomelanin) — the enzyme tyrosinase (copper-dependent) oxidizes tyrosine to DOPA and then to dopaquinone, which polymerizes to form eumelanin (the brown-black pigment) or, in combination with cysteine, pheomelanin (the red-yellow pigment). Loss-of-function mutations in tyrosinase cause oculocutaneous albinism type 1, with complete absence of melanin in skin, hair, and eyes. The dopaquinone intermediate is highly reactive and the same redox chemistry that produces pigment also contributes to melanocyte oxidative stress and melanoma vulnerability.
- Trace amine cascade (tyrosine → tyramine → octopamine) — aromatic L-amino acid decarboxylase also acts on tyrosine to produce tyramine without the prior hydroxylation. Tyramine is the trace amine in aged cheeses, cured meats, and fermented foods responsible for the MAO-inhibitor "cheese reaction" hypertensive crisis. Further beta-hydroxylation of tyramine by dopamine beta-hydroxylase gives octopamine, a vertebrate trace amine with modest sympathomimetic activity. This minor pathway is the reason MAO inhibitors require dietary tyramine restriction.
The unifying observation is that one rate-limiting amino acid feeds four hormone and neurotransmitter cascades. This is also why tyrosine status is rarely the rate-limiting factor for any single cascade in adequately fed adults — the tyrosine supply must be divided across all four downstream uses, but the systemic tyrosine flux from dietary protein and from hepatic phenylalanine hydroxylation is large compared to any single cascade's demand. The exception is acute stress, where one cascade (catecholamines) acutely accelerates to substrate-limiting demand, producing the conditions where supplementation matters.
What is not settled: a 2015 review (Jongkees) reports that results "vary considerably, with some studies finding beneficial effects, whereas others do not." It describes the potential for treating clinical disorders as limited, with any benefit likely depending on the presence and extent of impaired neurotransmitter function and synthesis, and the potential for physical exercise as minimal. It concludes that tyrosine does seem to enhance thinking performance, particularly in short-term stressful or mentally demanding situations, but only when neurotransmitter function is intact and dopamine or norepinephrine is temporarily depleted.
Age may change the response. In a trial of 17 adults aged 60–75 given single doses of 100, 150 or 200 mg/kg (van de Rest 2017), blood tyrosine rose more than in 17 young adults on the same 150 mg/kg dose, and working memory fell at higher doses (P=0.048). That range overlaps the 100–150 mg/kg dose described on the Stress & Cognitive Performance page. The older adults' comparison was between doses; the abstract lists no placebo arm.
The therapeutic complication that runs through every benefit page is the redox chemistry of the dopamine and DOPA intermediates. Both can spontaneously oxidize to dopaquinone and downstream reactive quinones if not properly compartmentalized in synaptic vesicles or in melanosomes. The same chemistry that produces pigment, when it occurs in dopaminergic neurons of the substantia nigra, contributes to the selective vulnerability of those neurons in Parkinson's disease. This is why patients on L-DOPA require careful management and why catecholamine biology straddles the line between essential function and oxidative liability.
Research Papers: Stress & Cognitive Performance
- Banderet LE, Lieberman HR (1989), classic USARIEM cold-plus-hypoxia tyrosine trial — PubMed: Banderet 1989
- Neri DF et al. (1995), sleep-deprivation tyrosine trial in aviation operators — PubMed: Neri 1995
- Jongkees BJ et al. (2015), comprehensive review of tyrosine for cognitive stress applications — PubMed PMID: 26424423
- van de Rest O et al. (2017), dose-dependent effects of oral tyrosine on plasma tyrosine levels and cognition in aging — PubMed PMID: 29168741
- Deijen JB, Orlebeke JF (1994), tyrosine for cognitive function under stress — PubMed: Deijen 1994
- Deijen JB et al. (1999), tyrosine in cadets after combat training course — PubMed: Deijen 1999
- Lieberman HR et al. (2005), "fog of war" cognitive degradation under combat-like stress — PubMed: Lieberman 2005
- Magill RA et al. (2003), tyrosine vs amphetamine vs caffeine under sleep deprivation — PubMed: Magill 2003
- Thomas JR et al. (1999), tyrosine and working memory in multitasking — PubMed: Thomas 1999
- Hase A et al. (2015), tyrosine effects in healthy adults (mixed evidence) — PubMed: Hase 2015
- Fernstrom JD, Fernstrom MH (2007), comprehensive review of tyrosine and catecholamine function in brain — PubMed: Fernstrom review
Research Papers: Dopamine & Mood
- Nagatsu T et al. (1964), original characterization of tyrosine hydroxylase as initial step in norepinephrine biosynthesis — PubMed: Nagatsu 1964
- Daubner SC et al. (2011), tyrosine hydroxylase regulation and dopamine synthesis — PubMed: Daubner 2011
- Gelenberg AJ et al. (1990), tyrosine for depression double-blind trial (negative result) — PubMed: Gelenberg 1990
- Wood DR et al. (1985), foundational adult ADHD pilot trial of phenylalanine/tyrosine — PubMed: Wood 1985
- Reimherr FW et al. (1987), follow-up L-tyrosine trial in adult ADHD with tolerance development — PubMed: Reimherr 1987
- Volkow ND et al. (2009), dopamine reward pathway in ADHD — PubMed: Volkow ADHD
- Werner ER et al. (2011), tetrahydrobiopterin biochemistry and BH4 cofactor pathway — PubMed: Werner 2011
- Beard JL (2003), iron deficiency and brain dopamine function — PubMed: Beard iron and dopamine
- Goldstein DS, Eisenhofer G, Kopin IJ (2003), plasma catecholamines and metabolites in humans — PubMed: Goldstein review
- Lemoine P et al. (1989), L-tyrosine: a long term treatment of Parkinson's disease (report of ten patients, in French) — PubMed PMID: 2502304
Research Papers: Thyroid Function
- Carvalho DP, Dupuy C (2017), thyroid hormone biosynthesis and release biochemistry — PubMed: Carvalho thyroid biosynthesis
- Ruf J, Carayon P (2006), thyroid peroxidase (TPO) structure and function — PubMed: TPO review
- Di Jeso B, Arvan P (2016), thyroglobulin molecular biology to clinical endocrinology — PubMed: Thyroglobulin review
- Bianco AC et al. (2002), iodothyronine selenodeiodinases for peripheral T4→T3 conversion — PubMed: Bianco deiodinases
- Zimmermann MB (2009), global iodine deficiency review — PubMed: Iodine deficiency
- Toulis KA et al. (2010), selenium supplementation in Hashimoto's meta-analysis — PubMed: Selenium Hashimoto's
- Drutel A et al. (2013), selenium and the thyroid gland clinical review — PubMed: Selenium thyroid
- Garber JR et al. (2012), AACE/ATA hypothyroidism clinical practice guideline — PubMed: Hypothyroidism guideline
- Pearce EN et al. (2013), global iodine nutrition update — PubMed: Pearce iodine
- Stathatos N (2012), thyroid physiology review — PubMed: Stathatos thyroid
Research Papers: Cold Tolerance
- Shurtleff D et al. (1994), tyrosine reverses cold-induced working memory deficit — PubMed: Shurtleff 1994
- Mahoney CR et al. (2007), tyrosine and working memory during cold exposure — PubMed: Mahoney 2007
- O'Brien C et al. (2007), tyrosine and cognitive/psychomotor performance during body cooling — PubMed: O'Brien 2007
- Castellani JW, Young AJ (2016), human physiological responses to cold exposure — PubMed: Castellani cold physiology
- Cannon B, Nedergaard J (2004), brown adipose tissue thermogenesis review — PubMed: Cannon BAT
- Tipton MJ et al. (2017), cold-water immersion physiology — PubMed: Tipton cold water
- Stocks JM et al. (2004), human physiological responses to cold exposure operational review — PubMed: Stocks cold physiology
- Coull NA et al. (2015), tyrosine and physical performance in heat (contrast to cold) — PubMed: Coull 2015
- Lieberman HR (2003), nutrition, brain function, and cognitive performance — PubMed: Lieberman 2003
- Lieberman HR et al. (2008), calorie deprivation, cognition, sleep — PubMed PMID: 18779282
Research Papers: Cross-Cutting (Metabolism, PKU, Melanin)
- van Spronsen FJ et al. (2021), phenylketonuria pathophysiology and management — PubMed PMID: 34017006
- Phenylalanine hydroxylase (PAH) and the hepatic tyrosine synthesis reaction — PubMed: PAH hepatic
- Tyrosinase and melanin synthesis biochemistry — PubMed: Tyrosinase melanin
- Oculocutaneous albinism type 1 and tyrosinase loss-of-function — PubMed: OCA1 albinism
- Tyramine and the MAO-inhibitor "cheese reaction" — PubMed: Tyramine cheese reaction
- Hereditary tyrosinemia type I and fumarylacetoacetate hydrolase deficiency — PubMed: Tyrosinemia type I
- LAT1 large neutral amino acid transporter and blood-brain barrier tyrosine transport — PubMed: LAT1 transport
- Dopaquinone redox chemistry and melanocyte oxidative stress — PubMed: Dopaquinone redox
- Tyrosine catabolism pathway (homogentisate, fumarate, acetoacetate) — PubMed: Tyrosine catabolism
- Alkaptonuria and homogentisic acid oxidase deficiency — PubMed: Alkaptonuria
External Authoritative Resources
- National Academies — Dietary Reference Intakes: Protein and Amino Acids (2005), Chapter 10 — comprehensive scientific summary of tyrosine biochemistry and clinical applications
- U.S. National Institutes of Health (NIH) Office of Dietary Supplements — Tyrosine
- MedlinePlus — Amino acids
- PubMed — All clinical research on human tyrosine supplementation
- PubMed — Tyrosine hydroxylase research corpus
- USARIEM — U.S. Army Research Institute of Environmental Medicine (where the foundational Banderet 1989 cold + tyrosine trial was conducted)
Connections
- All Amino Acids
- Dopamine, Reward & How Habits Hijack You — interactive animation
- Tyrosine (Main Page)
- Tyrosine for Stress & Cognitive Performance
- Tyrosine for Dopamine & Mood
- Tyrosine for Thyroid Function
- Tyrosine for Cold Tolerance
- Phenylalanine (Precursor)
- Tryptophan
- Leucine
- Isoleucine
- Methionine
- Cysteine
- Depression
- Attention-Deficit/Hyperactivity Disorder
- Anxiety
- Fatigue
- Brain Fog
- Hashimoto's Thyroiditis
- Reverse T3 and Low T3 Syndrome
- Thyroid Panel
- Iodine (Thyroid Substrate Pair)
- Selenium (Deiodinase Cofactor)
- Iron (TH Cofactor)
- Vitamin B6 (AADC Cofactor)
- Vitamin C (DBH Cofactor)
- Vitamin A Benefits Hub
- History
- Sources