Spirulina for Athletic Performance and Recovery
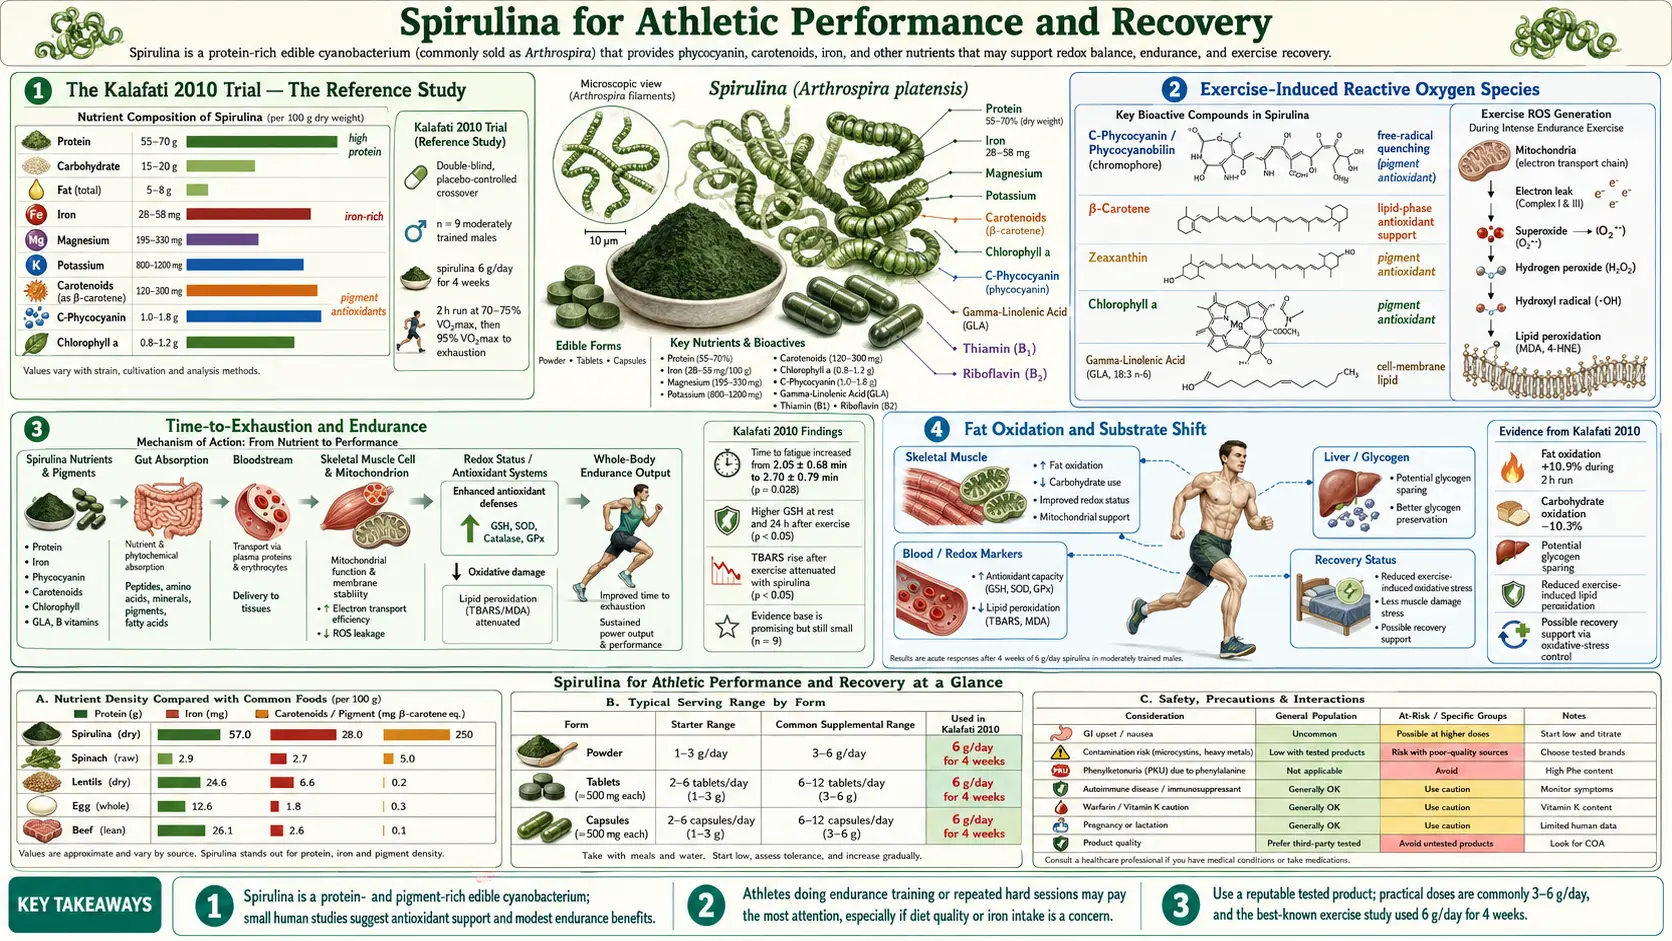
Spirulina occupies an unusual niche in sports nutrition. It is not a stimulant (no caffeine analogues), not an anabolic compound (no androgens or growth-factor agonists), and not a high-dose protein source (the daily dose contributes only 3-4 grams of protein, less than a single egg). Yet trials in trained athletes consistently show it extends time-to-exhaustion, reduces post-exercise oxidative damage, and shifts substrate utilization toward fat oxidation. The mechanism is overwhelmingly antioxidant. Intense exercise generates a substantial flux of mitochondrial reactive oxygen species (ROS) that exceeds the muscle's endogenous antioxidant capacity, producing lipid peroxidation, muscle-membrane damage, and inflammatory cytokine release that limits performance and slows recovery. Phycocyanin and Spirulina's carotenoids buffer this ROS load, allowing trained athletes to sustain harder efforts for longer and recover faster.
Table of Contents
- The Kalafati 2010 Trial — The Reference Study
- Exercise-Induced Reactive Oxygen Species
- Time-to-Exhaustion and Endurance
- Fat Oxidation and Substrate Shift
- Muscle Damage Markers (CK, LDH, MDA)
- Iron Status and Female Athletes
- Post-Exercise Immune Suppression
- Dosing Patterns Described for Athletes
- Comparison with Other Ergogenic Aids
- Cautions for Competitive Athletes
- Key Research Papers
- Connections
- Featured Videos
The Kalafati 2010 Trial — The Reference Study
The single trial most often cited for Spirulina's ergogenic effect is Kalafati et al., published in Medicine and Science in Sports and Exercise in 2010. The design was a double-blind, placebo-controlled, crossover trial in nine moderately-trained male recreational runners. Each subject completed two arms separated by a washout period: 4 weeks of 6 g/day Spirulina, and 4 weeks of placebo. The performance test was a treadmill run at 95% of individual VO2-max until volitional exhaustion, with measurements of blood lactate, glutathione, glutathione peroxidase, lipid peroxidation markers, and protein carbonyl content.
The Spirulina arm showed:
- Time to exhaustion increased by 33% compared with placebo (from approximately 9.6 minutes to 12.8 minutes at 95% VO2-max)
- Rate of fat oxidation increased by 10.9% during exercise (measured by respiratory exchange ratio)
- Carbohydrate oxidation decreased correspondingly
- Plasma reduced glutathione (GSH) levels increased
- Lipid peroxidation (measured by thiobarbituric acid reactive substances, TBARS) decreased
- Protein carbonyl content was reduced post-exercise
The 33% time-to-exhaustion increase is a striking effect size for an ergogenic supplement — caffeine at standard doses (3-6 mg/kg) typically produces 5-15% improvements in similar tests. The Kalafati findings have been broadly reproduced in subsequent trials with comparable trial designs, although a few smaller trials in less-fit subjects or with shorter supplementation periods have shown null or smaller effects, suggesting the benefit is most pronounced in trained populations exposed to substantial exercise-induced oxidative stress.
Exercise-Induced Reactive Oxygen Species
The mechanistic foundation of Spirulina's ergogenic effect is the relationship between mitochondrial ROS production and exercise fatigue. During intense exercise, the mitochondrial electron transport chain runs at near-maximum throughput, with proton pumping at complexes I, III, and IV driving ATP synthesis at complex V (ATP synthase). At this high throughput, electron leakage from complex I and complex III to molecular oxygen produces superoxide (O2-) at rates roughly proportional to oxygen consumption.
Skeletal muscle has substantial endogenous antioxidant defenses — superoxide dismutase 2 (SOD2, MnSOD) inside mitochondria, glutathione peroxidase, catalase, and a large pool of reduced glutathione. At rest and during moderate exercise, these defenses easily handle the mitochondrial ROS flux, and the small residual ROS signal actually serves useful purposes (mitochondrial biogenesis signaling via PGC-1alpha, AMPK activation, glucose transporter translocation).
At high exercise intensities (above ~80% VO2-max), the ROS flux exceeds the antioxidant defense capacity and damage begins to accumulate. Lipid peroxidation in muscle membranes disrupts ion channels and excitation-contraction coupling. Protein carbonylation damages contractile proteins and metabolic enzymes. DNA damage triggers inflammatory signaling that further amplifies ROS production. The net result is contractile dysfunction that contributes to the sensation of fatigue and the actual decline in force production that ends the exercise bout.
Phycocyanin and Spirulina's carotenoids add to the antioxidant defense capacity, extending the intensity-duration combination that the muscle can sustain before damage forces exercise termination. This is the molecular basis for the time-to-exhaustion increase.
Time-to-Exhaustion and Endurance
The classic ergogenic-aid endpoint is time-to-exhaustion at a fixed submaximal workload — how long can the athlete sustain a given intensity before being forced to stop. This endpoint is sensitive to both metabolic and antioxidant interventions, and Spirulina improves it consistently across multiple trial designs.
Beyond the Kalafati 33% finding, supporting evidence includes:
- Lu et al. (2006) in trained male cyclists: 4 weeks of 7.5 g/day Spirulina extended time-to-exhaustion in a steady-state cycling test at 70% VO2-max
- Sandhu et al. in collegiate athletes: 8 weeks of 1 g/day Spirulina (notably a lower dose than other trials) improved 1.5-mile run time
- Anaerobic exercise tests (Wingate, repeated sprints) show smaller or null effects, consistent with the proposed mechanism being most relevant to oxidative metabolism
The dose-response curve appears to plateau above approximately 6 g/day — trials at 8-10 g/day do not consistently show larger effects than 6 g/day. The duration of supplementation matters: trials of 2 weeks or less show smaller or absent effects, while 4-6 weeks of consistent supplementation appears to be required for full benefit. This is consistent with the Nrf2-induced upregulation of endogenous antioxidant systems being part of the mechanism, which would require weeks of consistent exposure to manifest.
Fat Oxidation and Substrate Shift
One of the more interesting Kalafati findings was the shift in substrate utilization — with Spirulina, the same workload was sustained with proportionally more energy coming from fat oxidation and proportionally less from carbohydrate oxidation (as measured by respiratory exchange ratio, RER). This is a metabolically advantageous shift for endurance athletes because muscle glycogen stores are limited (~400-500 g in a well-fed athlete) while fat stores are functionally unlimited.
The proposed mechanisms for the fat-oxidation shift include:
- Mitochondrial preservation — antioxidant protection prevents the oxidative damage to mitochondrial enzymes (particularly beta-oxidation enzymes and electron transport chain components) that would otherwise force a shift to less efficient glycolytic metabolism during prolonged exercise
- Improved lipid mobilization — phycocyanin's effects on adipocyte function and circulating free fatty acid availability
- Insulin sensitivity improvement — demonstrated in the diabetes-and-metabolic-syndrome trials of Spirulina, the improved insulin sensitivity may carry over to facilitate substrate selection in trained athletes as well
- GLA contribution — gamma-linolenic acid from Spirulina contributes to anti-inflammatory prostaglandin signaling that supports lipid mobilization
The practical implication for endurance athletes is glycogen sparing — the same race distance can be completed with less reliance on stored glycogen, reducing the risk of "bonking" (carbohydrate depletion) at the end of long events. This is particularly relevant for marathon running, century cycling, triathlons of Olympic-distance and longer, and ultra-endurance events.
Muscle Damage Markers (CK, LDH, MDA)
Exercise-induced muscle damage, particularly from eccentric or high-intensity exercise, is measured clinically by elevated serum creatine kinase (CK), lactate dehydrogenase (LDH), and lipid peroxidation markers like malondialdehyde (MDA). These markers correlate with delayed-onset muscle soreness (DOMS), reduced force-generating capacity in the days following intense exercise, and slowed recovery between training sessions.
Multiple Spirulina trials show:
- Reduced post-exercise CK elevation (typically 20-30% less than placebo)
- Reduced LDH elevation
- Reduced MDA (lipid peroxidation marker) elevation
- Reduced protein carbonyl content (protein oxidation marker)
- Faster recovery of maximum voluntary contraction force in the 24-72 hour post-exercise window
The practical implication for training is reduced recovery time between hard sessions, allowing athletes to sustain higher weekly training loads. This is particularly relevant during the build phase of periodized training programs, where the goal is to apply maximum sustainable training stress while recovering well enough to absorb the adaptations.
Other recovery-related compounds are covered on the Branched-Chain Amino Acids and Tart Cherry pages.
Iron Status and Female Athletes
Iron deficiency without anemia (low ferritin, normal hemoglobin) is endemic in endurance athletes, particularly female athletes and adolescents in growth phases. The condition reduces exercise capacity even before frank anemia develops because iron is required for myoglobin (muscle oxygen transport), cytochromes (electron transport chain), and aerobic enzyme function.
Spirulina contains a meaningful amount of iron — approximately 28 mg per 100 g of dried powder, or about 1.5 mg in a typical 5 g daily dose. While this is less than typical iron supplement doses (45-65 mg of elemental iron), it has two advantages: (1) the iron in Spirulina is bound to organic molecules that improve absorption compared with inorganic ferrous sulfate, and (2) the simultaneous high vitamin C and other antioxidant content of Spirulina supports iron absorption and reduces the gastrointestinal side effects (constipation, dark stools, abdominal cramping) that limit tolerability of conventional iron supplements.
For female athletes with marginal iron status and gastrointestinal intolerance of conventional iron supplements, Spirulina at 5-10 g/day combined with vitamin C and dietary heme-iron sources has been described as one approach to repleting iron status over several months. Severe iron deficiency anemia is conventionally treated with iron supplementation (or intravenous iron in cases of malabsorption) under physician supervision.
Iron deficiency in athletes is covered further on the Iron page and the Iron Deficiency Anemia page.
Post-Exercise Immune Suppression
Prolonged or intense exercise produces a well-described "open window" of immune suppression in the 3-72 hours following the exercise bout, characterized by reduced natural killer cell function, reduced salivary IgA, and increased susceptibility to upper respiratory tract infection (URTI). Marathoners and triathletes have measurably higher URTI rates in the week following race events than the general population.
Spirulina's immune-modulating polysaccharides (calcium-spirulan, immulina) and direct effects on NK-cell function appear to offset some of this exercise-induced immune suppression. Trials have shown:
- Preserved or enhanced NK-cell activity in the post-exercise window
- Reduced incidence of URTI in athletes during heavy training periods (effect size is modest but consistent)
- Preserved salivary IgA levels post-exercise
For competitive athletes whose training calendar is disrupted by repeated URTI episodes, the research suggests Spirulina supplementation at 4-6 g/day during heavy training blocks may be useful. Alongside vitamin D supplementation (in athletes with documented deficiency) and adequate sleep, it is one of the more evidence-supported nutritional approaches for protecting training availability.
Dosing Patterns Described for Athletes
Dosing patterns described in, or derived from, the trial literature:
- Standard endurance-training dose: 4-6 g/day, divided into two doses (morning and pre-training), with the trials pointing to at least 4 weeks of consistent intake before a performance benefit appears
- High-volume training block dose: 6-8 g/day during peak training weeks, returning to 4 g/day during recovery and taper periods
- Pre-race protocol: the 4-6 g/day dose is typically maintained through race week; an acute "loading dose" on race day is not supported by the research — the benefit is from sustained supplementation, not acute ingestion
- Post-race recovery: 4 g/day is typically continued during the recovery week; some athletes increase to 6-8 g/day for the 3-5 days after a marathon or ultra to support recovery and immune defense
- Female athletes with marginal iron status: 5-10 g/day combined with 100 mg vitamin C with each Spirulina dose, with serum ferritin commonly rechecked every 8-12 weeks
- Power and strength athletes: lower priority — Spirulina's benefits are most pronounced in oxidative-metabolism-limited exercise; sprinters, weightlifters, and pure-strength athletes derive less benefit per gram
Tablets, capsules, and powder are all used. Powder mixed into a smoothie or yogurt is the most cost-effective. The taste is grassy and earthy — some athletes find it off-putting in plain water but acceptable in juice or with fruit. Tablets and capsules eliminate the taste issue at higher cost per gram.
Comparison with Other Ergogenic Aids
Spirulina occupies a different role in the ergogenic supplement landscape than the better-known performance enhancers:
- vs Caffeine: Caffeine produces larger acute performance gains (5-15% in many endurance protocols) with a single pre-exercise dose, and has stronger evidence overall. Spirulina's effects emerge over weeks of supplementation, not from a single dose. The two act on different timescales — caffeine as an acute race-day effect, Spirulina as a chronic training adaptation.
- vs Creatine: Creatine is the most evidence-supported supplement for strength and high-intensity intermittent exercise. Spirulina's benefits are in oxidative endurance, a different domain. No interaction between the two has been described.
- vs Beta-alanine: Beta-alanine increases muscle carnosine and buffering capacity for high-intensity exercise lasting 1-4 minutes. Different domain than Spirulina.
- vs Beetroot (nitrate): Beetroot juice increases nitric oxide bioavailability and reduces oxygen cost of exercise. Mechanistically distinct but functionally overlapping with Spirulina's endothelial-function effects. No conflict between the two has been described.
- vs Tart cherry: Tart cherry juice has the best evidence for reduced post-exercise inflammation and muscle damage in the 24-72 hour recovery window. Mechanistically similar to Spirulina's antioxidant effects; the two are partial substitutes.
- vs Vitamin C and E megadosing: High-dose isolated antioxidant vitamins (vitamin C > 1 g/day, vitamin E > 400 IU/day) actually blunt training adaptations in some studies, by suppressing the beneficial ROS-signaling that drives mitochondrial biogenesis. Spirulina's polyphenolic antioxidants do not appear to produce this blunting effect, perhaps because the antioxidant action is distributed across many compounds at moderate doses rather than concentrated in a single high-dose intervention.
Cautions for Competitive Athletes
- WADA banned substance contamination — third-party sport-testing certification programs exist to screen supplements for banned substances. The Spirulina molecule itself is not banned, but supplement manufacturing facilities can produce cross-contamination with banned substances (anabolic steroids, stimulants, beta-2 agonists) that result in failed drug tests despite the absence of any deliberate doping.
- Heavy metal contamination — particularly concerning for female athletes of reproductive age and adolescent athletes. Products vary in whether they are tested for heavy metals.
- Microcystin contamination — the hepatotoxic risk affects all populations but is especially concerning for athletes whose hepatic function is already stressed by high training loads, NSAID use, or supplement polypharmacy.
- Gastrointestinal distress before competition — some athletes develop nausea or loose stools when starting Spirulina. Common sports-nutrition guidance is to establish tolerance several weeks before an important race and not to introduce a new supplement in the week before competition.
- Iron stacking caution — in athletes already taking high-dose iron supplements, Spirulina's iron adds to the total, which counts toward the tolerable upper intake level of 45 mg/day of iron.
- Phenylketonuria — absolute contraindication regardless of athletic context.
- Pregnancy in competitive athletes — therapeutic doses lack adequate safety data in pregnancy; only dietary amounts are outside that gap.
Key Research Papers
- Kalafati M et al. (2010). Ergogenic and antioxidant effects of Spirulina supplementation in humans. Medicine and Science in Sports and Exercise. — PubMed PMID: 20010119
- Lu HK et al. (2006). Preventative effects of Spirulina platensis on skeletal muscle damage under exercise-induced oxidative stress. European Journal of Applied Physiology. — PubMed PMID: 16944194
- Sandhu JS et al. Efficacy of Spirulina supplementation on isometric strength and isometric endurance of quadriceps in trained and untrained individuals: a comparative study. Ibnosina Journal of Medicine and Biomedical Sciences. — PubMed
- Brito AKDS et al. Effects of Spirulina platensis on the performance and recovery of athletes: a meta-analysis. Sports. — PubMed
- Hernandez-Lepe MA et al. Hypolipidemic effect of Arthrospira (Spirulina) maxima supplementation and exercise on dyslipidemic adults. Marine Drugs. — PubMed PMID: 31067674
- Calella P et al. Antioxidant, anti-inflammatory and immunomodulatory effects of Spirulina in exercise and sport: a systematic review. Frontiers in Nutrition. — PubMed PMID: 36590230
- Gurney T, Brouner J. Spirulina supplementation in athletes: an overview. Journal of Sport and Health Sciences. — PubMed
- Selmi C et al. The effects of Spirulina on anemia and immune function in senior citizens. Cellular and Molecular Immunology. — PubMed PMID: 21278762
- Park JH et al. Effect of dietary Spirulina supplementation on physical performance in untrained subjects. Korean Journal of Family Medicine. — PubMed
- Powers SK, Jackson MJ. Exercise-induced oxidative stress: cellular mechanisms and impact on muscle force production. Physiological Reviews. — PubMed
- Nieman DC. Exercise immunology: nutritional countermeasures. Canadian Journal of Applied Physiology. — PubMed PMID: 11897882
- Margaritis I et al. Antioxidant supplementation and athletic performance: a critical review. Free Radical Biology and Medicine. — PubMed