⚠ Evidence warning: Clinical trials or other evidence do not support the claim that serine supplements can improve age-related memory complaints and high homocysteine or methylation problems. This page keeps it as a report of what people, websites or other media say.
Serine — Benefits Deep Dive
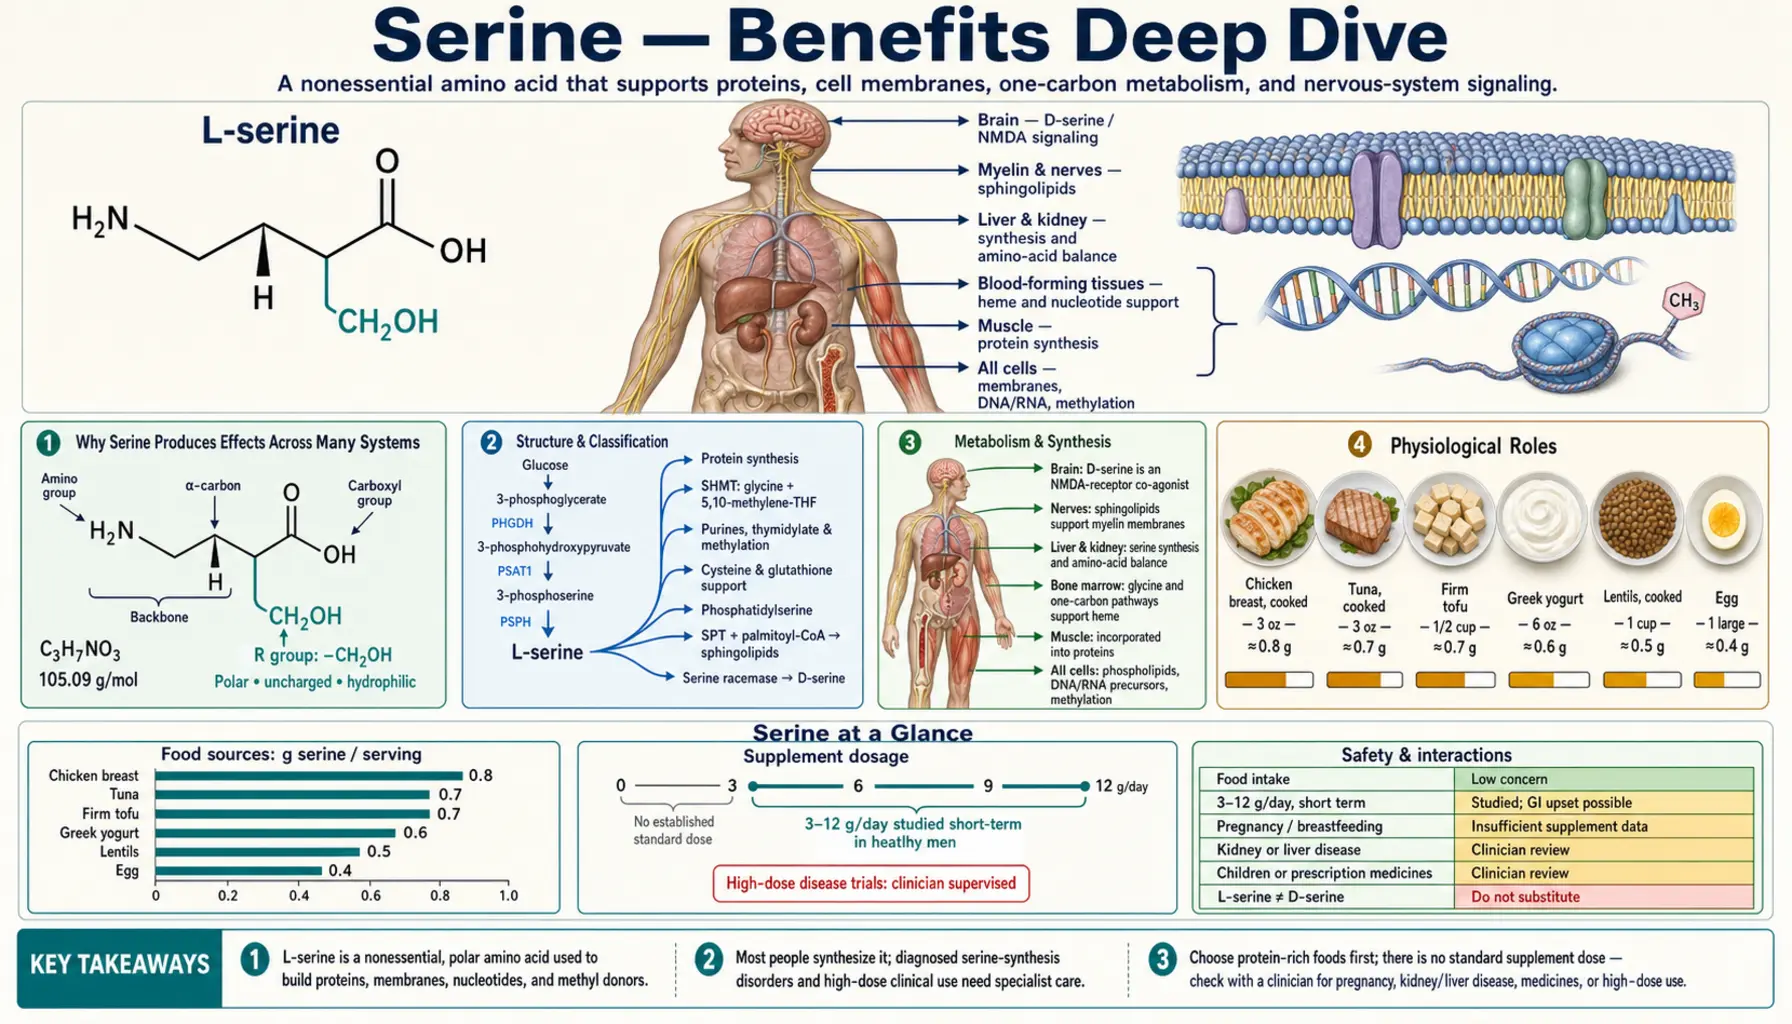
Serine is the rare non-essential amino acid that occurs in two distinct chiral forms each with a separate, important biological function. L-serine is the protein-coding form, the substrate that feeds phosphatidylserine for cell membranes and brain function, sphingolipid biosynthesis for the myelin sheath, and one-carbon metabolism for DNA synthesis and methylation. D-serine is the dextrorotary enantiomer, synthesized in the brain by serine racemase, that serves as the principal endogenous co-agonist at N-methyl-D-aspartate (NMDA) glutamate receptors and is the focus of two decades of schizophrenia and cognitive aging research. Four deep-dive pages below explore the conditions where serine produces the largest clinical effect — age-related cognitive decline (via phosphatidylserine), schizophrenia and N-methyl-D-aspartate-mediated cognition (via D-serine), the methylation network and cancer metabolism (via the SHMT serine-glycine interconversion), and the rare hereditary sensory and autonomic neuropathy type 1 (HSAN1) plus the broader sphingolipid pathology that links serine to metabolic syndrome and myelin disease.
Deep-Dive Articles
Phosphatidylserine & the Aging Brain
Phosphatidylserine (PS) as the major inner-leaflet anionic phospholipid of every cell membrane, concentrated at 13-15% of total phospholipid in brain tissue. The Crook 1991 and 1992 trials in age-associated memory impairment, the switch from bovine cortex to soy-derived PS in the mid-1990s driven by bovine spongiform encephalopathy (BSE, “mad cow disease”), the 2003 U.S. Food and Drug Administration (FDA) qualified health claim for cognitive dysfunction, the Hirayama and Manor pediatric attention-deficit/hyperactivity disorder (ADHD) trials, and the cortisol-modulation effect that supports PS use in athletic overtraining.
Read the deep dive →D-Serine & N-Methyl-D-Aspartate Receptors
The discovery that mammals make D-amino acids after all — D-serine is synthesized by serine racemase in glutamatergic neurons and serves as the principal endogenous co-agonist at the glycine site of synaptic N-methyl-D-aspartate receptors. The Tsai 1998 and Heresco-Levy 2005 schizophrenia trials, sarcosine and D-amino acid oxidase (DAO) inhibitor pipelines, the Sasabe 2007 finding that D-serine accumulates pathologically in amyotrophic lateral sclerosis (ALS) spinal cord, and the bidirectional therapeutic implications.
Read the deep dive →Glycine Source & One-Carbon Metabolism
Serine hydroxymethyltransferase (SHMT) cleaves L-serine to glycine plus 5,10-methylenetetrahydrofolate (5,10-methylene-THF), the activated one-carbon donor that feeds DNA synthesis, the methionine cycle, and S-adenosylmethionine-dependent methylation throughout the body. Cytosolic SHMT1 vs mitochondrial SHMT2, why serine is the quantitatively dominant one-carbon source, the glycine cleavage system, methylenetetrahydrofolate reductase (MTHFR) variants, and the serine-and-glycine restriction strategy in cancer metabolism (Maddocks 2013, 2017).
Read the deep dive →Sphingolipid Synthesis & HSAN1
Serine palmitoyltransferase (SPT) is the rate-limiting step of all sphingolipid biosynthesis: L-serine + palmitoyl-CoA → 3-ketodihydrosphingosine. Mutations in SPTLC1 cause Hereditary Sensory and Autonomic Neuropathy type 1 (HSAN1) by changing SPT substrate specificity so the enzyme misincorporates L-alanine in place of L-serine, producing toxic 1-deoxysphingolipids. Oral L-serine 400 mg/kg/day partially corrects the defect — one of the cleanest examples of disease-modifying amino acid therapy. In a randomized trial of 18 patients (Fridman 2019), one year of L-serine improved the neuropathy score by 1.5 points relative to placebo (p = 0.03), and toxic deoxysphinganine fell 59% versus an 11% rise on placebo, with no serious side effects.
Read the deep dive →Table of Contents
- Deep-Dive Articles
- Why Serine Produces Effects Across Many Systems
- Research Papers: Phosphatidylserine & Brain
- Research Papers: D-Serine & N-Methyl-D-Aspartate
- Research Papers: SHMT, Glycine, & One-Carbon Metabolism
- Research Papers: SPT, Sphingolipids, & HSAN1
- Research Papers: Cross-Cutting (Metabolism, Status, Safety)
- External Authoritative Resources
- Connections
- Featured Videos
Why Serine Produces Effects Across Many Systems
Most amino acids occupy a single primary functional role — either as a building block of protein (typical case), as a precursor to a small set of neurotransmitters and signaling molecules (tryptophan, tyrosine, glutamate), or as a regulator of a specific metabolic process (arginine for nitric oxide, methionine for methylation). Serine is unusual because it operates as a central hub for at least four fundamentally distinct biochemical networks, each of which produces a different category of clinical effect.
- Phosphatidylserine and membrane biology — one serine molecule is consumed per phosphatidylserine (PS) molecule made. PS is the dominant anionic phospholipid of the inner membrane leaflet, concentrated in brain at 13-15% of total phospholipid. This is the mechanism behind age-related cognitive decline, the Crook 1991 trials, and the U.S. Food and Drug Administration qualified health claim for PS in cognitive dysfunction.
- D-serine and N-methyl-D-aspartate receptor signaling — the L-serine to D-serine racemization by serine racemase produces the endogenous co-agonist at the glycine site of synaptic N-methyl-D-aspartate receptors. This is the mechanism behind the schizophrenia trials of D-serine, the broader N-methyl-D-aspartate hypofunction hypothesis, and the bidirectional implications for amyotrophic lateral sclerosis where D-serine accumulates pathologically.
- SHMT and one-carbon metabolism — serine hydroxymethyltransferase converts serine to glycine plus 5,10-methylenetetrahydrofolate (5,10-methylene-THF), the activated one-carbon donor that feeds DNA synthesis and the methionine cycle. Serine is the quantitatively dominant one-carbon source (~50-90% of total flux). This is the mechanism behind the methylation network, methylenetetrahydrofolate reductase variants and homocysteine, and the cancer-metabolism strategy of serine and glycine restriction.
- SPT and sphingolipid biosynthesis — serine palmitoyltransferase condenses L-serine with palmitoyl-CoA to launch the entire sphingolipid biosynthesis network. This is the mechanism behind myelin biology, the rare hereditary neuropathy HSAN1 (one of the cleanest examples of disease-modifying amino acid therapy), and the broader role of ceramides in insulin resistance and metabolic syndrome.
The unifying thread across these four networks is that each requires serine as substrate, and each is sensitive to serine supply at the relevant rate-limiting enzyme. Serine availability therefore acts as a master regulator of cellular function in a way that few other small molecules can match. The clinical implication is that adequate serine intake supports a broad range of physiological functions simultaneously, and that targeted serine supplementation can address specific deficits across very different organ systems — from age-related cognitive complaints (where PS substrate provision is the goal), to elevated homocysteine and methylation cycle dysfunction (where SHMT substrate provision is the goal), to the rare HSAN1 neuropathy (where direct competition with toxic substrate misincorporation is the goal).
The complication is that the same molecule can produce opposite effects in different settings. In schizophrenia, the N-methyl-D-aspartate hypofunction hypothesis predicts benefit from boosting N-methyl-D-aspartate signaling, and earlier small trials of D-serine added to antipsychotics were encouraging; the largest add-on trial (Weiser 2012; 195 patients, D-serine 2 g/day for 16 weeks) found no difference from placebo for negative symptoms (11.4% vs 14.8% improvement) or cognition (6.8% vs 6.1%), and its authors noted a relatively large placebo response and lower achieved doses than in earlier trials. In amyotrophic lateral sclerosis, where pathological D-serine accumulation is linked to motor neuron excitotoxicity, raising D-serine is a theoretical concern; L-serine itself, at 0.5 to 15 g twice daily, appeared safe in a 20-patient phase I trial in amyotrophic lateral sclerosis (Bradley 2018), in which two patients withdrew because of gastrointestinal side effects. The same logic applies to cancer biology, where the cell-proliferation support that serine provides is therapeutically desirable in most settings but undesirable in actively growing tumors. The four deep-dives address these nuances within each domain.
Research Papers: Phosphatidylserine & Brain
- Crook TH et al. (1991), foundational age-associated memory impairment trial with bovine-cortex PS — PubMed: Crook 1991 age-associated memory impairment
- Crook T et al. (1992), PS in early Alzheimer's-type cognitive impairment — PubMed: Crook 1992
- Cenacchi T et al. (1993), Italian multicenter PS trial in cognitive decline — PubMed: Cenacchi 1993
- FDA (2003), qualified health claim for PS and reduced risk of cognitive dysfunction — PubMed: FDA qualified claim
- Hirayama S et al. (2014), randomized soy-PS trial in pediatric ADHD — PubMed: Hirayama ADHD
- Manor I et al. (2012), PS-Omega3 conjugate in pediatric ADHD — PubMed: Manor PS-Omega3
- Monteleone P et al. (1990), PS modulation of neuroendocrine stress response — PubMed: Monteleone cortisol
- Starks MA et al. (2008), PS for exercise-induced cortisol — PubMed: Starks exercise
- Vance JE (2008), PS and PE in mammalian cells review — PubMed: Vance PS/PE review
- Kim HY et al. (2014), PS in the brain — metabolism and function — PubMed: Kim PS brain review
Research Papers: D-Serine & N-Methyl-D-Aspartate
- Hashimoto A et al. (1992), discovery of free D-serine in rat brain — PubMed: Hashimoto 1992
- Wolosker H, Blackshaw S, Snyder SH (1999), serine racemase as the brain's D-serine factory — PubMed: Wolosker 1999
- Mothet JP et al. (2000), D-serine as endogenous NMDA co-agonist — PubMed: Mothet 2000
- Tsai G et al. (1998), D-serine added to antipsychotics in schizophrenia — PubMed: Tsai 1998
- Heresco-Levy U et al. (2005), high-dose D-serine in schizophrenia — PubMed: Heresco-Levy 2005
- Sasabe J et al. (2007), D-serine accumulation in ALS spinal cord — PubMed: Sasabe ALS
- Lane HY et al. (2013), sodium benzoate DAO inhibitor in schizophrenia — PubMed: Lane benzoate JAMA
- Tsai G, Lane HY et al. (2004), sarcosine in schizophrenia — PubMed: Sarcosine schizophrenia
- Mitchell J et al. (2010), DAO loss-of-function in familial ALS — PubMed: DAO familial ALS
- Coyle JT, Balu DT (2018), The role of serine racemase in the pathophysiology of brain disorders. Advances in Pharmacology — PubMed PMID: 29413527
- Weiser M, Heresco-Levy U, Davidson M, et al. (2012), A multicenter, add-on randomized controlled trial of low-dose D-serine for negative and cognitive symptoms of schizophrenia. Journal of Clinical Psychiatry — PubMed PMID: 22795211
- Bradley WG, Miller RX, Levine TD, et al. (2018), Studies of environmental risk factors in amyotrophic lateral sclerosis (ALS) and a phase I clinical trial of L-serine. Neurotoxicity Research — PubMed PMID: 28527102
Research Papers: SHMT, Glycine, & One-Carbon Metabolism
- Ducker GS, Rabinowitz JD (2017), one-carbon metabolism in health and disease — PubMed: Ducker review
- Maddocks ODK et al. (2013), serine starvation and p53 in cancer — PubMed: Maddocks 2013
- Maddocks ODK et al. (2017), serine-glycine restriction in tumor models — PubMed: Maddocks 2017
- Locasale JW (2013), serine and glycine cancer metabolism review — PubMed: Locasale review
- Meléndez-Hevia E et al. (2009), glycine and collagen biosynthesis weak link — PubMed: Meléndez-Hevia
- Tibbetts AS, Appling DR (2010), compartmentalization of one-carbon metabolism — PubMed: Tibbetts review
- Frosst P et al. (1995), MTHFR C677T discovery — PubMed: Frosst MTHFR
- Stover PJ (2009), one-carbon metabolism-genome interactions — PubMed: Stover folate genome
- Bailey LB et al. (2015), folate biomarkers for development — PubMed: Folate biomarkers
Research Papers: SPT, Sphingolipids, & HSAN1
- Dawkins JL et al. (2001), SPTLC1 mutations in HSAN1 — PubMed: Dawkins HSAN1
- Penno A et al. (2010), neurotoxic deoxysphingolipids mechanism — PubMed: Penno deoxy-SL
- Garofalo K et al. (2011), oral L-serine reduces deoxysphingolipids — PubMed: Garofalo JCI
- Fridman V, Suriyanarayanan S, Novak P, et al. (2019), Randomized trial of L-serine in patients with hereditary sensory and autonomic neuropathy type 1. Neurology — PubMed PMID: 30626650
- Hannun YA, Obeid LM (2018), sphingolipids in physiology and disease — PubMed: Hannun review
- Breslow DK, Weissman JS (2010), ORMDL sphingolipid homeostasis — PubMed: Breslow ORMDL
- Summers SA, Chaurasia B, Holland WL (2019), ceramides as metabolic messengers — PubMed: Ceramides metabolism
- Moffatt MF et al. (2007), ORMDL3 childhood asthma GWAS — PubMed: ORMDL3 asthma
- Eichler FS et al. (2009), SPT1 overexpression rescues HSAN1 phenotype — PubMed: Eichler HSAN1 rescue
- Chaurasia B, Summers SA (2015), ceramides as lipotoxic metabolic inducers — PubMed: Chaurasia ceramides
Research Papers: Cross-Cutting (Metabolism, Status, Safety)
- de Koning TJ, Snell K, Duran M, et al. (2003), L-serine in disease and development. Biochemical Journal — PubMed PMID: 12534373
- Tabatabaie L et al. (2010), L-serine biosynthesis disorders review — PubMed: Serine biosynthesis disorders
- Yang M, Vousden KH (2016), serine and one-carbon metabolism in cancer — PubMed: Serine cancer review
- Possemato R et al. (2011), PHGDH amplification in breast cancer — PubMed: PHGDH breast cancer
- Selvy PE et al. (2011), phospholipase D and PS biology review — PubMed: Phospholipase D review
- Ron D, Walter P (2007), unfolded protein response and lipid metabolism — PubMed: UPR lipid metabolism
- de Koning TJ, Klomp LW (2004), Serine-deficiency syndromes (treatment of serine-synthesis defects with L-serine). Current Opinion in Neurology — PubMed PMID: 15021249
- Newman AC, Maddocks ODK (2017), one-carbon metabolism in cancer review — PubMed: Newman one-carbon cancer
- Pacheco-Alvarez D, Solórzano-Vargas RS, Del Río AL (2002), Biotin in metabolism and its relationship to human disease (general biotin review). Archives of Medical Research — PubMed PMID: 12459313
- Wolosker H et al. (2008), D-amino acids in brain comprehensive review — PubMed: D-amino acids review
External Authoritative Resources
- Linus Pauling Institute — Other Nutrients (Amino Acids) — comprehensive scientific micronutrient and amino acid summaries
- StatPearls — Biochemistry, Amino Acid Synthesis and Degradation (open-access medical reference)
- GeneReviews — Hereditary Sensory and Autonomic Neuropathy Type IA (HSAN1) (NCBI Bookshelf)
- MedlinePlus Genetics — Hereditary sensory neuropathy type IA (HSAN1)
- GeneReviews — Serine Deficiency Disorders
- PubMed — All research on serine (40,000+ papers)
- PubMed — All research on phosphatidylserine
- PubMed — D-serine and the brain
Connections
- All Amino Acids
- Serine (Main Page)
- Serine for Phosphatidylserine & Brain
- Serine for D-Serine & N-Methyl-D-Aspartate
- Serine as Glycine Source (SHMT)
- Serine in Sphingolipid Synthesis (SPT)
- Glycine
- Methionine
- Cysteine
- Threonine
- Glutamic Acid
- Alanine
- Vitamin B6 (SHMT & SPT Cofactor)
- Vitamin B12
- Folate
- Homocysteine
- Alzheimer's Disease
- Amyotrophic Lateral Sclerosis
- Schizophrenia
- Insulin Resistance
- Bone Broth (Glycine Source)
- Omega-3 Fatty Acids
- History
- Sources