⚠ Evidence warning: Clinical trials or other evidence do not support the claims that beta-alanine adds to the effects of caffeine and of nitrate, and gives vegetarians larger performance gains. This page keeps it as a report of what people, websites or other media say.
Beta-Alanine for Endurance and High-Intensity Exercise
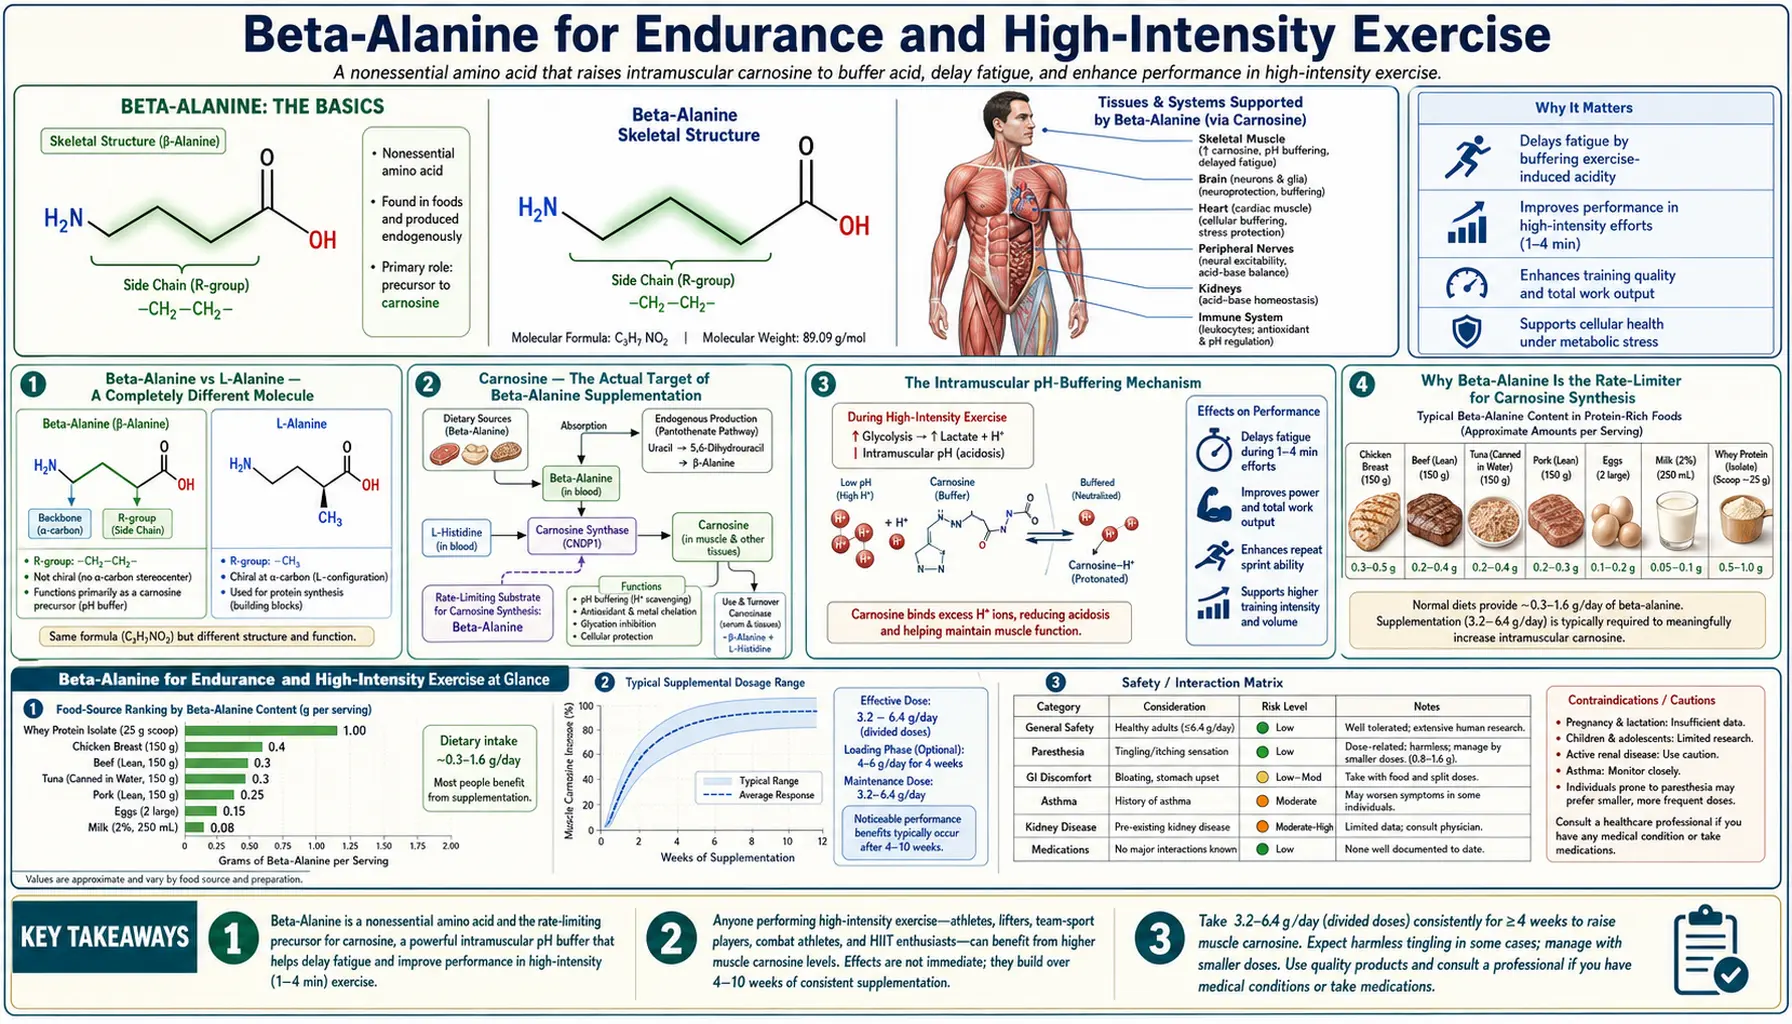
Beta-alanine is one of the most important misconceptions in sports nutrition: despite the shared name, it is biochemically and pharmacologically nothing like L-alanine. Beta-alanine (3-aminopropanoic acid) is a structural isomer in which the amino group sits on the beta-carbon rather than the alpha-carbon, and crucially, it is not incorporated into proteins. Its sole established role in human physiology is as the rate-limiting precursor for carnosine (beta-alanyl-L-histidine), a dipeptide present at high concentrations in skeletal muscle, where it functions as an intramuscular pH buffer during anaerobic exercise. Beta-alanine supplementation raises muscle carnosine concentration: by 58.8% at 4 weeks and 80.1% at 10 weeks in one trial (Hill 2007), and by 23-39% across three muscles after 5-6 weeks at 4.8 g/day in another (Baguet 2009) — an effect achievable through no dietary route except concentrated meat consumption, and not achievable at all through L-alanine supplementation. About two decades of well-controlled randomized trials have established that beta-alanine produces a small but reliable improvement in exercise capacity for efforts in the 1-4 minute range (where intramuscular pH drops are most performance-limiting), and the Australian Institute of Sport lists it among its six Group A performance supplements. The 2015 position stand of the International Society of Sports Nutrition (ISSN) also supports it for exercise performance.
Table of Contents
- Beta-Alanine vs L-Alanine — A Completely Different Molecule
- Carnosine — The Actual Target of Beta-Alanine Supplementation
- The Intramuscular pH-Buffering Mechanism
- Why Beta-Alanine Is the Rate-Limiter for Carnosine Synthesis
- Dose and Loading Protocols (Harris / Hoffman)
- The Paraesthesia ("Tingle") Effect
- Documented Exercise-Capacity Effects
- Non-Responders and the Vegetarian Effect
- Other Putative Roles of Carnosine (Beyond Exercise)
- Stacking with Other Sports Supplements
- Cautions
- Key Research Papers
- Connections
- Featured Videos
Beta-Alanine vs L-Alanine — A Completely Different Molecule
The most important conceptual point about beta-alanine is that it is, despite the shared name, a fundamentally different molecule from L-alanine and serves a non-overlapping biological role. The two share only the molecular formula (C3H7NO2) and a stoichiometric similarity. Their biochemistry, transport, metabolism, and clinical applications are entirely separate.
The structural distinction is the position of the amino group relative to the carboxylic acid:
- L-alanine (alpha-alanine): The amino group is attached to the alpha-carbon — the carbon adjacent to the carboxylic acid group. This is the standard amino acid configuration shared by all 20 proteinogenic amino acids. L-alanine is incorporated into proteins via the standard ribosomal machinery and participates in transamination reactions catalyzed by alanine aminotransferase (ALT).
- Beta-alanine (3-aminopropanoic acid): The amino group is attached to the beta-carbon — one carbon further from the carboxylic acid. This single-bond difference makes beta-alanine non-proteinogenic. There is no transfer RNA that codes for beta-alanine, no aminoacyl-tRNA synthetase that recognizes it, and no ribosome that incorporates it into protein. It is also not a substrate for alanine aminotransferase (the enzyme is specific for the alpha-amino-acid stereochemistry).
The two amino acids are also transported differently. L-alanine uses the System A and System ASC sodium-dependent transporters (SNAT1, SNAT2, ASCT1, ASCT2). Beta-alanine uses a completely different transporter, the taurine/gamma-aminobutyric acid (GABA) transporter family (TauT/SLC6A6), which it shares with taurine and gamma-aminobutyric acid. This is the biochemical reason that taurine and beta-alanine compete for uptake at the muscle cell membrane and at the blood-brain barrier — a fact relevant when stacking these two supplements.
The only metabolic connection between L-alanine and beta-alanine in human physiology is that beta-alanine can be slowly produced from L-aspartate through aspartate decarboxylation in the liver, and from cytosine and uracil (pyrimidine bases) through their catabolic pathway. These endogenous sources produce only modest amounts of beta-alanine — nowhere near enough to saturate muscle carnosine synthesis, which is why oral supplementation produces such striking carnosine increases.
Carnosine — The Actual Target of Beta-Alanine Supplementation
Carnosine (beta-alanyl-L-histidine) is a dipeptide of beta-alanine and L-histidine connected by a standard peptide bond. It was discovered in 1900 by the Russian biochemist V.S. Gulewitsch in beef extract (hence the name "carnosine" from carnis, Latin for flesh). It is present at high concentrations — 5-25 mmol/kg dry muscle — in skeletal muscle of all vertebrates, with the highest concentrations in the fast-twitch (Type II) fibers that are most dependent on anaerobic glycolysis.
The functional importance of carnosine in muscle was established through the work of Roger Harris and his colleagues in the early 2000s. Three properties make carnosine uniquely well-suited for its buffering role:
- Optimal pKa — the imidazole side chain of the histidine moiety has a pKa of approximately 6.83, very close to physiological intramuscular pH during heavy exercise (which can drop from 7.0 at rest to 6.4 during maximal anaerobic exertion). This is the ideal pKa range for a chemical buffer — the dipeptide accepts protons (H+) most efficiently exactly in the pH window where buffering matters most. Free histidine has a similar pKa but is less effective because of its non-restricted geometry.
- High intramuscular concentration — carnosine accumulates at concentrations of 10-30 mM in trained sprinters and elite anaerobic athletes. The ISSN position stand reports that estimates of its share of muscle buffering run from as much as 40% in animals to as low as 7% in humans, and Abe's 2000 review says non-bicarbonate buffering in vertebrate muscle is mainly supported by histidine groups in proteins, free histidine in some fish, and dipeptides such as carnosine. By comparison, intramuscular phosphate buffers are typically 5-10 mM and intramuscular protein buffers contribute another 20-30 mM equivalent capacity.
- Cytosolic localization — carnosine is freely dissolved in the muscle cell cytosol rather than confined to organelles. This puts it precisely where the protons accumulate during anaerobic glycolysis (Robergs and colleagues' 2004 review, which drew published replies, attributes these protons to the breakdown of adenosine triphosphate during intense exercise, and reports that lactate production retards rather than causes acidosis). The cytosol is the active site of buffering, not the mitochondria or the sarcoplasmic reticulum.
Carnosine concentrations vary substantially between individuals, fiber types, and species. Sprinters have higher concentrations than endurance athletes. Type IIx fibers (fastest fast-twitch) have higher concentrations than Type I (slow oxidative). In a study of 149 people (Everaert 2011), men had 36%, 28% and 82% higher concentrations than women in three leg muscles, and vegetarians had 26% lower carnosine in the gastrocnemius than omnivores (meat being the dietary source of preformed beta-alanine). Genetic polymorphisms in carnosine synthetase are proposed to explain some of the remaining individual variability; the same study found muscle carnosine unrelated to the gene for carnosinase (the degradative enzyme, CNDP1) or to plasma carnosinase activity.
Muscle carnosine falls slowly after supplementation stops: Baguet 2009 measured a decline of 2-4% per week, with a return to baseline within 9 weeks at group level (15 weeks in high responders, 6 weeks in low responders). Loading is slow as well: in a 24-week trial, carnosine was still climbing well after week 4 (+11.37 mmol/kg dry muscle at week 4, +21.20 at week 20). This relatively slow turnover is why beta-alanine is dosed continuously rather than only on training/competition days, and why the timing of beta-alanine intake within a day matters very little.
The Intramuscular pH-Buffering Mechanism
To understand why intramuscular carnosine matters for exercise performance, it helps to understand the proton-accumulation problem during anaerobic exercise.
During high-intensity exercise that exceeds the rate at which oxygen can be supplied and used by the mitochondria, muscle cells rely on anaerobic glycolysis — the conversion of glucose to lactate — for adenosine triphosphate (ATP) production. Each glucose molecule that goes through anaerobic glycolysis yields 2 adenosine triphosphate plus 2 lactate. The lactate is not the cause of the "burn" or the fatigue — it is the protons (H+), which the 2004 Robergs review attributes to adenosine triphosphate breakdown rather than to lactate formation. The lactate is shipped to the liver via the Cori cycle and is, if anything, a useful aerobic fuel for the heart and slow-twitch fibers. The protons are what drop intramuscular pH from 7.0 at rest toward 6.4 at exhaustion.
The pH drop has multiple performance-limiting effects:
- Inhibition of phosphofructokinase-1 (PFK-1) — the rate-limiting glycolytic enzyme is allosterically inhibited by low pH. As pH drops, glycolytic flux slows, adenosine triphosphate production falls, and the muscle cannot sustain force.
- Reduced calcium sensitivity of the contractile apparatus — troponin-C's calcium-binding affinity is pH-dependent. Lower pH reduces the calcium binding and thereby reduces the activation of the actin-myosin cross-bridge cycle for a given calcium release from the sarcoplasmic reticulum.
- Direct inhibition of the calcium-release channel (RyR1) — ryanodine receptor 1 activity is also pH-sensitive. Low cytosolic pH reduces the magnitude of each calcium release event from the sarcoplasmic reticulum.
- Increased excitatory neurotransmitter release from peripheral pain afferents — the "burn" itself acts as a central nervous system-mediated negative feedback signal that reduces voluntary effort.
Carnosine's role is to absorb protons before they can reach the concentrations that trigger these performance-limiting effects. Each mole of carnosine's imidazole group can buffer one mole of H+, so the total buffering capacity scales linearly with intramuscular concentration. Raising muscle carnosine (by +58.8% at 4 weeks and +80.1% at 10 weeks in Hill 2007) raises the carnosine contribution to total intramuscular buffering capacity in proportion, which is described as enough to delay the onset of severe acidosis by tens of seconds in the 1-4 minute exercise window.
Why Beta-Alanine Is the Rate-Limiter for Carnosine Synthesis
Carnosine is synthesized intramuscularly by carnosine synthase (ATPGD1, also known as CARNS1), which catalyzes the adenosine triphosphate-dependent condensation of free beta-alanine and free L-histidine. The reaction is:
beta-alanine + L-histidine + adenosine triphosphate → carnosine + adenosine diphosphate + phosphate
Older accounts gave adenosine monophosphate and pyrophosphate as the products. Drozak and colleagues (2010) purified the enzyme and found carnosine forming with a matching amount of adenosine diphosphate instead, which places carnosine synthase in the ATP-grasp family of enzymes.
The reaction depends on both substrates being available at sufficient concentration. The key insight from the Harris 2006 and Hill 2007 studies is that L-histidine is normally present in muscle at saturating concentrations, while beta-alanine is normally present at sub-saturating concentrations. This makes beta-alanine the rate-limiting substrate. Oral histidine loading does not raise muscle carnosine. Oral beta-alanine loading does.
The mathematical implication is straightforward: increasing the bioavailable beta-alanine pool increases the substrate for carnosine synthase, which proportionally increases the muscle carnosine concentration over the weeks-long timescale that the muscle pool requires to equilibrate. The kinetics of the equilibration follow a roughly exponential approach to a new steady-state ceiling. Hill 2007 showed that 4 weeks of loading at 4.8 g/day raised muscle carnosine by 58%, and 10 weeks of loading at the same dose raised it by 80% the additional 6 weeks added much less benefit than the first 4 weeks, consistent with an asymptotic approach to a ceiling.
The diet contains some preformed carnosine and anserine (the methylated carnosine analog found at higher concentrations in poultry and fish), and much of it does not last. Gardner and colleagues (1991) recovered up to 14% of ingested intact carnosine in urine, showing that it crosses the intestine, and then found rapid breakdown after absorption by the blood enzyme carnosinase (CN1, CNDP1). The net effect is that almost all the beta-alanine that reaches muscle for carnosine synthesis must come from supplemental free beta-alanine, not from dietary carnosine. This is why concentrated meat consumption raises muscle carnosine only modestly compared to direct beta-alanine supplementation.
The longest trial found in this review ran 24 weeks: 25 active men were assigned to 6.4 g a day of sustained-release beta-alanine or placebo (Saunders 2017). Carnosine rose +11.37 mmol/kg dry muscle by week 4 and about +20 by weeks 20-24, with wide differences between people (maximal rises from +17.13 to +41.32), none on placebo, and a high-intensity cycling test improved. The authors say this spread suggests something other than beta-alanine supply also has a major influence on muscle carnosine.
Dose and Loading Protocols (Harris / Hoffman)
The usual beta-alanine loading protocols trace to the Harris 2006 study and to later trials such as Hoffman 2008, a training trial in college football players. The 2015 ISSN position stand by Trexler and colleagues states that daily supplementation with 4 to 6 g for at least 2 to 4 weeks has been shown to improve exercise performance, and that tingling can be attenuated by divided lower doses (1.6 g) or a sustained-release formula. The protocols described are:
- Loading dose: 4-6 g/day for 4-12 weeks, divided into smaller doses of 0.8-1.6 g taken every 3-4 hours throughout the day. The division into smaller doses is important not for efficacy but to minimize paraesthesia (see below). The 4-week endpoint represents the minimum required to reach approximately 50-60% of the steady-state ceiling; 12 weeks reaches approximately 80-90%.
- Maintenance dose: Stegen 2014 tested 0.4, 0.8 and 1.2 g/day for six weeks after loading; about 1.2 g/day kept muscle carnosine 30%-50% above baseline. Figures up to 2.4 g/day are also quoted, a dose that trial did not test. Discontinuation results in a slow washout, described under Carnosine above (2-4% per week in Baguet 2009).
- Sustained-release formulations: Beta-alanine is available in slow-release tablets (Decombaz 2012) that release the dose over 1-2 hours rather than producing the peak plasma concentration of immediate-release. Decombaz tested 1.6 g in 11 healthy adults: peak blood level was 82 versus 248 µmol/L, and side effects could not be told apart from placebo. Once-daily dosing of the full 4-6 g without the tingle effect is also claimed; that trial did not test it.
- Timing within a day: Does not matter for efficacy. Carnosine is built up over weeks; the time-of-day a given dose is taken has no impact on the steady-state concentration. Athletes may prefer to take beta-alanine away from training to avoid paraesthesia during sessions, or with food to slow absorption and reduce paraesthesia.
- Cycling on and off: Not biochemically necessary. The longest trial found in this review ran 24 weeks at 6.4 g/day; the 2019 risk assessment listed under Cautions reports paraesthesia as the only side effect. Some athletes choose to cycle off during the off-season to reduce supplement cost, with the understanding that they will need 4-12 weeks of reloading before the next competitive season.
Doses above 6 g/day are described as not producing proportionally greater muscle carnosine elevation. Blancquaert and colleagues (2016; mouse work plus recombinant mouse and human enzymes) report that only 3-6% of ingested beta-alanine is used for carnosine synthesis, and that the rest can be routed to oxidation by two transaminase enzymes in liver and kidney, 4-aminobutyrate-2-oxoglutarate transaminase and alanine-glyoxylate transaminase. Doses above 10 g/day are described as wasted and dramatically increase paraesthesia without performance benefit.
The Paraesthesia ("Tingle") Effect
The most distinctive feature of beta-alanine supplementation is the harmless paraesthesia effect that occurs within 15-30 minutes of taking a bolus dose larger than approximately 800 mg. It is described variously as "pins and needles," "skin tingles," or a "tropical itch" sensation, typically felt in the face, neck, hands, and torso. It subsides within 30-60 minutes and produces no lasting effect. Athletes initially mistake it for an allergic reaction or a stimulant effect; it is neither.
The mechanism is the activation of the MrgprD receptor (Mas-related G-protein-coupled receptor member D), a recently discovered class of GPCR expressed on a subset of cutaneous C-fiber sensory neurons. Beta-alanine is one of the only known endogenous ligands of MrgprD, and high plasma beta-alanine concentrations transiently depolarize MrgprD-expressing neurons, producing the tingle sensation. The same MrgprD pathway is also involved in itch sensation, which is why some users describe the sensation as itchy rather than tingly.
Practical management of paraesthesia includes:
- Divided dosing — the original Harris/Hoffman 0.8-1.6 g doses every 3-4 hours stays below the paraesthesia threshold for most users.
- Slow-release tablets — the Decombaz formulation flattens the peak plasma concentration enough to eliminate paraesthesia even at 1.6 g per dose.
- Taking with food — gastric emptying delays absorption and reduces peak plasma concentration; a 1.6 g dose taken with a meal produces minimal paraesthesia for most users.
- Habituation — the paraesthesia intensity decreases over weeks of consistent use as users either upregulate MrgprD desensitization or simply adapt to the sensation.
The paraesthesia is harmless and reversible. No serious adverse events have been linked to it in long-term studies. The clinical significance is essentially zero — it is a marker of the dose having been absorbed, not a sign of toxicity. Users who find it intolerable can use slow-release formulations to eliminate it entirely.
Documented Exercise-Capacity Effects
The Saunders 2017 British Journal of Sports Medicine meta-analysis (40 studies, 70 individual exercise outcomes, n=1,461 participants) is the largest aggregation of beta-alanine exercise trials. It reports a small overall effect size of 0.18 (95% confidence interval 0.08 to 0.28). Within efforts of 0.5-10 minutes, tests to exhaustion improved (effect size 0.50, confidence interval 0.25 to 0.75), while timed performance did not clearly improve (0.11, confidence interval -0.20 to 0.42). Taking sodium bicarbonate as well gave the largest effect against placebo (0.43, confidence interval 0.22 to 0.64). With the earlier Hobson 2012 meta-analysis (15 manuscripts, 360 participants), the picture by duration is:
- All exercise measures: Hobson 2012 reports a median 2.85% improvement (-0.37 to 10.49%) after a median total of 179 g of beta-alanine.
- Exercise duration of 1 to 4 minutes (the "sweet spot"): Hobson 2012 found exercise of 60-240 seconds improved (P=0.001), and the ISSN position stand reports more pronounced effects in tasks of 1 to 4 minutes. A figure of +4-5% is also quoted; it is in neither meta-analysis abstract. This corresponds to events like 400m and 800m running, 200m freestyle swimming, 1000m rowing, and 30-second to 4-minute Wingate or mixed circuit-type efforts.
- Exercise duration below 30 seconds: No meaningful benefit; Hobson 2012 found none under 60 seconds (P=0.312). Very short maximal efforts are powered by adenosine triphosphate-PCr (creatine phosphate) rather than glycolysis, so intramuscular pH does not drop enough to be performance-limiting. Creatine, which extends this energy system, is the supplement usually discussed for this duration range.
- Exercise duration above 10 minutes: Smaller benefit. Duration significantly moderated effects in Saunders 2017 (p=0.004). Hobson 2012 found exercise over 240 seconds also improved (P=0.046), and the ISSN position stand reports modest benefit on time to exhaustion in tests over 4 minutes, with more research needed beyond 25 minutes. Long-duration exercise is oxidative rather than glycolytic, so the intramuscular pH does not drop into the carnosine-buffering range. Beta-alanine is described as having minimal value for marathon running, long-distance cycling, or other endurance events without high-intensity surges.
- Exercise involving repeated sprint bouts: Beta-alanine improves performance in the later sprints of a series. Single sprints are described as showing no benefit, and repeated sprints with short rest intervals (mixed circuit training, soccer, hockey, basketball) as showing benefit because the cumulative pH drop is in the carnosine-buffering range. Saunders 2017 found no moderating effect of intermittent versus continuous exercise (p=0.436).
Real-world translation in elite athletes is modest but meaningful. A 4% improvement in a 2000m rowing time would mean about 14 seconds faster on an elite 6:00 erg time — a margin described as the difference between qualifying for and missing the Olympic team. For recreational athletes, the practical benefit is "a few more reps" or "a few more seconds" in the late stages of glycolytically demanding sessions. Beta-alanine is not a transformative supplement — it does not make slow athletes fast — but it produces a small reliable edge in the specific exercise domain where carnosine buffering matters.
Non-Responders and the Vegetarian Effect
Muscle carnosine rises differ widely between people: Baguet 2009 divided subjects into high responders (+55%) and low responders (+15%). Several mechanisms have been proposed:
- Serum carnosinase (CNDP1) polymorphisms — high-activity CNDP1 variants hydrolyze plasma carnosine and beta-alanyl-histidine intermediates more rapidly, reducing the carnosine pool available for muscle uptake. The CNDP1 CTG haplotype is said to be associated with reduced beta-alanine efficacy. Everaert 2011 (149 people) found muscle carnosine not related to the CNDP1 gene or to plasma carnosinase activity; it did not test the response to supplements.
- Baseline carnosine concentration — subjects who start with high baseline carnosine show smaller percentage increases because they are closer to the carnosine synthase saturation ceiling. Trained sprinters and meat-eaters often show smaller increases than untrained subjects and vegetarians.
- Carnosine synthase variants — rare polymorphisms in ATPGD1/CARNS1 produce lower enzyme activity and reduce the carnosine response to beta-alanine loading.
Conversely, vegetarians are the population most likely to show large beta-alanine responses. Because vegetarian diets contain essentially no preformed carnosine and minimal beta-alanine (which is concentrated in muscle meat), vegetarians typically have lower baseline muscle carnosine than omnivores (26% lower in the gastrocnemius in Everaert 2011). Beta-alanine supplementation in vegetarian athletes therefore produces larger relative increases and larger associated performance improvements. The 2007 Derave trial in trained sprinters showed substantial benefit. The ISSN position stand says vegetarians have greater increases in carnosine concentrations than carnivores; a figure of approximately 50% larger responses is also quoted.
Other Putative Roles of Carnosine (Beyond Exercise)
Beyond its established role as a muscle pH buffer, carnosine has additional biological properties that are areas of active research, though clinical translations remain incomplete:
- Anti-glycation — carnosine is one of the most potent endogenous inhibitors of advanced glycation end-product (AGE) formation. It binds to reactive carbonyl groups (methylglyoxal, glyoxal, 4-hydroxynonenal) and quenches them before they can crosslink with proteins. This has generated interest in carnosine as an anti-aging compound and as a complementary therapy in diabetic complications, though clinical evidence remains preliminary.
- Antioxidant activity — carnosine scavenges singlet oxygen, hydroxyl radicals, and peroxyl radicals. It chelates copper, iron, and zinc, all of which can drive Fenton-type radical chemistry. The functional significance of this in vivo is debated.
- Heavy metal chelation — carnosine binds copper, zinc, and other transition metals. Some research has explored zinc-L-carnosine as a gastric mucosal protectant (used clinically in Japan as polaprezinc for gastric ulcer healing).
- Neuroprotection — carnosine and its methylated relative homocarnosine are present in the brain (homocarnosine in cerebrospinal fluid (CSF) reflects gamma-aminobutyric acid metabolism). Some preclinical evidence suggests neuroprotection in models of cerebral ischemia, but clinical trials in stroke have been small and inconclusive.
- Wound healing — topical and oral carnosine have been studied in diabetic ulcer healing. Effects are modest but the safety profile is excellent.
For the well-established role of beta-alanine in exercise specifically, the evidence base is strong. The other potential applications remain promising but unproven at clinical scale. These findings do not show beta-alanine to be an anti-aging or neuroprotection supplement — the demonstrated use case is exercise capacity in glycolytically demanding sport.
Stacking with Other Sports Supplements
Beta-alanine is one of the evidence-supported sports supplements alongside creatine monohydrate, caffeine, sodium bicarbonate, and nitrates (beetroot); all five are on the Australian Institute of Sport's Group A list, which also includes glycerol. These five have independent mechanisms and are often combined:
- Beta-alanine + creatine monohydrate — the most popular stack, with strong rationale. Creatine extends the adenosine triphosphate-PCr system that powers very short maximal efforts (5-20 seconds); beta-alanine extends the glycolytic system that powers slightly longer efforts (30 seconds to 4 minutes). The two work in adjacent energy systems and produce additive benefits in mixed-domain circuit sessions. The 2006 Stout trial (51 untrained men, 28 days) found physical working capacity at the neuromuscular fatigue threshold higher than placebo with beta-alanine and with the combination, but reported "no additive or unique effects" of creatine versus beta-alanine alone.
- Beta-alanine + sodium bicarbonate — both work as pH buffers but at different sites. Beta-alanine (via carnosine) buffers intramuscularly; sodium bicarbonate (via bicarbonate) buffers extracellularly in the blood, drawing protons out of muscle into circulation via the proton-lactate cotransporter. The two have additive effects, but sodium bicarbonate carries a high gastrointestinal side-effect burden (acute diarrhea) that limits its real-world use.
- Beta-alanine + caffeine — non-overlapping mechanisms (caffeine is central-nervous-system focused on perceived exertion and motor unit recruitment). Stacking is safe and produces additive effects on high-intensity exercise.
- Beta-alanine + beetroot/nitrate — nitrate works by improving mitochondrial efficiency and lowering the oxygen cost of submaximal exercise. Different mechanism from beta-alanine's pH buffering. The two are additive in middle-distance events.
- Beta-alanine + taurine — competes for the same TauT transporter. Some authors have suggested that chronic high-dose beta-alanine could deplete muscle taurine, but the magnitude appears small and clinically inconsequential. Taurine supplementation alongside beta-alanine is said to answer any theoretical depletion concern.
For more on the broader sports nutrition landscape, see our pages on Leucine (for muscle protein synthesis) and Glutamine (for recovery and gut barrier function).
Cautions
- Paraesthesia is harmless but distracting — the ISSN position stand reports that divided lower doses (1.6 g) or a sustained-release formula attenuate the tingle.
- No documented long-term safety issues — the longest trial found in this review ran 24 weeks at 6.4 g/day. The ISSN position stand says beta-alanine "currently appears to be safe in healthy populations at recommended doses".
- 2019 risk assessment — a systematic review of 101 human and 50 animal studies found tingling (paraesthesia) the only reported side effect (odds ratio 8.9 versus placebo), with dropout rates similar to placebo. Blood alanine aminotransferase (ALT), a liver enzyme, rose slightly (effect size 0.274), with average values staying well within the normal range. It found no main effect on muscle taurine or histidine in people.
- Theoretical taurine depletion — via TauT competition. Magnitude is described as small. Taurine 1-2 g/day alongside is mentioned for vegetarian endurance athletes, who may also have lower baseline taurine; the 2019 risk assessment found no main effect on muscle taurine in people, and Hill 2007 found none at 10 weeks.
- Pregnancy and lactation — no studies have evaluated beta-alanine safety in pregnancy. There is no safety data for pregnant or breastfeeding women.
- Children and adolescents — pediatric safety data for athletes under 18 are lacking. The principal use case (high-intensity competitive sport) is adult-focused anyway.
- Banned substance concerns — beta-alanine is not on the WADA Prohibited List and is allowed in all competitive sports. It is a naturally occurring molecule and produces no positive doping test.
- Distinction from L-alanine for the consumer — the two are easily confused when shopping. L-alanine supplements (typically marketed for blood sugar or general amino acid support) do not raise muscle carnosine and do not produce the exercise capacity benefits of beta-alanine. A beta-alanine label specifically says "beta-alanine" (sometimes written as "β-alanine").
- Stack interactions with stimulants — many pre-workout products combine beta-alanine, caffeine, and other stimulants. The combined paraesthesia plus stimulant arousal can feel intense and is sometimes mistakenly attributed to one ingredient alone. Knowing which sensation comes from which ingredient helps users titrate the stack to their tolerance.
Key Research Papers
- Harris RC, Tallon MJ, Dunnett M, et al. (2006). The absorption of orally supplied beta-alanine and its effect on muscle carnosine synthesis in human vastus lateralis. Amino Acids 30(3):279-289. — DOI: 10.1007/s00726-006-0299-9. — doi:10.1007/s00726-006-0299-9
- Hill CA, Harris RC, Kim HJ, et al. (2007). Influence of beta-alanine supplementation on skeletal muscle carnosine concentrations and high intensity cycling capacity. Amino Acids 32(2):225-233. — DOI: 10.1007/s00726-006-0364-4. — doi:10.1007/s00726-006-0364-4
- Hoffman J, Ratamess NA, Faigenbaum AD, et al. (2008). Short-duration beta-alanine supplementation increases training volume and reduces subjective feelings of fatigue in college football players. Nutrition Research 28(1):31-35. — DOI: 10.1016/j.nutres.2007.11.004. — doi:10.1016/j.nutres.2007.11.004
- Trexler ET, Smith-Ryan AE, Stout JR, et al. (2015). International Society of Sports Nutrition position stand: Beta-alanine. Journal of the International Society of Sports Nutrition 12:30. — DOI: 10.1186/s12970-015-0090-y. — doi:10.1186/s12970-015-0090-y
- Saunders B, Elliott-Sale K, Artioli GG, et al. (2017). Beta-alanine supplementation to improve exercise capacity and performance: a systematic review and meta-analysis. British Journal of Sports Medicine 51(8):658-669. — DOI: 10.1136/bjsports-2016-096396. — doi:10.1136/bjsports-2016-096396
- Boldyrev AA, Aldini G, Derave W (2013). Physiology and pathophysiology of carnosine. Physiological Reviews 93(4):1803-1845. — DOI: 10.1152/physrev.00039.2012. — doi:10.1152/physrev.00039.2012
- Derave W, Ozdemir MS, Harris RC, et al. (2007). Beta-Alanine supplementation augments muscle carnosine content and attenuates fatigue during repeated isokinetic contraction bouts in trained sprinters. Journal of Applied Physiology 103(5):1736-1743. — DOI: 10.1152/japplphysiol.00397.2007. — doi:10.1152/japplphysiol.00397.2007
- Stout JR, Cramer JT, Mielke M, et al. (2006). Effects of twenty-eight days of beta-alanine and creatine monohydrate supplementation on the physical working capacity at neuromuscular fatigue threshold. Journal of Strength & Conditioning Research 20(4):928-931. — DOI: 10.1519/R-19655.1. — PubMed PMID: 17194255
- Decombaz J, Beaumont M, Vuichoud J, et al. (2012). Effect of slow-release beta-alanine tablets on absorption kinetics and paresthesia. Amino Acids 43(1):67-76. — DOI: 10.1007/s00726-011-1169-7. — doi:10.1007/s00726-011-1169-7
- Sale C, Saunders B, Harris RC (2010). Effect of beta-alanine supplementation on muscle carnosine concentrations and exercise performance. Amino Acids 39(2):321-333. — DOI: 10.1007/s00726-009-0443-4. — doi:10.1007/s00726-009-0443-4
- Liu Q, Sikand P, Ma C, et al. (2012). Mechanisms of itch evoked by beta-alanine. Journal of Neuroscience 32(42):14532-14537. — DOI: 10.1523/JNEUROSCI.3509-12.2012. — doi:10.1523/JNEUROSCI.3509-12.2012
- Stegen S, Bex T, Vervaet C, et al. (2014). Beta-alanine dose for maintaining moderately elevated muscle carnosine levels. Medicine & Science in Sports & Exercise 46(7):1426-1432. — DOI: 10.1249/MSS.0000000000000248. — doi:10.1249/MSS.0000000000000248
- Hobson RM, Saunders B, Ball G, Harris RC, Sale C (2012). Effects of beta-alanine supplementation on exercise performance: a meta-analysis. Amino Acids 43(1):25-37. — PubMed PMID: 22270875
- Saunders B, de Salles Painelli V, de Oliveira LF, et al. (2017). Twenty-four weeks of beta-alanine supplementation on carnosine content, related genes, and exercise. Medicine & Science in Sports & Exercise 49(5):896-906. — PubMed PMID: 28157726
- Baguet A, Reyngoudt H, Pottier A, et al. (2009). Carnosine loading and washout in human skeletal muscles. Journal of Applied Physiology 106(3):837-842. — PubMed PMID: 19131472
- Everaert I, Mooyaart A, Baguet A, et al. (2011). Vegetarianism, female gender and increasing age, but not CNDP1 genotype, are associated with reduced muscle carnosine levels in humans. Amino Acids 40(4):1221-1229. — PubMed PMID: 20865290
- Dolan E, Swinton PA, Painelli VS, et al. (2019). A systematic risk assessment and meta-analysis on the use of oral beta-alanine supplementation. Advances in Nutrition 10(3):452-463. — PubMed PMID: 30980076
- Drozak J, Veiga-da-Cunha M, Vertommen D, Stroobant V, Van Schaftingen E (2010). Molecular identification of carnosine synthase as ATP-grasp domain-containing protein 1 (ATPGD1). Journal of Biological Chemistry 285(13):9346-9356. — PubMed PMID: 20097752
- Blancquaert L, Baba SP, Kwiatkowski S, et al. (2016). Carnosine and anserine homeostasis in skeletal muscle and heart is controlled by beta-alanine transamination. Journal of Physiology 594(17):4849-4863. — PubMed PMID: 27062388
- Gardner ML, Illingworth KM, Kelleher J, Wood D (1991). Intestinal absorption of the intact peptide carnosine in man, and comparison with intestinal permeability to lactulose. Journal of Physiology 439:411-422. — PubMed PMID: 1910085
- Robergs RA, Ghiasvand F, Parker D (2004). Biochemistry of exercise-induced metabolic acidosis. American Journal of Physiology — Regulatory, Integrative and Comparative Physiology 287(3):R502-R516. — PubMed PMID: 15308499
- Abe H (2000). Role of histidine-related compounds as intracellular proton buffering constituents in vertebrate muscle. Biochemistry (Moscow) 65(7):757-765. — PubMed PMID: 10951092
PubMed Topic Searches
Connections
- All Amino Acids
- Alanine Overview
- Alanine Benefits Hub
- Alanine for Gluconeogenesis & Blood Sugar
- Alanine for Immune Function
- Alanine for Liver Function (Alanine Aminotransferase)
- Histidine (Carnosine Partner)
- Taurine (TauT Transporter Sibling)
- Leucine
- Isoleucine
- Valine
- Glutamine
- Creatine Monohydrate
- Athletic Performance
- Beef (Dietary Carnosine)
- Chicken (Dietary Carnosine)
- Fatigue
- Beta-Alanine — the standalone page for the carnosine-precursor amino acid compared throughout this article.
- History
- Sources