Valine for Muscle Protein Synthesis
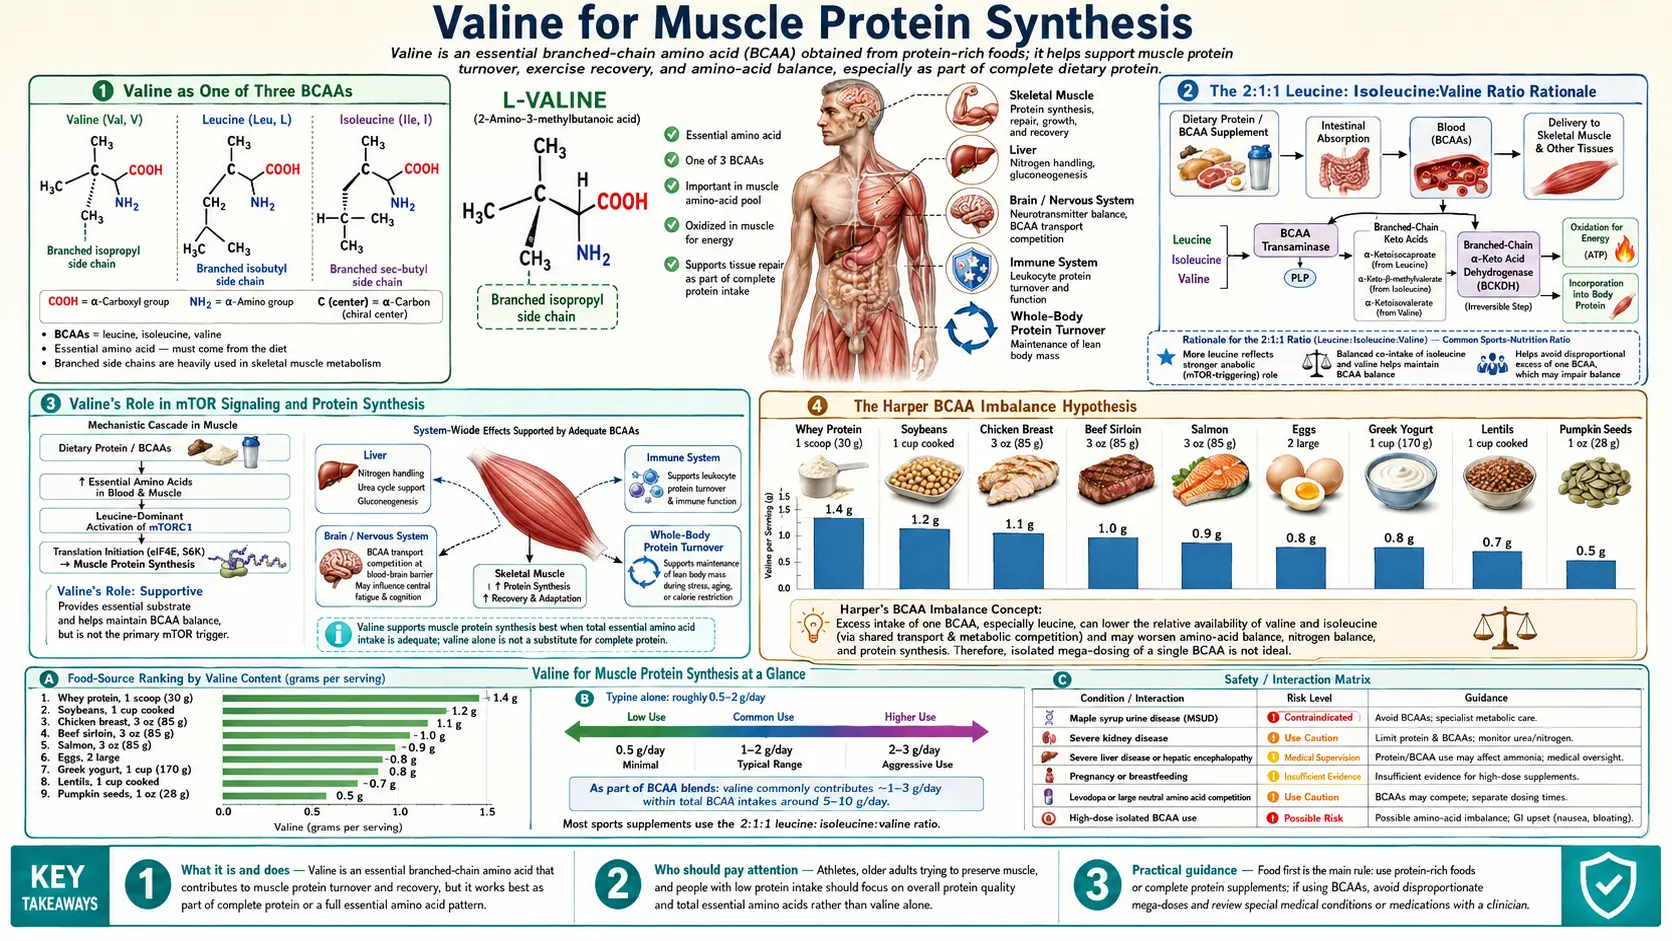
Valine is one of the three branched-chain amino acids (BCAAs), the structural and signaling trio that constitutes roughly one-third of skeletal muscle protein. The conventional 2:1:1 leucine:isoleucine:valine ratio in branched-chain amino acid (BCAA) supplements is not arbitrary — it mirrors the relative abundance of these three amino acids in muscle tissue itself. Yet valine is the most frequently shortchanged member of the trio, especially in leucine-only "anabolic activator" supplements that promise mechanistic target of rapamycin (mTOR) signaling but ignore the substrate-availability problem. The Harper imbalance hypothesis, formulated by Alfred Harper in the 1960s, demonstrated that excess leucine alone can paradoxically depress growth in animal models by competitively depleting plasma valine and isoleucine. This page explains why balanced branched-chain amino acid intake matters more than leucine maximalism, how valine specifically contributes to mechanistic target of rapamycin activation, and the clinical contexts where the 2:1:1 ratio has been validated.
Table of Contents
- Valine as One of Three Branched-Chain Amino Acids
- The 2:1:1 Leucine:Isoleucine:Valine Ratio Rationale
- Valine's Role in Mechanistic Target of Rapamycin Signaling and Protein Synthesis
- The Harper Branched-Chain Amino Acid Imbalance Hypothesis
- What Leucine-Only Supplements Leave Out
- Valine in Muscle Tissue Composition
- Post-Exercise Recovery and Soreness Reduction
- Sarcopenia and the Aging Muscle
- Clinical Applications: Cachexia, Trauma, Intensive Care Unit
- Practical Dosing Strategies
- Key Research Papers
- Connections
- Featured Videos
Valine as One of Three Branched-Chain Amino Acids
The three branched-chain amino acids — leucine, isoleucine, and valine — share a defining structural feature: a non-linear, branched aliphatic side chain that distinguishes them from the other 17 proteinogenic amino acids. The branching is what gives them both their name and their distinctive metabolic behavior. Unlike most amino acids, which are processed first by the liver upon absorption, branched-chain amino acids largely bypass first-pass hepatic metabolism and are instead taken up directly by skeletal muscle, where the enzymes that initiate their catabolism (branched-chain aminotransferase, BCAT2, and the rate-limiting branched-chain alpha-ketoacid dehydrogenase, BCKAD complex) are most abundant.
This direct muscular routing is what makes branched-chain amino acids especially relevant to athletic and clinical contexts where rapid amino acid availability at the muscle is required. Within the trio, each amino acid plays a partially distinct role: leucine is the principal anabolic signaling amino acid, the most potent activator of the mechanistic target of rapamycin (mTOR) pathway; isoleucine contributes to glucose uptake by muscle through both insulin-dependent and insulin-independent pathways; valine serves both as a substrate for protein synthesis and as a metabolic feedstock for the TCA cycle via succinyl-CoA. All three are essential amino acids — the human body cannot synthesize them de novo and must obtain them through diet or supplementation.
Yet the three are not interchangeable. The supplement industry has historically over-emphasized leucine because of its singular role in mechanistic target of rapamycin activation, leading to a series of products marketed as "leucine boosters" or "anabolic activators" that contain little or no valine and isoleucine. The biochemistry of muscle protein synthesis, however, requires substrate from all three plus the other six essential amino acids — mechanistic target of rapamycin activation without substrate availability is like turning on a factory's power without delivering the raw materials. This substrate-vs-signal distinction is central to understanding why balanced branched-chain amino acid intake matters more than leucine maximalism.
The 2:1:1 Leucine:Isoleucine:Valine Ratio Rationale
The standard branched-chain amino acid supplement ratio of 2:1:1 (leucine:isoleucine:valine) is not arbitrary; it reflects the approximate ratio of these three amino acids in human skeletal muscle protein. When muscle is broken down (analyzed by hydrolysis and amino acid quantification), the branched-chain amino acid content typically falls in the range of 20-22% leucine, 10-12% isoleucine, and 10-12% valine relative to total amino acid content. The 2:1:1 ratio therefore approximately mirrors the substrate composition of the tissue being built.
Some product lines have promoted alternative ratios — 4:1:1, 8:1:1, even 10:1:1 — on the theory that more leucine is always better for mechanistic target of rapamycin activation. The main argument made against these higher ratios is biochemical. The downside of high-leucine ratios is precisely the Harper imbalance problem: by saturating the BCAT2 enzyme with leucine, the metabolism of valine and isoleucine is competitively inhibited, and plasma levels of both drop. The mechanistic target of rapamycin pathway may be activated, but the actual substrates for new muscle protein become limiting.
A practical implication: when comparing branched-chain amino acid supplements, the ratio is just as important as the total dose. A 5-gram serving at 2:1:1 (2.5g leucine, 1.25g isoleucine, 1.25g valine) is more bioavailable as muscle substrate than a 5-gram serving at 4:1:1 (3.33g leucine, 0.83g isoleucine, 0.83g valine), despite the lower absolute leucine content in the former. Whole food protein (whey, casein, egg, meat) provides branched-chain amino acids in approximately the 2:1:1 ratio naturally, which is one of several reasons that food-source protein consistently outperforms isolated branched-chain amino acid supplements in muscle synthesis trials.
Valine's Role in Mechanistic Target of Rapamycin Signaling and Protein Synthesis
The mechanistic target of rapamycin pathway is the central regulator of cellular anabolism. Mechanistic target of rapamycin exists in two complexes: mTORC1 (rapamycin-sensitive, the canonical anabolic kinase) and mTORC2 (less rapamycin-sensitive, involved in cytoskeletal regulation and Akt signaling). Muscle protein synthesis is driven primarily through mTORC1, which when active phosphorylates two key downstream targets: 4E-BP1 (releasing eIF4E to initiate cap-dependent mRNA translation) and p70S6K (activating the ribosomal S6 kinase to increase translation throughput).
Leucine is the dominant amino acid signal to mTORC1. Leucine is sensed by Sestrin2, a cytoplasmic leucine sensor that, when leucine-loaded, releases its inhibition of GATOR2, which in turn permits Rag GTPases to recruit mTORC1 to the lysosomal surface where it can be activated by Rheb. This is a beautifully specific molecular sensing mechanism, and it is why leucine alone can transiently activate the pathway. However, sustained mTORC1 activity and actual protein synthesis require additional inputs: insulin signaling, mechanical load (exercise), energy status (low AMP/ATP ratio), and — critically — substrate availability of all the amino acids required to build the protein being synthesized.
Valine's role here is principally as substrate. When mTORC1 fires and ribosomes begin translating muscle protein mRNAs, the elongation step requires charged tRNAs for every codon, including valine codons (GUU, GUC, GUA, GUG — four of the 64 possible codons in the genetic code, used wherever a valine residue appears in the protein sequence). If valine-tRNA pools are depleted, elongation stalls at valine codons, and the ribosome cannot complete the protein. The classic experimental demonstration of this is the General Amino Acid Control (GAAC) response: when any one essential amino acid runs low, uncharged tRNA accumulates, which activates the GCN2 kinase, which phosphorylates eIF2alpha, which globally suppresses cap-dependent translation. The net result is that valine deficiency — even with abundant leucine and mechanistic target of rapamycin signaling — can dramatically reduce overall protein synthesis output.
Valine has also been proposed to play a second role in the mechanistic target of rapamycin pathway, at the leucine sensor Sestrin2. In the 2016 test-tube experiments that identified Sestrin2 as a leucine sensor (Wolfson and colleagues), of 18 amino acids tested at 300 µM each, only those most similar to leucine — methionine, isoleucine and valine — had any effect on the Sestrin2–GATOR2 interaction. The crystal-structure study published alongside it (Saxton and colleagues) found that small amino acids such as alanine or valine fail to make favourable contacts in Sestrin2's leucine pocket, so that only leucine and the structurally similar isoleucine and methionine interact appreciably. Any direct effect of valine on Sestrin2 is therefore weak. The idea that mixed branched-chain amino acid supplements produce a longer and more sustained mechanistic target of rapamycin activation than equivalent leucine-only doses, because the trio keeps Sestrin2 in a "loaded" state for longer, is a hypothesis that these studies did not test.
The Harper Branched-Chain Amino Acid Imbalance Hypothesis
The most consequential discovery in branched-chain amino acid nutrition was made by Alfred Harper at the University of Wisconsin in a series of experiments in the 1950s and 1960s. Harper was studying amino acid imbalance — specifically, why adding a single amino acid to an otherwise marginally adequate diet sometimes produced growth depression in rats rather than the expected improvement. His seminal observation was that excess dietary leucine caused growth depression that could be reversed by adding valine and isoleucine. This finding became known as the "branched-chain amino acid antagonism" or "Harper imbalance hypothesis."
The mechanism Harper proposed, later confirmed at the molecular level, is competitive: all three branched-chain amino acids share the same transamination enzyme (branched-chain aminotransferase, BCAT) and the same rate-limiting dehydrogenase complex (BCKAD). When dietary leucine is in large excess, it competitively saturates these enzymes, accelerating its own catabolism and incidentally accelerating the catabolism of any valine and isoleucine present. The net effect is that excess leucine literally depletes the body's pools of valine and isoleucine, creating a functional deficiency of two essential amino acids even when total nitrogen intake is adequate.
This is biochemically counterintuitive but practically important. The Harper effect has been replicated in multiple species (rat, pig, chicken, human) and across multiple endpoints (growth rate, plasma amino acid concentrations, muscle protein synthesis rates, hepatic protein turnover). In the contemporary human literature, the most thoroughly documented manifestation is in patients with chronic kidney disease on low-protein diets supplemented with keto-analogs of leucine — these patients exhibit reproducible drops in plasma valine and isoleucine and require explicit valine and isoleucine supplementation to maintain balance.
The Harper hypothesis also explains a longstanding observation in protein quality scoring: the "limiting amino acid" concept. In any given protein source, the amino acid present in lowest amount relative to requirement sets the upper limit on how much of that protein can actually be used for synthesis. The other amino acids, even if present in abundance, are degraded for energy rather than incorporated into new tissue. Valine is rarely the limiting amino acid in animal proteins, but in some plant proteins (particularly maize) it can become co-limiting alongside lysine, which is why traditional cuisines that pair maize with legumes (Mexican beans and corn, for example) produce a more complete amino acid profile than either food alone.
What Leucine-Only Supplements Leave Out
Despite four decades of accumulated evidence supporting balanced branched-chain amino acid intake, the supplement market continues to feature leucine-only and high-leucine-ratio products marketed for muscle building. The rationale presented to consumers focuses on mechanistic target of rapamycin activation: "leucine is the only amino acid that directly activates mechanistic target of rapamycin, so just take leucine." This framing is technically true about the signaling step but ignores the substrate-availability step.
The practical consequence of leucine-only supplementation in humans has been examined in several controlled trials. A 2016 study by Moberg and colleagues in American Journal of Physiology — Cell Physiology compared the muscle's protein-building signal (mTORC1 signalling, measured in muscle biopsies) in eight trained volunteers who took placebo, leucine alone, full branched-chain amino acids (leucine + isoleucine + valine) or essential amino acids (EAAs, all nine, including the branched-chain amino acids) during four sessions of resistance exercise. The result: 90 minutes into recovery, the activity of the signalling enzyme S6 kinase 1 ranked placebo < leucine < branched-chain amino acids < EAAs, with a ninefold increase in the EAA trial. At 180 minutes, a second signalling marker (4E-BP1 phosphorylation) was still 40% higher with branched-chain amino acids or EAAs than with leucine alone. The authors concluded that EAAs appear to stimulate the start of protein building (translation initiation) more effectively than the other supplements, and that this effect is primarily attributable to the branched-chain amino acids. The study measured signalling, not muscle protein synthesis itself. In it, adding isoleucine and valine to leucine made the signal stronger.
Read together, these studies point the same way: balanced branched-chain amino acids produced a stronger signal than leucine alone, and complete essential-amino-acid sources a stronger one still. Whey protein, casein, egg protein, and high-quality meat or fish provide all nine essential amino acids in roughly the proportions needed for muscle synthesis, with the branched-chain amino acid fraction naturally at 2:1:1. Isolated branched-chain amino acids have been used mainly in narrow contexts: intra-workout sipping when whole protein would cause gastrointestinal distress; specific clinical situations like cirrhotic encephalopathy where the branched-chain amino acid-to-aromatic ratio matters; or supplementation of a marginally low-protein diet (e.g., some endurance-sport contexts during caloric restriction).
Valine in Muscle Tissue Composition
Quantitatively, valine constitutes approximately 5-6% of total amino acid residues in human skeletal muscle protein by weight. Across the major myofibrillar proteins:
- Myosin heavy chain (the most abundant muscle protein, the molecular motor of contraction): approximately 5.5% valine residues
- Actin (the second most abundant, the thin-filament protein): approximately 4.5% valine residues
- Titin (the largest known protein, the molecular spring providing passive tension): approximately 6.2% valine residues
- Troponin and tropomyosin (the regulatory proteins of the thin filament): approximately 5-7% valine residues
A 70-kg adult with approximately 28 kg of skeletal muscle (40% of body weight) carries roughly 5.6 kg of muscle protein, of which approximately 310 grams is valine residues. The daily turnover rate of muscle protein in a healthy adult is approximately 1-2%, meaning roughly 3-6 grams of valine residues are synthesized into muscle protein each day, and an approximately equal amount is liberated by proteolysis and either recycled (through reincorporation) or catabolized to succinyl-CoA via the BCKAD pathway.
This continuous turnover is the basis for the dietary valine requirement (~26 mg/kg/day per WHO, or ~1.8 g/day for a 70-kg adult). The requirement scales with muscle mass and with the rate of muscle remodeling: athletes engaged in heavy resistance training have approximately 50-100% higher muscle protein turnover and correspondingly higher valine (and overall branched-chain amino acid) requirements. Patients in catabolic states (sepsis, severe burn, post-surgical recovery, advanced cancer cachexia) may have 200-300% higher turnover, justifying targeted branched-chain amino acid supplementation as part of medical nutrition therapy.
Post-Exercise Recovery and Soreness Reduction
Resistance exercise produces microscopic damage to muscle fibers, particularly at the Z-disc and sarcomeric junctions, which is the structural basis for delayed-onset muscle soreness (DOMS) experienced 24-72 hours after a novel or intense training bout. The repair of this damage requires both mechanistic target of rapamycin signaling (to upregulate translation) and amino acid substrate (to provide the building blocks of new sarcomeric protein).
Branched-chain amino acid supplementation has been studied extensively for its effect on DOMS, with mixed but generally favorable results. A 2017 systematic review by Fouré and Bendahan analysed 11 studies of branched-chain amino acid supplementation after exercise-induced muscle damage and found high heterogeneity between their results. It concluded that branched-chain amino acids can be efficacious on markers of exercise-induced muscle damage as long as the damage was low-to-moderate, the daily intake was high (more than 200 mg per kg of body weight per day) and supplementation lasted a long time (more than 10 days), and that they were especially effective when taken before the damaging exercise.
Direct human data on branched-chain amino acids taken on their own come from a 2017 study by Jackman and colleagues in 10 resistance-trained young men. A drink of 5.6 g of branched-chain amino acids taken right after a workout raised muscle building (myofibrillar protein synthesis) over the next 4 hours by 22% compared with a placebo drink. Blood valine peaked about 144% above its starting level 30 minutes after the drink, and blood leucine and isoleucine about 300%. This was a single-session study that compared branched-chain amino acids with placebo, not with whole protein.
Within the branched-chain amino acid effect, valine's specific contribution is harder to dissect because human studies typically administer the trio together. Animal studies that have separated the branched-chain amino acids suggest that the soreness-reduction effect requires all three components, consistent with the substrate availability argument: damaged sarcomeres need to be rebuilt, and rebuilding requires balanced amino acid supply.
The International Society of Sports Nutrition (ISSN) position stand on protein and exercise (2017) states that a daily protein intake of 1.4-2.0 g per kg of body weight is sufficient for most exercising people, and that higher intakes (2.3-3.1 g/kg/day) may be needed to keep lean body mass in resistance-trained people during periods of calorie restriction. Its general figure per serving is 0.25 g of high-quality protein per kg of body weight, or an absolute dose of 20-40 g, ideally spread evenly every 3-4 hours across the day. It also notes that it is the essential amino acids that are required to stimulate muscle protein synthesis. This pattern provides ample branched-chain amino acid in the 2:1:1 ratio naturally and outperforms isolated branched-chain amino acid supplementation in nearly all controlled comparisons.
Sarcopenia and the Aging Muscle
Sarcopenia — the progressive age-related loss of muscle mass, strength, and function — is a major contributor to frailty, falls, and loss of independence in older adults. By age 80, the average person has lost approximately 30% of the muscle mass present at age 30. The mechanism is partly anabolic resistance: older muscle requires higher amino acid concentrations to achieve the same mechanistic target of rapamycin activation and protein synthesis response that younger muscle achieves at lower concentrations. The protein Recommended Dietary Allowance (RDA) of 0.8 g/kg/day, set decades ago for healthy adults, is now widely recognized as inadequate for older adults. The PROT-AGE Study Group (2013) gives an average daily intake of at least 1.0-1.2 g/kg/day for people over 65, at least 1.2 g/kg/day for those who are exercising or otherwise active, and 1.2-1.5 g/kg/day for most older adults with acute or chronic disease. The exception it names is older people with severe kidney disease (an estimated glomerular filtration rate, eGFR, under 30 mL/min/1.73 m²) who are not on dialysis: they may need to limit protein intake.
Within this elevated protein requirement, the branched-chain amino acid fraction — and valine specifically — remains in the same approximately 2:1:1 ratio as the muscle being preserved. Some clinical trials have tested whether leucine fortification (adding pure leucine to meals) can overcome anabolic resistance in older adults; results have been mixed, with some trials showing acute mechanistic target of rapamycin activation but limited long-term effects on muscle mass. As with younger adults, the limitation appears to be substrate, not signal: leucine fortification without proportional valine and isoleucine produces transient signaling without sustained synthesis.
The HMB (beta-hydroxy-beta-methylbutyrate) supplement — a leucine metabolite — has been studied as an alternative anabolic intervention in sarcopenia, particularly during periods of bed rest. Some evidence supports modest preservation of muscle mass during forced immobilization, though the effect is small compared to resistance exercise itself. For most older adults, the highest-yield interventions remain (1) progressive resistance training, (2) adequate total protein (PROT-AGE: at least 1.0-1.2 g/kg/day, and at least 1.2 g/kg/day for active people) in 25-40g doses per meal, and (3) sufficient vitamin D status — in that order. Isolated branched-chain amino acid or leucine supplementation is a distant fourth-line consideration.
Clinical Applications: Cachexia, Trauma, Intensive Care Unit
In severe catabolic illness — advanced cancer cachexia, major trauma, severe burns, sepsis with prolonged intensive care unit (ICU) stay — the body's muscle protein turnover dramatically accelerates, with proteolysis outpacing synthesis and producing rapid lean tissue loss. Branched-chain amino acid-enriched nutrition has been studied in each of these contexts:
- Cancer cachexia — trials of branched-chain amino acid-enriched oral nutrition supplements (typically 5-10 g branched-chain amino acid in 2:1:1 ratio added to standard supplements) have shown modest preservation of lean body mass and improvement in some quality-of-life measures, though effects on overall mortality have been inconsistent. The European Society for Clinical Nutrition and Metabolism (ESPEN) cancer cachexia guidelines do not strongly recommend branched-chain amino acid enrichment as standard but consider it reasonable in selected patients.
- Major trauma and post-surgical recovery — branched-chain amino acid-enriched parenteral nutrition was extensively studied in the 1980s and 1990s in surgical and trauma intensive care unit contexts. Most trials showed improved nitrogen balance with branched-chain amino acid enrichment but only marginal improvements in clinical outcomes, leading current intensive care unit nutrition guidelines (ASPEN/SCCM) to recommend standard protein dosing (1.2-2.0 g/kg/day) rather than branched-chain amino acid-specific formulations as the primary intervention.
- Severe burns — burn patients have among the highest documented protein requirements (up to 2.5-3 g/kg/day), and branched-chain amino acid-enriched formulas have been used historically. Modern burn nutrition emphasizes total energy and protein adequacy with high-biological-value whole protein sources over branched-chain amino acid-specific enrichment.
- Sepsis — the role of branched-chain amino acids in sepsis is more uncertain. Some animal studies suggest that elevated plasma branched-chain amino acids may exacerbate insulin resistance and worsen outcomes in sepsis; clinical guidelines do not recommend branched-chain amino acid-enriched feeding for sepsis routinely.
- Cirrhosis and hepatic encephalopathy — a 2026 Cochrane review of 18 randomised trials (934 adults, almost all with cirrhosis) found that the evidence suggests branched-chain amino acids reduce hepatic encephalopathy, the confusion and brain dysfunction caused by liver failure (risk ratio 0.79; low-certainty evidence). They may have little to no effect on death, but that evidence is very uncertain (risk ratio 0.89; very low-certainty evidence). Nausea and diarrhoea occurred in 12% of people taking branched-chain amino acids and 3% in the control groups, with very uncertain evidence on whether the supplements caused the difference. In an earlier one-year Italian trial of 174 people with advanced cirrhosis, oral branched-chain amino acid supplements reduced the combined rate of death or deterioration compared with lactoalbumin (a milk protein) and lowered hospital admissions, though long-term compliance was poor.
The thread running through these clinical contexts is the same as in athletic supplementation: substrate adequacy through total protein intake is more impactful than isolated branched-chain amino acid dosing, and balanced branched-chain amino acid outperforms isolated leucine when supplementation is used.
Practical Dosing Strategies
For most adults pursuing muscle health, the most effective valine "supplementation" is simply adequate dietary protein in the 2:1:1 branched-chain amino acid ratio that occurs naturally in animal proteins and many plant proteins. Figures reported for different groups:
- General adult requirement (sedentary): WHO 26 mg/kg/day of valine, approximately 1.8 g/day for a 70-kg adult, met by ~80 g of total protein from mixed sources.
- Recreationally active adult: 1.2-1.6 g/kg/day total protein, distributed across 4-5 meals of 25-40 g protein each, supplies approximately 3-5 g/day of valine without supplementation.
- Strength/hypertrophy athlete: the ISSN position stand gives 1.4-2.0 g/kg/day total protein as sufficient for most exercising people, and 2.3-3.1 g/kg/day to keep lean mass during calorie restriction. Isolated branched-chain amino acids are not needed to reach these totals; when they are used, 5-10 g of 2:1:1 branched-chain amino acids around training is the usual amount.
- Endurance athlete: 1.2-1.8 g/kg/day total protein. Branched-chain amino acids (5-10 g of 2:1:1) sipped intra-workout may modestly reduce perceived exertion and central fatigue; no clear muscle synthesis benefit.
- Older adult (60+): the PROT-AGE Study Group gives at least 1.0-1.2 g/kg/day total protein for people over 65, at least 1.2 g/kg/day for those who are active and 1.2-1.5 g/kg/day for most with acute or chronic disease (older people with severe kidney disease who are not on dialysis may need to limit protein); meals with at least 30 g of high-quality protein are used to overcome anabolic resistance. Leucine fortification (e.g., 2-3 g leucine added per meal) has been tested with mixed results (see the sarcopenia section above).
- Cirrhosis / hepatic encephalopathy: branched-chain amino acid-enriched formulas have been given under medical supervision (Marchesini protocol) at 0.25 g/kg/day branched-chain amino acid in 2:1:1 ratio, with an evening dose to maintain overnight nitrogen balance.
A varied diet that includes any combination of meat, fish, eggs, dairy, legumes, fermented soy (tempeh, natto, miso) or quinoa and reaches its total daily protein target supplies more than enough valine. Isolated valine supplements (sold as a standalone amino acid) have a role mainly in the management of inherited metabolic disorders.
Key Research Papers
- Harper AE, Benevenga NJ, Wohlhueter RM (1970). Effects of ingestion of disproportionate amounts of amino acids. Physiological Reviews. — PubMed PMID: 4912906
- Moberg M et al. (2016). Activation of mTORC1 by leucine is potentiated by branched-chain amino acids and even more so by essential amino acids following resistance exercise. American Journal of Physiology — Cell Physiology. — PubMed PMID: 27053525
- Wolfson RL et al. (2016). Sestrin2 is a leucine sensor for the mTORC1 pathway. Science. — PubMed PMID: 26449471
- Saxton RA et al. (2016). Structural basis for leucine sensing by the Sestrin2-mTORC1 pathway. Science. — PubMed PMID: 26586190
- Fouré A, Bendahan D (2017). Is branched-chain amino acids supplementation an efficient nutritional strategy to alleviate skeletal muscle damage? A systematic review. Nutrients. — PubMed PMID: 28934166
- Jackman SR et al. (2017). Branched-chain amino acid ingestion stimulates muscle myofibrillar protein synthesis following resistance exercise in humans. Frontiers in Physiology. — PubMed PMID: 28638350
- Jäger R et al. (2017). International Society of Sports Nutrition Position Stand: protein and exercise. Journal of the International Society of Sports Nutrition. — PubMed PMID: 28642676
- Plotkin DL et al. (2021). Isolated leucine and branched-chain amino acid supplementation for enhancing muscular strength and hypertrophy: a narrative review. International Journal of Sport Nutrition and Exercise Metabolism. — PubMed PMID: 33741748
- Wilkinson DJ et al. (2013). Effects of leucine and its metabolite beta-hydroxy-beta-methylbutyrate on human skeletal muscle protein metabolism. Journal of Physiology. — PubMed PMID: 23551944
- Drummond MJ, Rasmussen BB (2008). Leucine-enriched nutrients and the regulation of mammalian target of rapamycin signalling and human skeletal muscle protein synthesis. Current Opinion in Clinical Nutrition and Metabolic Care. — PubMed PMID: 18403916
- Phillips SM (2017). Current concepts and unresolved questions in dietary protein requirements and supplements in adults. Frontiers in Nutrition. — PubMed PMID: 28534027
- Wagenmakers AJ (1998). Muscle amino acid metabolism at rest and during exercise: role in human physiology and metabolism. Exercise and Sport Sciences Reviews. — PubMed PMID: 9696993
- Volpi E et al. (2003). Essential amino acids are primarily responsible for the amino acid stimulation of muscle protein anabolism in healthy elderly adults. American Journal of Clinical Nutrition. — PubMed PMID: 12885705
- Bauer J et al. (2013). Evidence-based recommendations for optimal dietary protein intake in older people: a position paper from the PROT-AGE Study Group. JAMDA. — PubMed PMID: 23867520
- Aamann L et al. (2026). Branched-chain amino acids for people with cirrhosis and hepatic encephalopathy. Cochrane Database of Systematic Reviews. — PubMed PMID: 41542879
- Marchesini G et al. (2003). Nutritional supplementation with branched-chain amino acids in advanced cirrhosis: a double-blind, randomized trial. Gastroenterology. — PubMed PMID: 12806613
PubMed Topic Searches
Connections
- All Amino Acids
- Valine Overview
- Valine Benefits Hub
- Valine for Energy Metabolism
- Valine for Cognitive Performance
- Valine for Nitrogen Balance & Wound Healing
- Leucine (Branched-Chain Amino Acid Partner)
- Isoleucine (Branched-Chain Amino Acid Partner)
- Glutamine
- Alanine
- Arginine
- Eggs
- Exercise
- Fatigue
- History
- Sources