⚠ Evidence warning: Clinical trials or other evidence do not support the claims that inadequate isoleucine drives nutritional anemia through lost hemoglobin synthesis, and that isoleucine triggers GLUT4 translocation and glucose entry into muscle without insulin receptor activation. This page keeps it as a report of what people, websites or other media say.
Isoleucine — Benefits Deep Dive
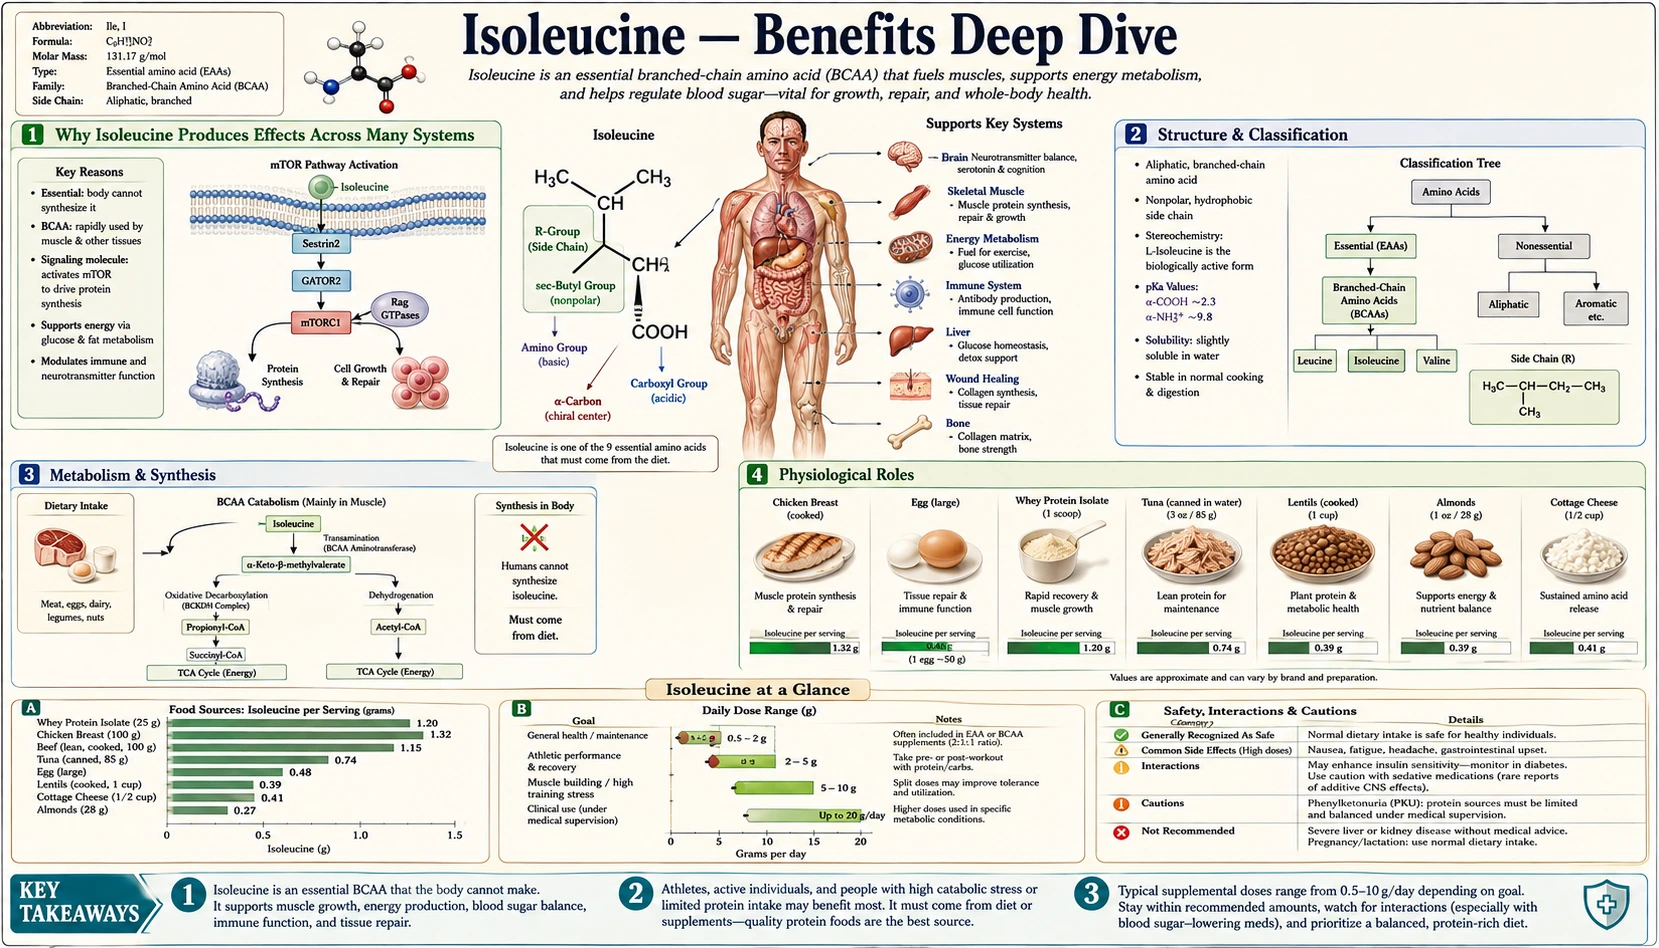
Isoleucine is one of three branched-chain amino acids (BCAAs) — alongside leucine and valine — and, in rat and muscle-cell studies, the one with the strongest insulin-independent glucose-uptake activity in skeletal muscle (leucine also raised glucose uptake in muscle cells, at higher concentrations). It is a structural isomer of leucine (same molecular formula, different arrangement of the side chain), but the two amino acids have distinct downstream effects: leucine is the dominant mTORC1 activator that turns on the protein synthesis machinery, while isoleucine is the dominant GLUT4 translocator that delivers glucose substrate to the working muscle. Four deep-dive pages below explore where isoleucine produces the most consequential clinical effects — muscle protein synthesis as part of the canonical 2:1:1 branched-chain amino acid (BCAA) trio, the Doi-and-Yoshizawa-characterized insulin-independent glucose uptake pathway with its complicated relationship to the branched-chain amino acid paradox in metabolic disease, the central-fatigue mechanism that underlies branched-chain amino acid use in endurance sport, and the unusual absence of isoleucine from adult human hemoglobin (fetal hemoglobin contains it) alongside the wound-healing protein-synthesis burst.
Deep-Dive Articles
Muscle Protein Synthesis
Isoleucine as one of three branched-chain amino acids (with leucine and valine) and the canonical 2:1:1 leucine:isoleucine:valine ratio in supplements. The division of labor between leucine's mechanistic target of rapamycin (mTOR) effect and isoleucine's GLUT4 effect — signal vs substrate. Why pure leucine supplementation underperforms full-spectrum branched-chain amino acids. Anti-catabolic effect during caloric restriction, sarcopenia and anabolic resistance in older adults, and the honest evidence summary on whether branched-chain amino acid supplementation adds anything to an already adequate dietary protein intake.
Read the deep dive →Glucose Uptake
The Doi & Yoshizawa research in rats and mouse muscle cells in the early 2000s showing isoleucine (without insulin) raises glucose uptake in muscle cells through phosphatidylinositol 3-kinase (PI3K) signaling. Fasted vs postprandial glucose dynamics, suppression of hepatic gluconeogenesis, the branched-chain amino acid paradox (elevated serum branched-chain amino acids in obesity and diabetes), the mTORC1-IRS-1 feedback loop that may make chronic high-dose branched-chain amino acids harmful, and what this means for practical glycemic management.
Read the deep dive →Endurance Performance
Branched-chain amino acids and central fatigue: the Newsholme tryptophan-serotonin hypothesis. How branched-chain amino acids compete with tryptophan for LAT1 transport across the blood-brain barrier, blunting brain serotonin synthesis and delaying the perception of fatigue in long-duration events. Pre-event, intra-event, and post-event branched-chain amino acid timing. The mixed meta-analysis evidence base — small but real benefit in long sub-maximal events, particularly in heat. Isoleucine's specific contribution via glucose uptake plus LAT1 competition.
Read the deep dive →Hemoglobin & Wound Healing
Isoleucine and hemoglobin — a 2026 preprint (not yet peer-reviewed) analysing 707 vertebrate genomes reports that adult human hemoglobin contains no isoleucine while fetal and embryonic hemoglobin do, and that the malaria parasite, which stops growing in adult red cells without outside isoleucine, grew without it in newborn cord-blood red cells. The broader heme protein family: myoglobin, cytochromes, catalase. Beta-defensin upregulation in epithelial innate immunity. The three phases of wound healing and their protein synthesis demands. Surgical, burn, and chronic wound applications including diabetic ulcers and pressure injuries.
Read the deep dive →Table of Contents
- Deep-Dive Articles
- Why Isoleucine Produces Effects Across Many Systems
- Research Papers: Muscle Protein Synthesis
- Research Papers: Glucose Uptake
- Research Papers: Endurance Performance
- Research Papers: Hemoglobin & Wound Healing
- Research Papers: Cross-Cutting (Mechanism, Status, Safety)
- External Authoritative Resources
- Connections
- Featured Videos
Why Isoleucine Produces Effects Across Many Systems
Most amino acids have one or two principal physiological roles — one or two enzyme cofactor positions, one or two structural positions in major proteins, or one or two neurotransmitter precursor functions. Isoleucine is unusual because it operates simultaneously at four conceptually distinct levels of physiology, and each level maps to a distinct category of clinical effect.
- Structural building block in skeletal muscle protein — the same protein-synthesis role as any other essential amino acid, but quantitatively more prominent because skeletal muscle is so abundant (the largest single tissue mass in most adults) and because isoleucine is enriched in the branched-chain amino acid-rich myofibrillar proteins (actin, myosin, troponin, tropomyosin, titin) that perform contraction. Loss of muscle through inadequate dietary isoleucine drives the sarcopenia and anti-catabolic clinical pictures. Loss of hemoglobin synthesis through inadequate isoleucine drives the amino-acid-limited nutritional anemia seen in severe protein-energy malnutrition. Hemoglobin is the exception: a 2026 preprint (not yet peer-reviewed) reports that the adult hemoglobin of humans and other non-Malagasy primates contains no isoleucine, while fetal and embryonic hemoglobin do.
- Signaling molecule for insulin-independent glucose uptake — the research of Doi, Yoshizawa, and colleagues established that isoleucine acts as a direct ligand input to PI3-kinase signaling in skeletal muscle, triggering GLUT4 translocation and glucose entry without requiring insulin receptor activation. In the research of Doi, Yoshizawa and colleagues, a single oral dose of isoleucine (0.3 g per kg of body weight) given to normal rats lowered blood sugar 30 and 60 minutes after a glucose drink, while the same dose of leucine or valine did not. In mouse muscle cells grown without insulin, 1 mM isoleucine raised glucose use by 16.8%; glucose uptake rose with 1–10 mM isoleucine and also with 5–10 mM leucine, and the isoleucine effect ran through phosphatidylinositol 3-kinase (PI3K) signaling (Doi 2003). These animal and cell findings are the proposed mechanism behind the acute glucose-lowering effect of fasted isoleucine and part of the rationale given for whey protein pre-loading before carbohydrate-containing meals in type 2 diabetes. What is not known is whether the same effect happens in people at the amounts found in food.
- Competitor at the blood-brain barrier LAT1 transporter — isoleucine, along with leucine and valine, competes with tryptophan for uptake into the brain. This is the molecular basis of the Newsholme central fatigue hypothesis and the rationale for branched-chain amino acid supplementation in long-duration endurance events. The competition is functional: shifting the branched-chain amino acid:tryptophan ratio in plasma demonstrably shifts brain serotonin synthesis in animal models.
- Oxidizable energy substrate during periods of negative energy balance — the branched-chain amino acids can be oxidized directly in skeletal muscle to produce adenosine triphosphate (ATP), bypassing the liver-centric metabolism of most other amino acids. This makes isoleucine a useful substrate during prolonged exercise, fasting, and caloric restriction, and underlies the anti-catabolic muscle-sparing effect.
The therapeutic complication is the branched-chain amino acid paradox: chronically elevated serum branched-chain amino acids are consistently associated with insulin resistance, obesity, and type 2 diabetes in cross-sectional epidemiology, and the elevation predicts future diabetes risk. The acute beneficial effect of isoleucine on glucose disposal coexists with apparent harm from chronic elevation. The proposed reconciliation involves the mTORC1-S6K1-IRS-1 feedback loop: chronic mTORC1 hyperactivation by sustained branched-chain amino acid elevation drives feedback inhibition of insulin receptor substrate 1, producing the very insulin resistance that the branched-chain amino acids were initially intended to bypass. This is the reasoning researchers give for favouring dietary isoleucine from whole protein sources (which deliver branched-chain amino acids in physiologic balance and physiologic quantity) over chronic high-dose isolated branched-chain amino acid supplementation in insulin-resistant people.
Mouse studies point at isoleucine itself. In a 2021 study, a low-isoleucine diet changed liver and fat metabolism in mice, raising liver insulin sensitivity and energy expenditure; cutting valine had similar but smaller effects, and cutting leucine had none. Reducing isoleucine or valine quickly restored metabolic health in mice made obese by diet, and in a human population study, differences in dietary isoleucine helped explain differences in body mass index (Yu 2021). In a 2023 study in genetically diverse mice, a diet low in isoleucine made both young and old mice leaner with better blood-sugar control, reduced frailty, and lengthened life in both sexes, more so in males (Green 2023). These are mouse results; restricting isoleucine has not been tested in this way in people.
The settings where isolated branched-chain amino acid or isoleucine supplementation has been studied are acute pre-event support in long endurance events, post-bariatric surgical recovery, specific clinical protocols (hepatic encephalopathy and burn protein support in hospital care), and older adults with sarcopenia who cannot meet protein needs through food alone. Outside these settings, a varied diet with adequate complete protein from a mix of animal and plant sources supplies isoleucine for all four of the mechanistic categories above.
Research Papers: Muscle Protein Synthesis
- Doi M, Yamaoka I, Fukunaga T, Nakayama M (2003). Isoleucine, a potent plasma glucose-lowering amino acid, stimulates glucose uptake in C2C12 myotubes. Biochemical and Biophysical Research Communications 312(4):1111-7 — PubMed PMID: 14651987
- Anthony JC et al. (2000). Orally administered leucine stimulates protein synthesis in skeletal muscle of postabsorptive rats — PubMed: Anthony 2000
- Wolfe RR (2017). Branched-chain amino acids and muscle protein synthesis in humans: myth or reality? — PubMed: Wolfe 2017
- Jackman SR et al. (2017). BCAA ingestion stimulates myofibrillar protein synthesis following resistance exercise — PubMed: Jackman 2017
- Wolfson RL et al. (2016). Sestrin2 is a leucine sensor for the mTORC1 pathway — PubMed: Wolfson 2016
- Kimball SR, Jefferson LS (2006). Signaling pathways for BCAA translational control — PubMed: Kimball 2006
- Bauer J et al. (2013). PROT-AGE position paper on dietary protein for older people — PubMed: Bauer PROT-AGE 2013
- Phillips SM (2014). Brief review of critical processes in exercise-induced muscular hypertrophy — PubMed: Phillips 2014
- Plotkin DL et al. (2021). Isolated leucine and BCAA supplementation for muscular strength — PubMed: Plotkin 2021
- Churchward-Venne TA et al. (2014). Leucine supplementation enhances myofibrillar protein synthesis — PubMed: Churchward-Venne 2014
Research Papers: Glucose Uptake
- Doi M, Yamaoka I, Nakayama M, Sugahara K, Yoshizawa F (2007). Hypoglycemic effect of isoleucine involves increased muscle glucose uptake and whole body glucose oxidation and decreased hepatic gluconeogenesis. American Journal of Physiology. Endocrinology and Metabolism 292(6):E1683-93 — PubMed PMID: 17299083
- Yoshizawa F (2012). New therapeutic strategy for amino acid medicine — PubMed: Yoshizawa 2012
- Newgard CB et al. (2009). BCAA-related metabolic signature in obesity and insulin resistance — PubMed: Newgard 2009
- Wang TJ et al. (2011). Metabolite profiles and risk of developing diabetes — PubMed: Wang 2011
- Lynch CJ, Adams SH (2014). BCAAs in metabolic signalling and insulin resistance — PubMed: Lynch & Adams 2014
- Felig P, Marliss E, Cahill GF (1969). Plasma amino acid levels and insulin secretion in obesity — PubMed: Felig 1969
- Pal S et al. (2010). Whey protein isolate effects on body composition and glucose — PubMed: Pal 2010
- Cummings NE et al. (2018). Restoration of metabolic health by decreased BCAA consumption — PubMed: Cummings 2018
- Tremblay F et al. (2007). IRS-1 Ser-1101 as S6K1 target in nutrient-induced insulin resistance — PubMed: Tremblay 2007
- Shou J, Chen PJ, Xiao WH (2020). Mechanism of increased risk of insulin resistance in aging skeletal muscle. Diabetology & Metabolic Syndrome 12:14 — PubMed PMID: 32082422
- Yu D, Richardson NE, Green CL, et al. (2021). The adverse metabolic effects of branched-chain amino acids are mediated by isoleucine and valine. Cell Metabolism 33(5):905-922.e6 — PubMed PMID: 33887198
- Green CL, Trautman ME, Chaiyakul K, et al. (2023). Dietary restriction of isoleucine increases healthspan and lifespan of genetically heterogeneous mice. Cell Metabolism 35(11):1976-1995.e6 — PubMed PMID: 37939658
Research Papers: Endurance Performance
- Blomstrand E (2001). Amino acids and central fatigue — PubMed: Blomstrand 2001
- Blomstrand E et al. (1991). BCAA administration during sustained exercise — PubMed: Blomstrand 1991
- Davis JM, Bailey SP (1997). Possible mechanisms of CNS fatigue during exercise — PubMed: Davis & Bailey 1997
- Mittleman KD et al. (1998). BCAAs prolong exercise during heat stress — PubMed: Mittleman 1998
- Fernstrom JD (2005). BCAAs and brain function — PubMed: Fernstrom 2005
- Meeusen R, Watson P (2007). Amino acids and the brain in central fatigue — PubMed: Meeusen 2007
- Gualano AB et al. (2011). BCAA supplementation and exercise capacity after glycogen depletion — PubMed: Gualano 2011
- Rahimi MH et al. (2017). BCAA supplementation and exercise-induced muscle damage meta-analysis — PubMed: Rahimi 2017
- AbuMoh'd MF et al. (2020). BCAA effects on muscular and central fatigue — PubMed: AbuMoh'd 2020
Research Papers: Hemoglobin & Wound Healing
- Perutz MF et al. (1960). Structure of haemoglobin: three-dimensional Fourier synthesis — PubMed: Perutz 1960
- Schroeder WA et al. (1967). Amino acid sequence of bovine fetal haemoglobin alpha-chain — PubMed: Schroeder 1967
- Demling RH (2009). Nutrition, anabolism, and the wound healing process — PubMed: Demling 2009
- Stechmiller JK (2010). Nutrition and wound healing — PubMed: Stechmiller 2010
- Posthauer ME et al. (2015). Nutrition for pressure ulcer management — PubMed: Posthauer 2015
- Williams JZ et al. (2002). Specialized amino acid mixture for human collagen deposition — PubMed: Williams 2002
- De Bandt JP, Cynober L (2006). BCAA use in burn, trauma, and sepsis — PubMed: De Bandt & Cynober 2006
- Bevins CL, Salzman NH (2011). Paneth cells and antimicrobial peptides in intestinal homeostasis — PubMed: Bevins & Salzman 2011
- Sunkara LT et al. (2011). Butyrate enhances antimicrobial host defense peptide expression — PubMed: Sunkara 2011
- Wernerman J et al. (1990). Alpha-ketoglutarate and postoperative muscle catabolism — PubMed: Wernerman 1990
- Houri-Zeevi L, Kampmann M, Duraisingh MT, Vosshall LB (2026). Isoleucine absence from adult human hemoglobin is mirrored in mosquito proteomes and limits malaria parasite growth. bioRxiv (preprint, not peer-reviewed), doi:10.64898/2026.09.23.753855 — PubMed PMID: 42818369
Research Papers: Cross-Cutting (Mechanism, Status, Safety)
- Harper AE, Miller RH, Block KP (1984). Branched-chain amino acid metabolism (Annual Review) — PubMed: Harper Annual Review 1984
- Brosnan JT, Brosnan ME (2006). Branched-chain amino acids: enzyme and substrate regulation — PubMed: Brosnan 2006
- Shimomura Y et al. (2006). Exercise promotes BCAA catabolism — PubMed: Shimomura 2006
- Holecek M (2018). Branched-chain amino acids in health and disease — PubMed: Holecek 2018
- WHO/FAO/UNU (2007). Protein and amino acid requirements in human nutrition — PubMed: WHO/FAO/UNU 2007
- Strauss KA, Puffenberger EG, Morton DH (2013). Maple syrup urine disease (GeneReviews) — PubMed: MSUD GeneReviews
- Marchesini G et al. (2003). BCAAs in the treatment of chronic hepatic encephalopathy — PubMed: Marchesini 2003
- Fernstrom JD (2013). Large neutral amino acids: dietary effects on brain neurochemistry and function — PubMed: Fernstrom 2013
- Phillips SM et al. (2016). Protein "requirements" beyond the RDA for older adults — PubMed: Phillips 2016
- Smith K et al. (1992). Flooding with L-[1-13C]leucine stimulates muscle protein synthesis — PubMed: Smith 1992
External Authoritative Resources
- U.S. National Institutes of Health (NIH) Office of Dietary Supplements — Dietary Supplements for Exercise and Athletic Performance — the most authoritative scientific summary of branched-chain amino acid biology, regularly updated
- U.S. National Institutes of Health Office of Dietary Supplements — All Fact Sheets (includes dietary protein and amino acid coverage)
- WHO — Protein and Amino Acid Requirements in Human Nutrition (Technical Report 935)
- U.S. National Institutes of Health Office of Dietary Supplements — Dietary Supplements for Exercise and Athletic Performance
- PubMed — All research on Isoleucine
Connections
- All Amino Acids
- Isoleucine (Main Page)
- Isoleucine for Muscle Protein Synthesis
- Isoleucine for Glucose Uptake
- Isoleucine for Endurance Performance
- Isoleucine for Hemoglobin & Wound Healing
- Leucine
- Valine
- Tryptophan
- Tyrosine
- Phenylalanine
- Insulin Resistance
- Metabolic Syndrome
- Anemia
- Fatigue
- Iron
- Zinc
- Vitamin C
- Eggs
- Blood Sugar
- History
- Sources